

256
Andrew CLARKE
has been glacial history. Periodic extensions of the
continental ice sheets at previous glacial maxima will
have covered large areas of the continental shelf, and
forced the fauna to move into the deeper waters of the
continental slope or become locally extinct (Clarke and
Crame, 1989; Brey et al., 1996). Such extensions and
retractions of the ice sheet are likely to have been a
powerful evolutionary forcing mechanism, driving both
speciation and extensive exchange between shelf, slope
and possibly even abyssal faunas (Clarke and Crame,
1989). A critical point, as yet unresolved, is whether
previous glacial maxima ever resulted in a complete
eradication of continental shelf habitat. Glaciological
and geophysical evidence currently remains equivocal,
although Brandt (1991, 1992) concluded from her
phylogenetic analysis of the Southern Ocean isopod
fauna that some shallow water refugia always remained
colonised.
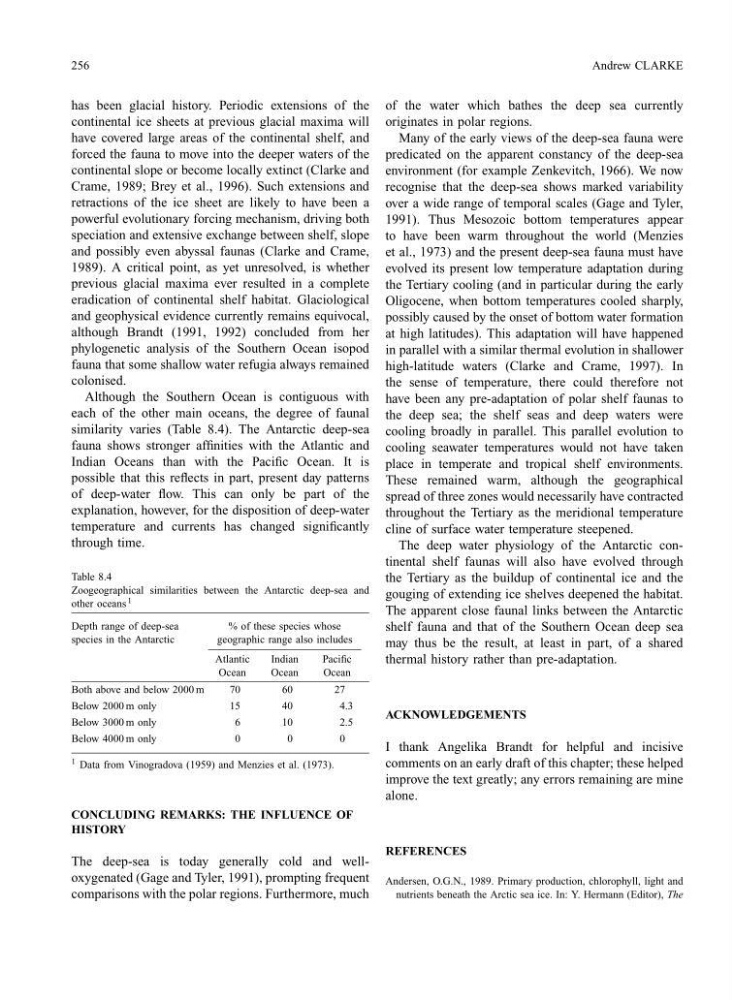
Although the Southern Ocean is contiguous with
each of the other main oceans, the degree of faunal
similarity varies (Table 8.4). The Antarctic deep-sea
fauna shows stronger affinities with the Atlantic and
Indian Oceans than with the Pacific Ocean. It is
possible that this reflects in part, present day patterns
of deep-water flow. This can only be part of the
explanation, however, for the disposition of deep-water
temperature and currents has changed significantly
through time.
Table 8.4
Zoogeographical similarities between the Antarctic deep-sea and
other oceans 1
Depth range of deep-sea
species in the Antarctic
% of these species whose
geographic range also includes
Atlantic
Ocean
Indian
Ocean
Pacific
Ocean
Both above and below 2000 m
70
60
27
Below 2000 m only
15
40
4.3
Below 3000 m only
6
10
2.5
Below 4000 m only
0
0
0
1 Data from Vinogradova (1959) and Menzies et al. (1973).
CONCLUDING REMARKS: THE INFLUENCE OF
HISTORY
The deep-sea is today generally cold and welloxygenated (Gage and Tyler, 1991), prompting frequent
comparisons with the polar regions. Furthermore, much
of the water which bathes the deep sea currently
originates in polar regions.
Many of the early views of the deep-sea fauna were
predicated on the apparent constancy of the deep-sea
environment (for example Zenkevitch, 1966). We now
recognise that the deep-sea shows marked variability
over a wide range of temporal scales (Gage and Tyler,
1991). Thus Mesozoic bottom temperatures appear
to have been warm throughout the world (Menzies
et al., 1973) and the present deep-sea fauna must have
evolved its present low temperature adaptation during
the Tertiary cooling (and in particular during the early
Oligocene, when bottom temperatures cooled sharply,
possibly caused by the onset of bottom water formation
at high latitudes). This adaptation will have happened
in parallel with a similar thermal evolution in shallower
high-latitude waters (Clarke and Crame, 1997). In
the sense of temperature, there could therefore not
have been any pre-adaptation of polar shelf faunas to
the deep sea; the shelf seas and deep waters were
cooling broadly in parallel. This parallel evolution to
cooling seawater temperatures would not have taken
place in temperate and tropical shelf environments.
These remained warm, although the geographical
spread of three zones would necessarily have contracted
throughout the Tertiary as the meridional temperature
cline of surface water temperature steepened.
The deep water physiology of the Antarctic continental shelf faunas will also have evolved through
the Tertiary as the buildup of continental ice and the
gouging of extending ice shelves deepened the habitat.
The apparent close faunal links between the Antarctic
shelf fauna and that of the Southern Ocean deep sea
may thus be the result, at least in part, of a shared
thermal history rather than pre-adaptation.
ACKNOWLEDGEMENTS
I thank Angelika Brandt for helpful and incisive
comments on an early draft of this chapter; these helped
improve the text greatly; any errors remaining are mine
alone.
REFERENCES
Andersen, O.G.N., 1989. Primary production, chlorophyll, light and
nutrients beneath the Arctic sea ice. In: Y. Hermann (Editor), The