

Chapter 20 Grazing in Seagrass Ecosystems
475
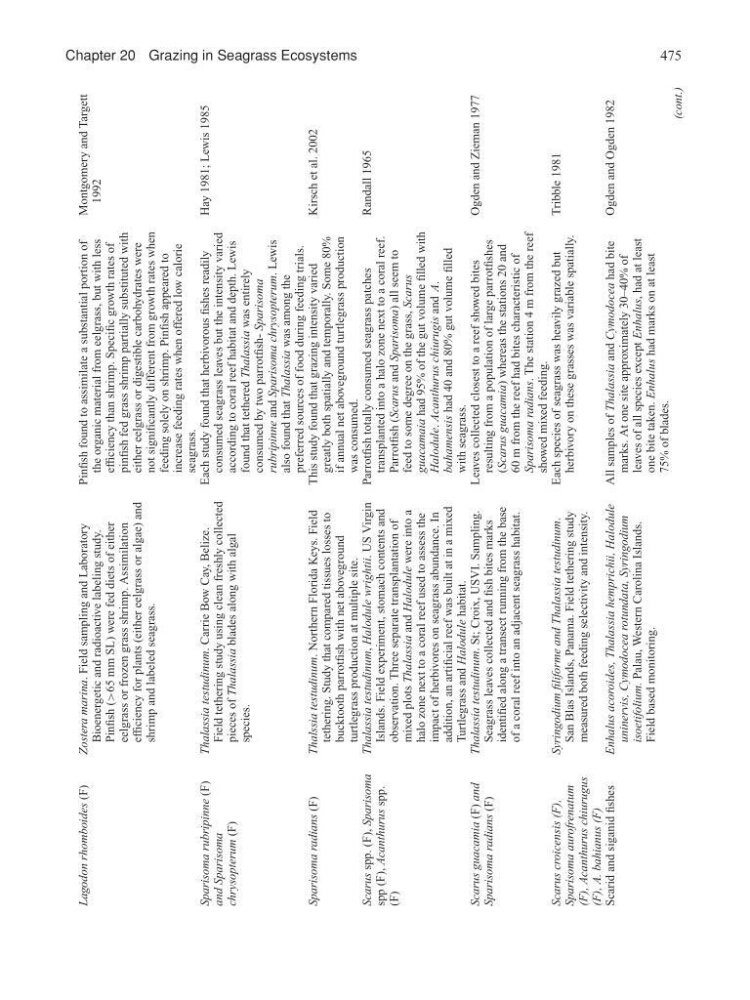
Lagodon rhomboides (F)
Zostera marina. Field sampling and Laboratory
Bioenergetic and radioactive labeling study.
Pinfish (>65 mm SL) were fed diets of either
eelgrass or frozen grass shrimp. Assimilation
efficiency for plants (either eelgrass or algae) and
shrimp and labeled seagrass.
Pinfish found to assimilate a substantial portion of
the organic material from eelgrass, but with less
efficiency than shrimp. Specific growth rates of
pinfish fed grass shrimp partially substituted with
either eelgrass or digestible carbohydrates were
not significantly different from growth rates when
feeding solely on shrimp. Pinfish appeared to
increase feeding rates when offered low calorie
seagrass.
Montgomery and Targett
1992
Sparisoma rubripinne (F)
and Sparisoma
chrysopterum (F)
Thalassia testudinum. Carrie Bow Cay, Belize.
Field tethering study using clean freshly collected
pieces of Thalassia blades along with algal
species.
Each study found that herbivorous fishes readily
consumed seagrass leaves but the intensity varied
according to coral reef habitat and depth. Lewis
found that tethered Thalassia was entirely
consumed by two parrotfish- Sparisoma
rubripinne and Sparisoma chrysopterum. Lewis
also found that Thalassia was among the
preferred sources of food during feeding trials.
Hay 1981; Lewis 1985
Sparisoma radians (F)
Thalssia testudinum. Northern Florida Keys. Field
tethering. Study that compared tissues losses to
bucktooth parrotfish with net aboveground
turtlegrass production at multiple site.
This study found that grazing intensity varied
greatly both spatially and temporally. Some 80%
if annual net aboveground turtlegrass production
was consumed.
Kirsch et al. 2002
Scarus spp. (F), Sparisoma
spp (F), Acanthurus spp.
(F)
Thalassia testudinum, Halodule wrightii. US Virgin
Islands. Field experiment, stomach contents and
observation. Three separate transplantation of
mixed plots Thalassia and Halodule were into a
halo zone next to a coral reef used to assess the
impact of herbivores on seagrass abundance. In
addition, an artificial reef was built at in a mixed
Turtlegrass and Halodule habitat.
Parrotfish totally consumed seagrass patches
transplanted into a halo zone next to a coral reef.
Parrotfish (Scarus and Sparisoma) all seem to
feed to some degree on the grass, Scarus
guacamaia had 95% of the gut volume filled with
Halodule. Acanthurus chiurugis and A.
bahamensis had 40 and 80% gut volume filled
with seagrass.
Randall 1965
Scarus guacamia (F) and
Sparisoma radians (F)
Thalassia testudinum. St; Croix, USVI. Sampling.
Seagrass leaves collected and fish bites marks
identified along a transect running from the base
of a coral reef into an adjacent seagrass habitat.
Leaves collected closest to a reef showed bites
resulting from a population of large parrotfishes
(Scarus guacamia) whereas the stations 20 and
60 m from the reef had bites characteristic of
Sparisoma radians. The station 4 m from the reef
showed mixed feeding.
Ogden and Zieman 1977
Scarus croicensis (F),
Sparisoma aurofrenatum
(F), Acanthurus chiurugus
(F), A. bahianus (F)
Syringodium filiforme and Thalassia testudinum.
San Blas Islands, Panama. Field tethering study
measured both feeding selectivity and intensity.
Each species of seagrass was heavily grazed but
herbivory on these grasses was variable spatially.
Tribble 1981
Scarid and siganid fishes
Enhalus acoroides, Thalassia hemprichii, Halodule
uninervis, Cymodocea rotundata, Syringodium
isoetifolium. Palau, Western Carolina Islands.
Field based monitoring.
All samples of Thalassia and Cymodocea had bite
marks. At one site approximately 30–40% of
leaves of all species except Enhalus, had at least
one bite taken. Enhalus had marks on at least
75% of blades.
Ogden and Ogden 1982
(cont.)