

7.3 Landscape Networks
Percolation theory combined with graph models is a powerful step forward
for landscape ecology. However, these models do not, as of yet, directly represent or reflect rates of dispersal among patches. An extension of these
models is to include rates of movement among patches in the landscape.
I call these landscape network models. A landscape network is a mathematical description of the functional relationships between landscape
components, be they habitat patches, river segments, an agricultural mosaic,
or any other subdivision of a landscape that can be defined. The focus of
a landscape network model is flow of energy, materials, and information
from one component to another. Typically these “components” will be
discrete habitat patches, and we are interested in the flux of individuals
moving between different patches. We could subdivide the landscape
into a continuum of points or perhaps into different habitat categories
rather than patches. For example, we might be interested in modeling the
movement of amphibians between aquatic and terrestrial habitat types.
Here, however, I focus on spatial landscape networks with discrete habitat
patches.
To begin with, imagine a scenario in which a landscape is subdivided into
a set of subregions. These subregions could be arbitrarily defined “cells”
in a grid or could be defined to map onto existing habitat patches. Let us
constrain this subdivision so that every point in the landscape falls within
one and only one subdivision. A typical scenario is an archipelago of forest
fragments embedded in a cleared, nonforest matrix. If we are interested
in modeling the movement of a given species in relation to these habitat
fragments, then the quantity of interest is the number of individuals that
move between any given pair of fragments over some period of time, say
a single generation. To do this, we need to label all the fragments. Let s 0
represent the nonforest matrix and s 1 ,s 2 ,s 3 , . . . , s N represent the N forest
fragments. Given that dispersal among patches may be rare, it is appropriate to model these events as a stochastic process. In the simplest model,
we need to know three things: (1) the probability of dispersing a distance
x, (2) the probability that in leaving patch i we end up in patch j, and
(3) the probability that we were in patch i to begin with. Dispersal data
for many organisms [e.g., Kot et al. (1996)] indicate the probability of
dispersing a given distance is often best fit by a function that decays as
a power law in the tails. However, other functions may be appropriate,
depending on the dispersal mode and life history of the organism modeled.
If we assume that the organism disperses in a random direction and travels
distance x, then the probability of moving from patch i to patch j, given that
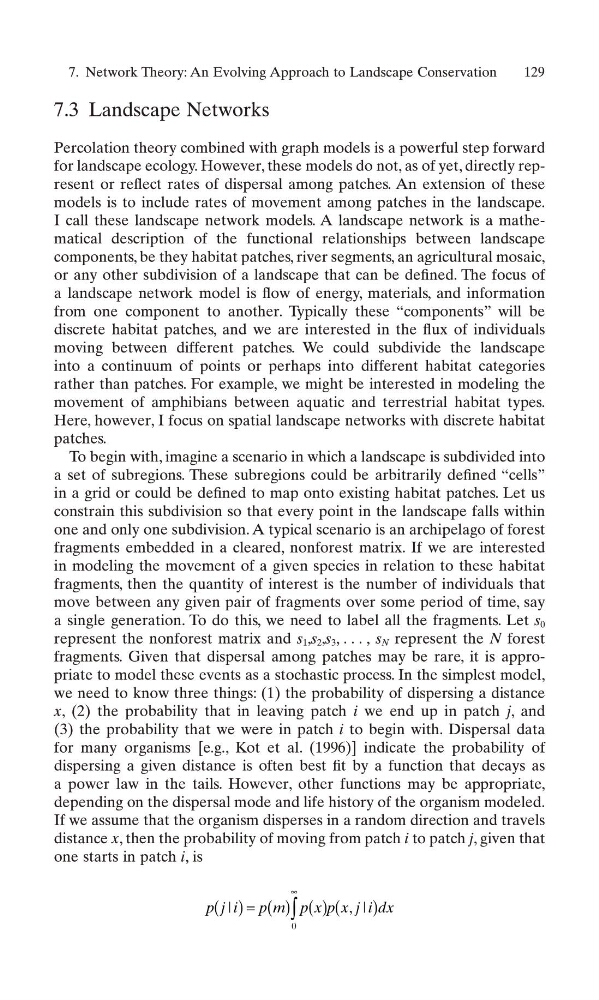
one starts in patch i, is
p j i p m p x p x j i dx
|
,|
( )= ( ) ( ) (
)
∞
∫
0
7. Network Theory: An Evolving Approach to Landscape Conservation
129