

11.3 Mechanics of Animal Swimming
361
likely the only mechanism they use actively, otherwise they are passive swimmers. On the other extreme, there are large animals, powerful enough to swim
independently by developing a thrust to overcome the drag forces.
Let us now be more specific and restrict our attention to one species, for
example, rainbow trout of different lengths, swimming in a flume tank.
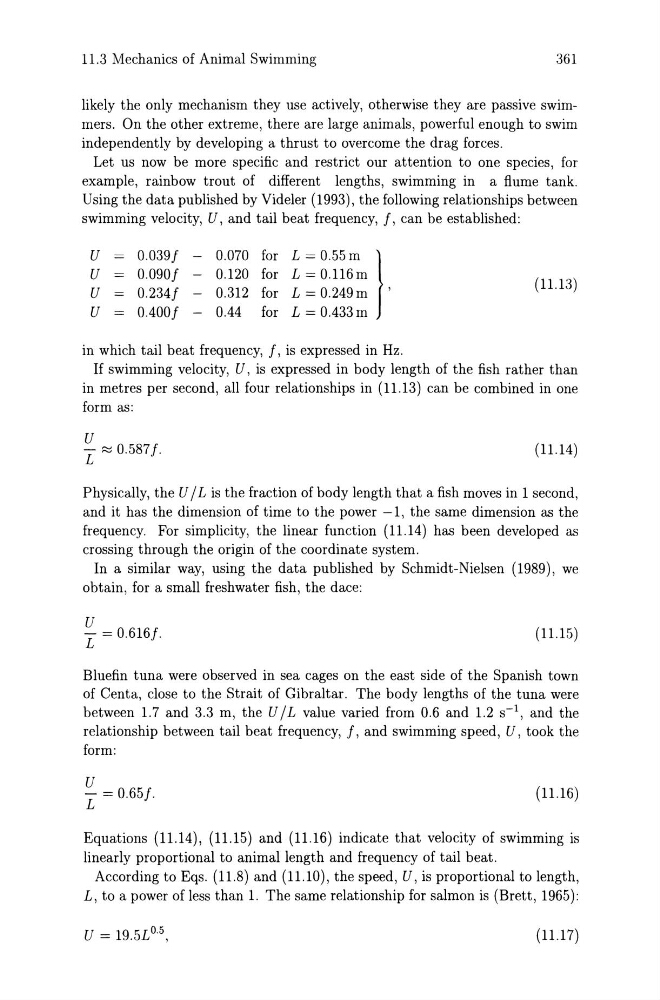
Using the data published by Videler (1993), the following relationships between
swimming velocity, U, and tail beat frequency, 1, can be established:
U = 0.0391 - 0.070 for L = 0.55 m }
U = 0.0901 - 0.120 for L=0.116m
U = 0.2341
0.312 for L = 0.249 m '
U = 0.4001 - 0.44 for L = 0.433 m
in which tail beat frequency, 1, is expressed in Hz.
(11.13)
If swimming velocity, U, is expressed in body length of the fish rather than
in metres per second, all four relationships in (11.13) can be combined in one
form as:
U
L ~ 0.587f.
(11.14)
Physically, the U / L is the fraction of body length that a fish moves in 1 second,
and it has the dimension of time to the power -1, the same dimension as the
frequency. For simplicity, the linear function (11.14) has been developed as
crossing through the origin of the coordinate system.
In a similar way, using the data published by Schmidt-Nielsen (1989), we
obtain, for a small freshwater fish, the dace:
U
L = 0.616f.
(11.15)
Bluefin tuna were observed in sea cages on the east side of the Spanish town
of Centa, close to the Strait of Gibraltar. The body lengths of the tuna were
between 1.7 and 3.3 m, the U / L value varied from 0.6 and 1.2 s-l, and the
relationship between tail beat frequency, 1, and swimming speed, U, took the
form:
U
L = 0.65f.
(11.16)
Equations (11.14), (11.15) and (11.16) indicate that velocity of swimming is
linearly proportional to animal length and frequency of tail beat.
According to Eqs. (11.8) and (11.10), the speed, U, is proportional to length,
L, to a power of less than 1. The same relationship for salmon is (Brett, 1965):
(11.17)