

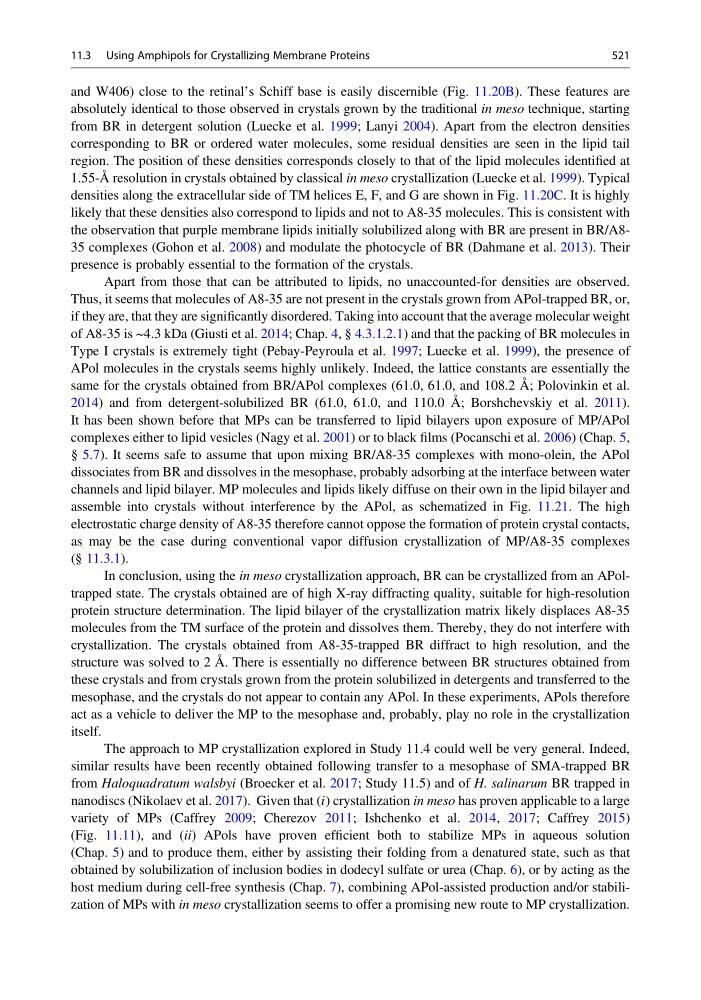
and W406) close to the retinal’s Schiff base is easily discernible (Fig. 11.20B). These features are
absolutely identical to those observed in crystals grown by the traditional in meso technique, starting
from BR in detergent solution (Luecke et al. 1999; Lanyi 2004). Apart from the electron densities
corresponding to BR or ordered water molecules, some residual densities are seen in the lipid tail
region. The position of these densities corresponds closely to that of the lipid molecules identified at
1.55-Å resolution in crystals obtained by classical in meso crystallization (Luecke et al. 1999). Typical
densities along the extracellular side of TM helices E, F, and G are shown in Fig. 11.20C. It is highly
likely that these densities also correspond to lipids and not to A8-35 molecules. This is consistent with
the observation that purple membrane lipids initially solubilized along with BR are present in BR/A835 complexes (Gohon et al. 2008) and modulate the photocycle of BR (Dahmane et al. 2013). Their
presence is probably essential to the formation of the crystals.
Apart from those that can be attributed to lipids, no unaccounted-for densities are observed.
Thus, it seems that molecules of A8-35 are not present in the crystals grown from APol-trapped BR, or,
if they are, that they are significantly disordered. Taking into account that the average molecular weight
of A8-35 is ~4.3 kDa (Giusti et al. 2014; Chap. 4, § 4.3.1.2.1) and that the packing of BR molecules in
Type I crystals is extremely tight (Pebay-Peyroula et al. 1997; Luecke et al. 1999), the presence of
APol molecules in the crystals seems highly unlikely. Indeed, the lattice constants are essentially the
same for the crystals obtained from BR/APol complexes (61.0, 61.0, and 108.2 Å; Polovinkin et al.
2014) and from detergent-solubilized BR (61.0, 61.0, and 110.0 Å; Borshchevskiy et al. 2011).
It has been shown before that MPs can be transferred to lipid bilayers upon exposure of MP/APol
complexes either to lipid vesicles (Nagy et al. 2001) or to black films (Pocanschi et al. 2006) (Chap. 5,
§ 5.7). It seems safe to assume that upon mixing BR/A8-35 complexes with mono-olein, the APol
dissociates from BR and dissolves in the mesophase, probably adsorbing at the interface between water
channels and lipid bilayer. MP molecules and lipids likely diffuse on their own in the lipid bilayer and
assemble into crystals without interference by the APol, as schematized in Fig. 11.21. The high
electrostatic charge density of A8-35 therefore cannot oppose the formation of protein crystal contacts,
as may be the case during conventional vapor diffusion crystallization of MP/A8-35 complexes
(§ 11.3.1).
In conclusion, using the in meso crystallization approach, BR can be crystallized from an APoltrapped state. The crystals obtained are of high X-ray diffracting quality, suitable for high-resolution
protein structure determination. The lipid bilayer of the crystallization matrix likely displaces A8-35
molecules from the TM surface of the protein and dissolves them. Thereby, they do not interfere with
crystallization. The crystals obtained from A8-35-trapped BR diffract to high resolution, and the
structure was solved to 2 Å. There is essentially no difference between BR structures obtained from
these crystals and from crystals grown from the protein solubilized in detergents and transferred to the
mesophase, and the crystals do not appear to contain any APol. In these experiments, APols therefore
act as a vehicle to deliver the MP to the mesophase and, probably, play no role in the crystallization
itself.
The approach to MP crystallization explored in Study 11.4 could well be very general. Indeed,
similar results have been recently obtained following transfer to a mesophase of SMA-trapped BR
from Haloquadratum walsbyi (Broecker et al. 2017; Study 11.5) and of H. salinarum BR trapped in
nanodiscs (Nikolaev et al. 2017). Given that (i) crystallization in meso has proven applicable to a large
variety of MPs (Caffrey 2009; Cherezov 2011; Ishchenko et al. 2014, 2017; Caffrey 2015)
(Fig. 11.11), and (ii) APols have proven efficient both to stabilize MPs in aqueous solution
(Chap. 5) and to produce them, either by assisting their folding from a denatured state, such as that
obtained by solubilization of inclusion bodies in dodecyl sulfate or urea (Chap. 6), or by acting as the
host medium during cell-free synthesis (Chap. 7), combining APol-assisted production and/or stabilization of MPs with in meso crystallization seems to offer a promising new route to MP crystallization.
11.3 Using Amphipols for Crystallizing Membrane Proteins
521