

5.3.1
Particle Composition
Purple membrane solubilized with OTG was ultracentrifuged. The supernatant was supplemented with
either unlabeled, deuterated, or tritiated A8-35 and the detergent removed by adsorption onto
Bio-Beads. The composition of the resulting BR/A8-35 particles was studied by (i) lipid analysis,
(ii) measurement of the content in [
3 H]A8-35, (iii) spectrophotometric determination of the content in
native and total protein, and (iv) determination by SEC, SANS, and AUC of the contrast match point,
mass, size, shape, and density of the particles. These properties depend on the mass of each constituent
present in the particles and provide internal controls as to the consistency of the measurements (Gohon
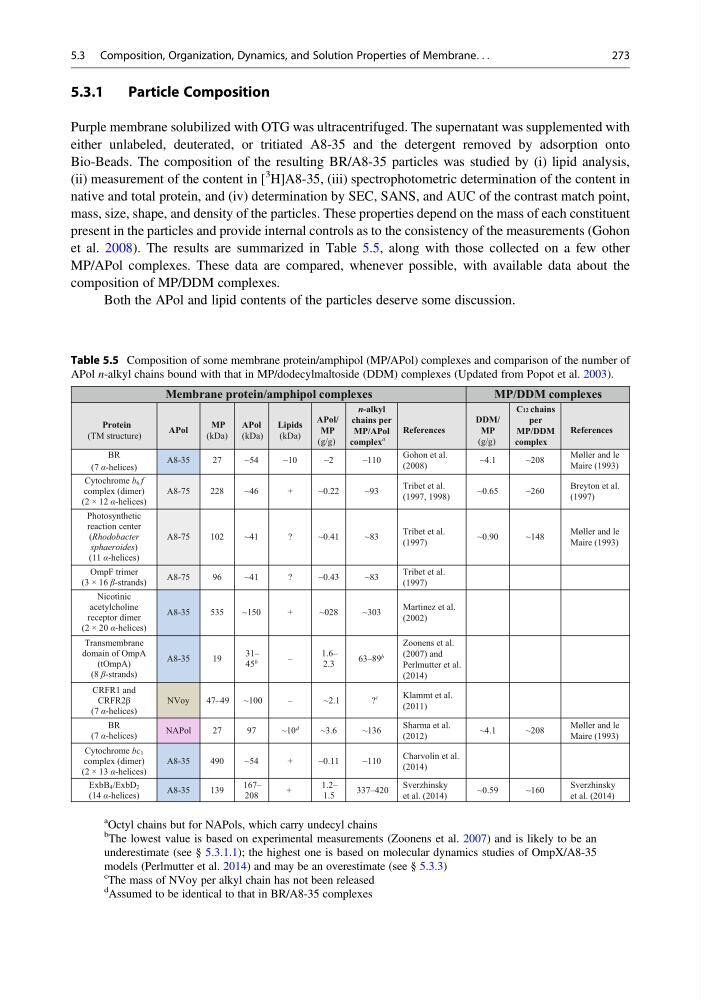
et al. 2008). The results are summarized in Table 5.5, along with those collected on a few other
MP/APol complexes. These data are compared, whenever possible, with available data about the
composition of MP/DDM complexes.
Both the APol and lipid contents of the particles deserve some discussion.
Table 5.5 Composition of some membrane protein/amphipol (MP/APol) complexes and comparison of the number of
APol n-alkyl chains bound with that in MP/dodecylmaltoside (DDM) complexes (Updated from Popot et al. 2003).
Membrane protein/amphipol complexes
MP/DDM complexes
Protein
(TM structure)
APol
MP
(kDa)
APol
(kDa)
Lipids
(kDa)
APol/
MP
(g/g)
n-alkyl
chains per
MP/APol
complex
a
References
DDM/
MP
(g/g)
C12 chains
per
MP/DDM
complex
References
BR
(7 α-helices)
A8-35
27
~54
~10
~2
~110
Gohon et al.
(2008)
~4.1
~208
Møller and le
Maire (1993)
Cytochrome b6 f
complex (dimer)
(2 × 12 α-helices)
A8-75
228
~46
+
~0.22
~93
Tribet et al.
(1997, 1998)
~0.65
~260
Breyton et al.
(1997)
Photosynthetic
reaction center
(Rhodobacter
sphaeroides)
(11 α-helices)
A8-75
102
~41
?
~0.41
~83
Tribet et al.
(1997)
~0.90
~148
Møller and le
Maire (1993)
OmpF trimer
(3 × 16 β-strands)
A8-75
96
~41
?
~0.43
~83
Tribet et al.
(1997)
Nicotinic
acetylcholine
receptor dimer
(2 × 20 α-helices)
A8-35
535
~150
+
~028
~303
Martinez et al.
(2002)
Transmembrane
domain of OmpA
(tOmpA)
(8 β-strands)
A8-35
19
31–
45
b
–
1.6–
2.3
63–89
b
Zoonens et al.
(2007) and
Perlmutter et al.
(2014)
CRFR1 and
CRFR2β
(7 α-helices)
NVoy
47–49
~100
–
~2.1
?
c
Klammt et al.
(2011)
BR
(7 α-helices)
NAPol
27
97
~10
d
~3.6
~136
Sharma et al.
(2012)
~4.1
~208
Møller and le
Maire (1993)
Cytochrome bc1
complex (dimer)
(2 × 13 α-helices)
A8-35
490
~54
+
~0.11
~110
Charvolin et al.
(2014)
ExbB4/ExbD2
(14 α-helices)
A8-35
139
167–
208
+
1.2–
1.5
337–420
Sverzhinsky
et al. (2014)
~0.59
~160
Sverzhinsky
et al. (2014)
a Octyl chains but for NAPols, which carry undecyl chains
b
The lowest value is based on experimental measurements (Zoonens et al. 2007) and is likely to be an
underestimate (see § 5.3.1.1); the highest one is based on molecular dynamics studies of OmpX/A8-35
models (Perlmutter et al. 2014) and may be an overestimate (see § 5.3.3)
c The mass of NVoy per alkyl chain has not been released
d
Assumed to be identical to that in BR/A8-35 complexes
5.3 Composition, Organization, Dynamics, and Solution Properties of Membrane. . .
273