

regression line should be forced to go through the point defined by
isosmotic volume at isosmolality. However, we show in [45] that
this argument is invalid on theoretical and statistical grounds and
has the potential to introduce errors. This being said, the validity of
the assumption that cells behave as linear osmometers is an ongoing
question in the literature. Some cells undergo both osmolyte and
surface area regulation in response to osmotic challenges [6], cells
regulate their permeability to water and solutes [46], and the
cytoskeleton-membrane complex or cell wall can allow cells to
withstand nontrivial transmembrane pressure differences
[47]. These features have been mostly neglected in the cryobiological literature, save, to our knowledge, Casula et al. [46] who study
the effects of stretch activated membrane proteins on the Boyle
van ’t Hoff relationship and its relevance to cryoprotectant equilibration protocols.
2.3 Osmolality
and Chemical Potential
In most physiologic literature, the approximation of the osmolality
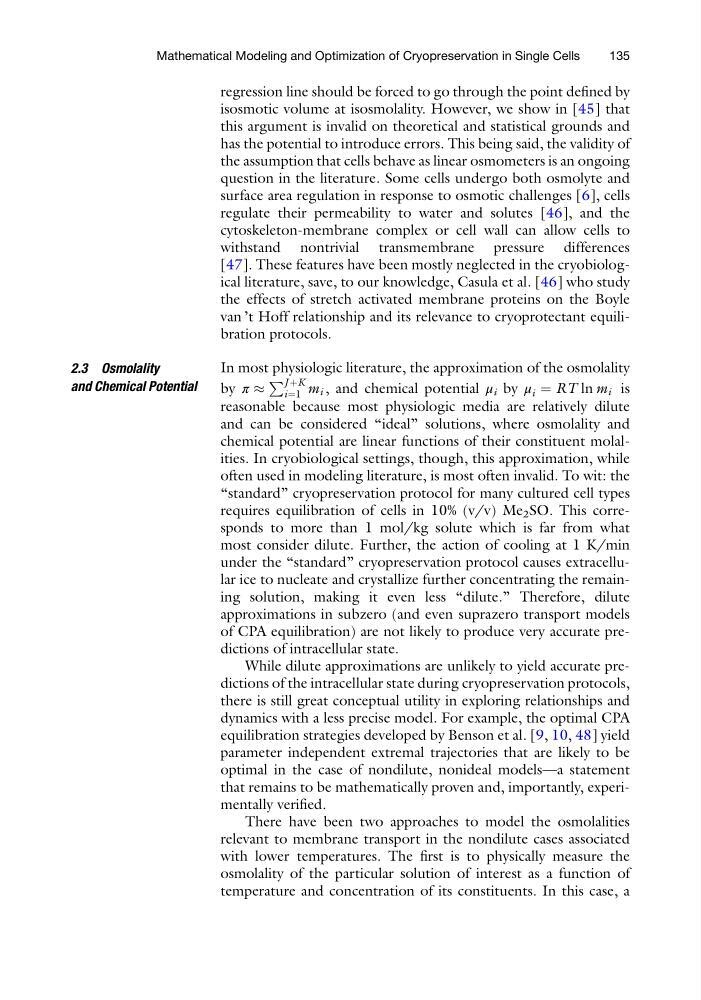
by π %
P J þK
i¼1 m i , and chemical potential μ i by μ i ¼ RT ln m i is
reasonable because most physiologic media are relatively dilute
and can be considered “ideal” solutions, where osmolality and
chemical potential are linear functions of their constituent molalities. In cryobiological settings, though, this approximation, while
often used in modeling literature, is most often invalid. To wit: the
“standard” cryopreservation protocol for many cultured cell types
requires equilibration of cells in 10% (v/v) Me 2 SO. This corresponds to more than 1 mol/kg solute which is far from what
most consider dilute. Further, the action of cooling at 1 K/min
under the “standard” cryopreservation protocol causes extracellular ice to nucleate and crystallize further concentrating the remaining solution, making it even less “dilute.” Therefore, dilute
approximations in subzero (and even suprazero transport models
of CPA equilibration) are not likely to produce very accurate predictions of intracellular state.
While dilute approximations are unlikely to yield accurate predictions of the intracellular state during cryopreservation protocols,
there is still great conceptual utility in exploring relationships and
dynamics with a less precise model. For example, the optimal CPA
equilibration strategies developed by Benson et al. [9, 10, 48] yield
parameter independent extremal trajectories that are likely to be
optimal in the case of nondilute, nonideal models—a statement
that remains to be mathematically proven and, importantly, experimentally verified.
There have been two approaches to model the osmolalities
relevant to membrane transport in the nondilute cases associated
with lower temperatures. The first is to physically measure the
osmolality of the particular solution of interest as a function of
temperature and concentration of its constituents. In this case, a
Mathematical Modeling and Optimization of Cryopreservation in Single Cells
135