

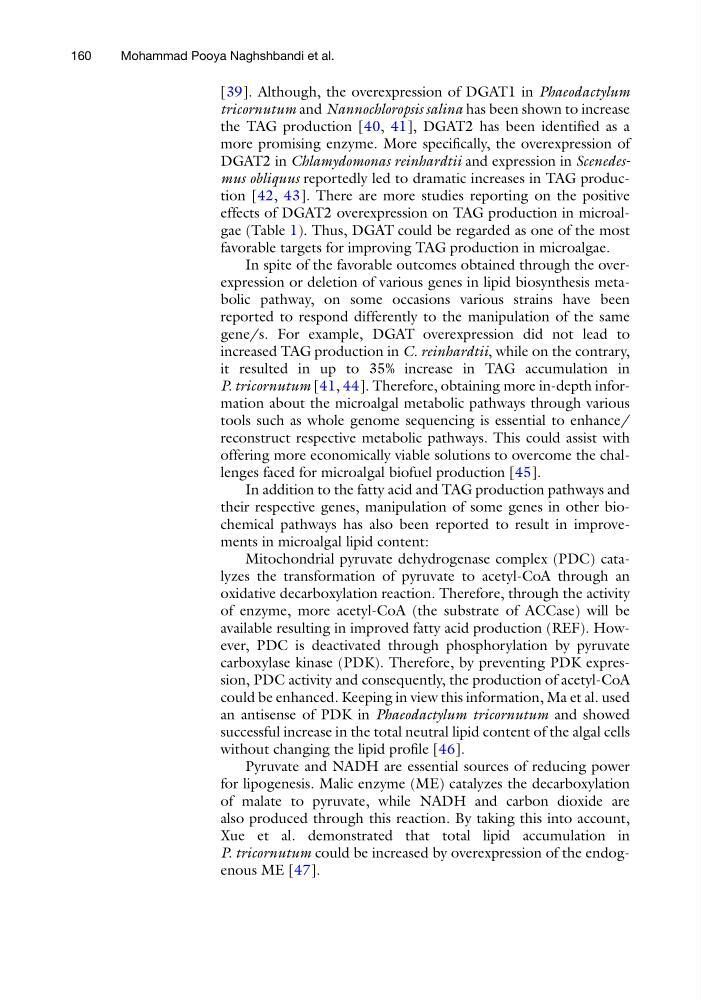
[39]. Although, the overexpression of DGAT1 in Phaeodactylum
tricornutum and Nannochloropsis salina has been shown to increase
the TAG production [40, 41], DGAT2 has been identified as a
more promising enzyme. More specifically, the overexpression of
DGAT2 in Chlamydomonas reinhardtii and expression in Scenedesmus obliquus reportedly led to dramatic increases in TAG production [42, 43]. There are more studies reporting on the positive
effects of DGAT2 overexpression on TAG production in microalgae (Table 1). Thus, DGAT could be regarded as one of the most
favorable targets for improving TAG production in microalgae.
In spite of the favorable outcomes obtained through the overexpression or deletion of various genes in lipid biosynthesis metabolic pathway, on some occasions various strains have been
reported to respond differently to the manipulation of the same
gene/s. For example, DGAT overexpression did not lead to
increased TAG production in C. reinhardtii, while on the contrary,
it resulted in up to 35% increase in TAG accumulation in
P. tricornutum [41, 44]. Therefore, obtaining more in-depth information about the microalgal metabolic pathways through various
tools such as whole genome sequencing is essential to enhance/
reconstruct respective metabolic pathways. This could assist with
offering more economically viable solutions to overcome the challenges faced for microalgal biofuel production [45].
In addition to the fatty acid and TAG production pathways and
their respective genes, manipulation of some genes in other biochemical pathways has also been reported to result in improvements in microalgal lipid content:
Mitochondrial pyruvate dehydrogenase complex (PDC) catalyzes the transformation of pyruvate to acetyl-CoA through an
oxidative decarboxylation reaction. Therefore, through the activity
of enzyme, more acetyl-CoA (the substrate of ACCase) will be
available resulting in improved fatty acid production (REF). However, PDC is deactivated through phosphorylation by pyruvate
carboxylase kinase (PDK). Therefore, by preventing PDK expression, PDC activity and consequently, the production of acetyl-CoA
could be enhanced. Keeping in view this information, Ma et al. used
an antisense of PDK in Phaeodactylum tricornutum and showed
successful increase in the total neutral lipid content of the algal cells
without changing the lipid profile [46].
Pyruvate and NADH are essential sources of reducing power
for lipogenesis. Malic enzyme (ME) catalyzes the decarboxylation
of malate to pyruvate, while NADH and carbon dioxide are
also produced through this reaction. By taking this into account,
Xue et al. demonstrated that total lipid accumulation in
P. tricornutum could be increased by overexpression of the endogenous ME [47].
160
Mohammad Pooya Naghshbandi et al.