

Processes 2018, 6, 134
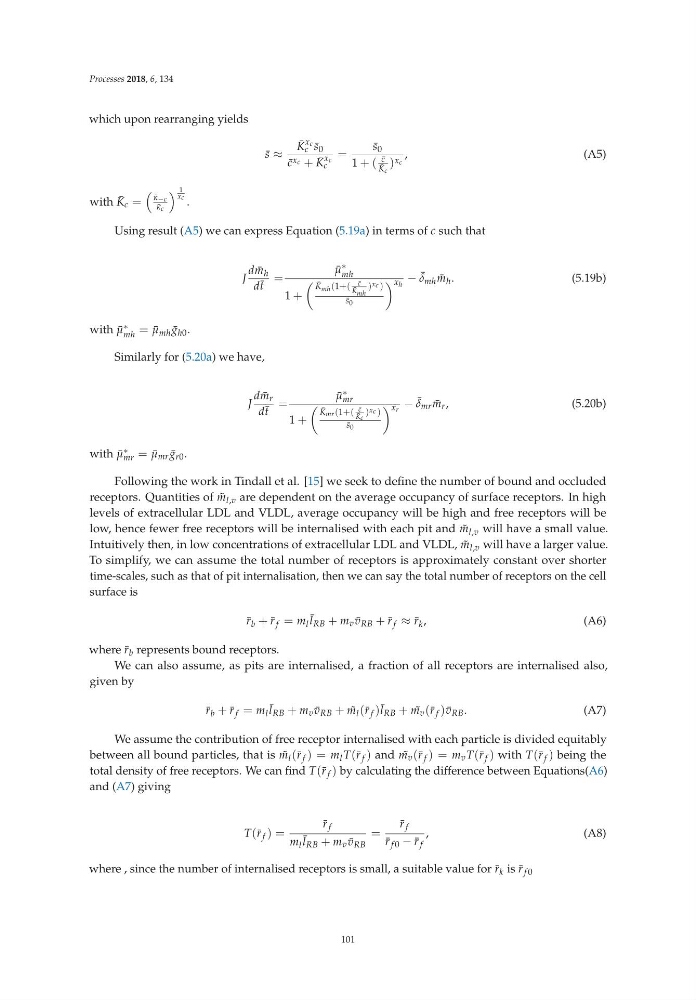
which upon rearranging yields
¯
s ≈
¯
K
xc
c ¯
s 0
¯
c xc + ¯
K
xc
c
=
¯
s 0
1 +(
¯
c
¯
Kc
) xc ,
(A5)
with ¯
K c =
¯
κ−c
¯
κc
1
xc .
Using result (A5) we can express Equation (5.19a) in terms of c such that
J
d ¯
m h
d ¯
t
=
¯
μ ∗
mh
1 +
¯
K mh (1+(
¯
c
¯
K mh
) xc )
¯
s 0
x h − ¯
δ mh ¯
m h .
(5.19b)
with ¯
μ ∗
mh = ¯
μ mh ¯
g h0 .
Similarly for (5.20a) we have,
J
d ¯
m r
d ¯
t
=
¯
μ ∗
mr
1 +
¯
Kmr(1+(
¯
c
¯
Kc
) xc )
¯
s 0
xr − ¯
δ mr ¯
m r ,
(5.20b)
with ¯
μ ∗
mr = ¯
μ mr ¯
g r0 .
Following the work in Tindall et al. [15] we seek to define the number of bound and occluded
receptors. Quantities of ˜
m l,v are dependent on the average occupancy of surface receptors. In high
levels of extracellular LDL and VLDL, average occupancy will be high and free receptors will be
low, hence fewer free receptors will be internalised with each pit and ˜
m l,v will have a small value.
Intuitively then, in low concentrations of extracellular LDL and VLDL, ˜
m l,v will have a larger value.
To simplify, we can assume the total number of receptors is approximately constant over shorter
time-scales, such as that of pit internalisation, then we can say the total number of receptors on the cell
surface is
¯
r b + ¯
r f = m l ¯
l RB + m v ¯
v RB + ¯
r f ≈ ¯
r k ,
(A6)
where ¯
r b represents bound receptors.
We can also assume, as pits are internalised, a fraction of all receptors are internalised also,
given by
¯
r b + ¯
r f = m l ¯
l RB + m v ¯
v RB + ˜
m l (¯ r f ) ¯
l RB + ˜
m v (¯ r f ) ¯
v RB .
(A7)
We assume the contribution of free receptor internalised with each particle is divided equitably
between all bound particles, that is ˜
m l (¯ r f )=m l T(¯ r f ) and ˜
m v (¯ r f )=m v T(¯ r f ) with T(¯ r f ) being the
total density of free receptors. We can find T(¯ r f ) by calculating the difference between Equations(A6)
and (A7) giving
T(¯ r f )=
¯
r f
m l ¯
l RB + m v ¯
v RB
=
¯
r f
¯
r f 0 − ¯
r f
,
(A8)
where , since the number of internalised receptors is small, a suitable value for ¯
r k is ¯
r f 0
101