

Processes 2018, 6, 134
Funding: F.P. acknowledges the support of an Engineering Physical Sciences Research Council (EPSRC) UK CASE
studentship in collaboration with Syngenta (EP/P505682/1 & EP/J500501/1). M.J.T. is grateful for the support of a
Research Council UK Fellowship (EP/C508777/1) during parts of the period in which this work was undertaken.
Conflicts of Interest: The atuhors declare no conflict of interest.
Appendix A. Model Reduction
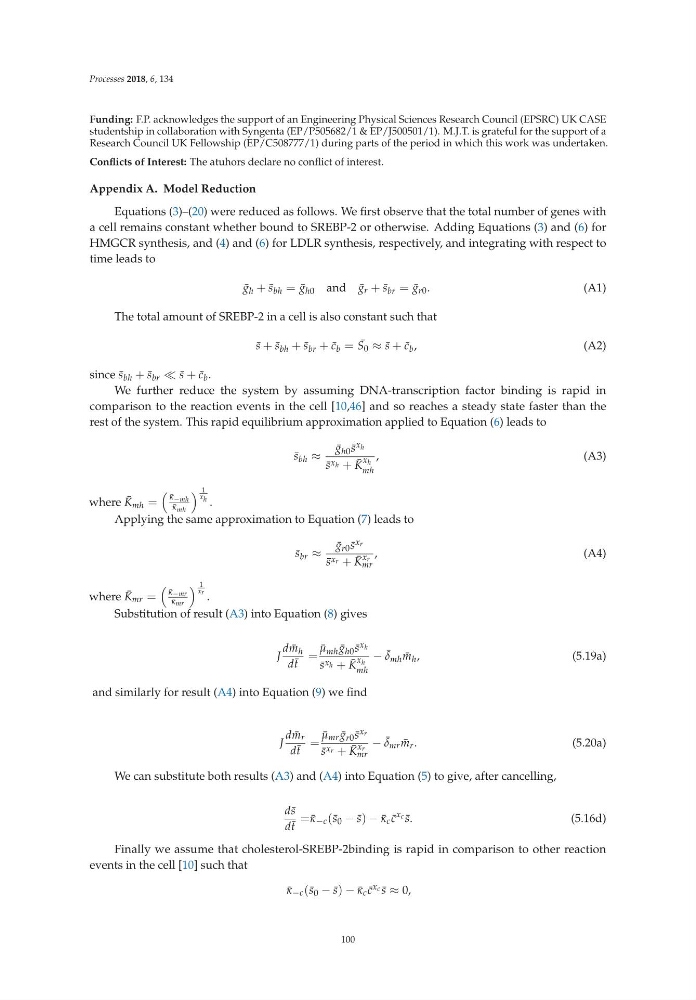
Equations (3)–(20) were reduced as follows. We first observe that the total number of genes with
a cell remains constant whether bound to SREBP-2 or otherwise. Adding Equations (3) and (6) for
HMGCR synthesis, and (4) and (6) for LDLR synthesis, respectively, and integrating with respect to
time leads to
¯
g h + ¯
s bh = ¯
g h0 and ¯
g r + ¯
s br = ¯
g r0 .
(A1)
The total amount of SREBP-2 in a cell is also constant such that
¯
s + ¯
s bh + ¯
s br + ¯
c b = ¯
S 0 ≈ ¯
s + ¯
c b ,
(A2)
since ¯
s bh + ¯
s br ≪ ¯
s + ¯
c b .
We further reduce the system by assuming DNA-transcription factor binding is rapid in
comparison to the reaction events in the cell [10,46] and so reaches a steady state faster than the
rest of the system. This rapid equilibrium approximation applied to Equation (6) leads to
¯
s bh ≈
¯
g h0 ¯
s x h
¯
s x h + ¯
K
x h
mh
,
(A3)
where ¯
K mh =
¯
κ −mh
¯
κ mh
1
x h .
Applying the same approximation to Equation (7) leads to
¯
s br ≈
¯
g r0 ¯
s xr
¯
s xr + ¯
K
xr
mr
,
(A4)
where ¯
K mr =
¯
κ−mr
¯
κmr
1
xr .
Substitution of result (A3) into Equation (8) gives
J
d ¯
m h
d ¯
t
=
¯
μ mh ¯
g h0 ¯
s x h
¯
s x h + ¯
K
x h
mh
− ¯
δ mh ¯
m h ,
(5.19a)
and similarly for result (A4) into Equation (9)wefind
J
d ¯
m r
d ¯
t
=
¯
μ mr ¯
g r0 ¯
s xr
¯
s xr + ¯
K
xr
mr
− ¯
δ mr ¯
m r .
(5.20a)
We can substitute both results (A3) and (A4) into Equation (5) to give, after cancelling,
d ¯
s
d ¯
t
= ¯
κ −c (¯ s 0 − ¯
s) − ¯
κ c ¯
c
xc ¯
s.
(5.16d)
Finally we assume that cholesterol-SREBP-2binding is rapid in comparison to other reaction
events in the cell [10] such that
¯
κ −c (¯ s 0 − ¯
s) − ¯
κ c ¯
c xc ¯
s ≈ 0,
100