

4. ENERGY-RICH COMPOUNDS
125
On the other hand, the phosphate group transferred in Reaction 30
was introduced earlier in the glycolytic scheme via an ATP-dependent
reaction (cf. Eq. 24a). In the latter instance, the "energy-rich" bond has
been conserved, rather than synthesized de novo.
In many systems, and especially in tissues of higher animals, the
major site of ATP synthesis is the citric acid cycle. The complete combustion of one mole of pyruvate to C0 2 and H 2 0 would yield approximately 273 kcal, of energy (27). During the realization of this process
via the citric acid cycle, approximately 14-15 moles of ATP are synthesized. ATP synthesis can occur only concomitantly with oxidative
steps in the cycle (i.e., pyruvate —> acetate, isocitrate-» oxalosuccinate,
a-ketoglutarate —» succinate, succinate —> fumarate, and malate -» oxaloacetate). The term "oxidative phosphorylation" has been given to the
process whereby Pi and ADP interact to form ATP during these oxidative steps (see pertinent reviews (79-83a). It should be noted that
this process results in the de novo synthesis of ATP from "energy-poor"
components.
The mechanism of oxidative phosphorylation is still obscure, due, at
least in part, to the fact that the enzymes responsible for this process
are found in most tissues to be associated with subcellular particles.
These may be comminuted by treatment with digitonin (84, 85),
ethanol (86-87a), or sonic oscillation (88-89a), to produce still smaller
particles which retain the ability to carry out oxidative phosphorylation. It has been suggested that phosphorylation occurs at several points
in the electron transport sequence intervening between the substrate
and molecular oxygen. This view has been given strong support by the
spectroscopic studies of Chance and his colleagues (83). Evidence has
been obtained that there are 3 sites of phosphorylation in the sequence
between DPNH and 0 2 : (1) between DPNH and a flavoprotein; (2)
between cytochromes b and c; and (3) between cytochromes c and a.
Furthermore, it has been noted that carefully prepared mitochondria
("tightly coupled" mitochondria) do not oxidize substrates until ADP
is added to initiate oxidative phosphorylation. A hypothetical scheme
showing oxidative phosphorylation at one stage in the electron transport sequence is given in Fig. 5. "A" and "AH 2 " represent a typical
substrate in the oxidized and reduced form. "DPNH ^ P" symbolizes
an "energy-rich" adduct between Pi and DPNH, which is not oxidized
by the flavoprotein system until the ^P is removed by transphosphorylation with ADP. The simplified net reaction for oxidative phosphorylation is depicted in Eq. 32. The resemblance of this reaction
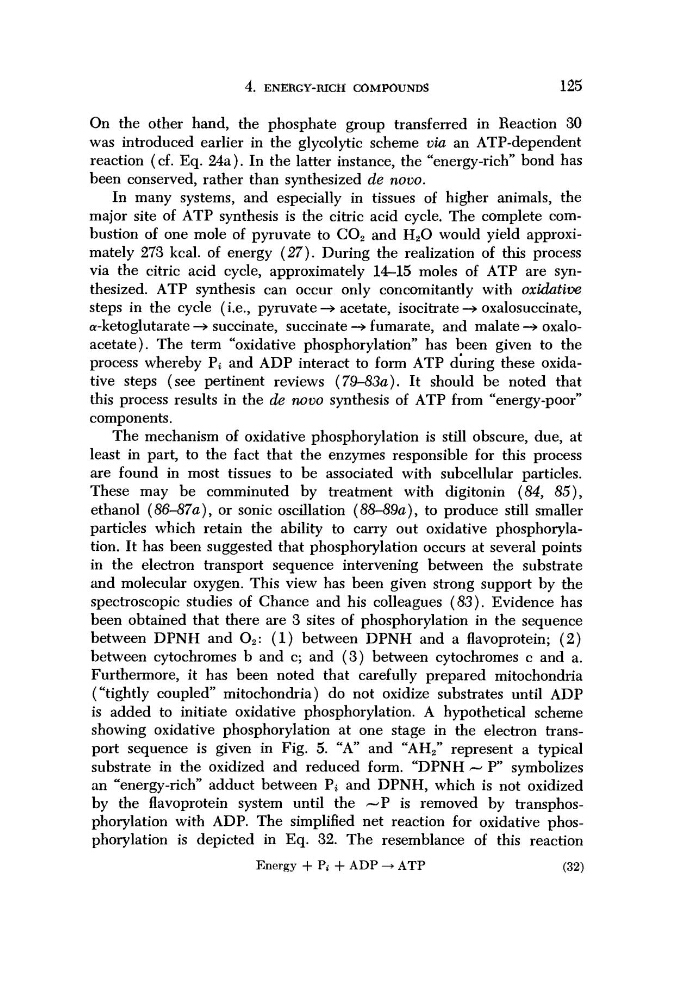
Energy + P t + ADP -* ATP
(32)