

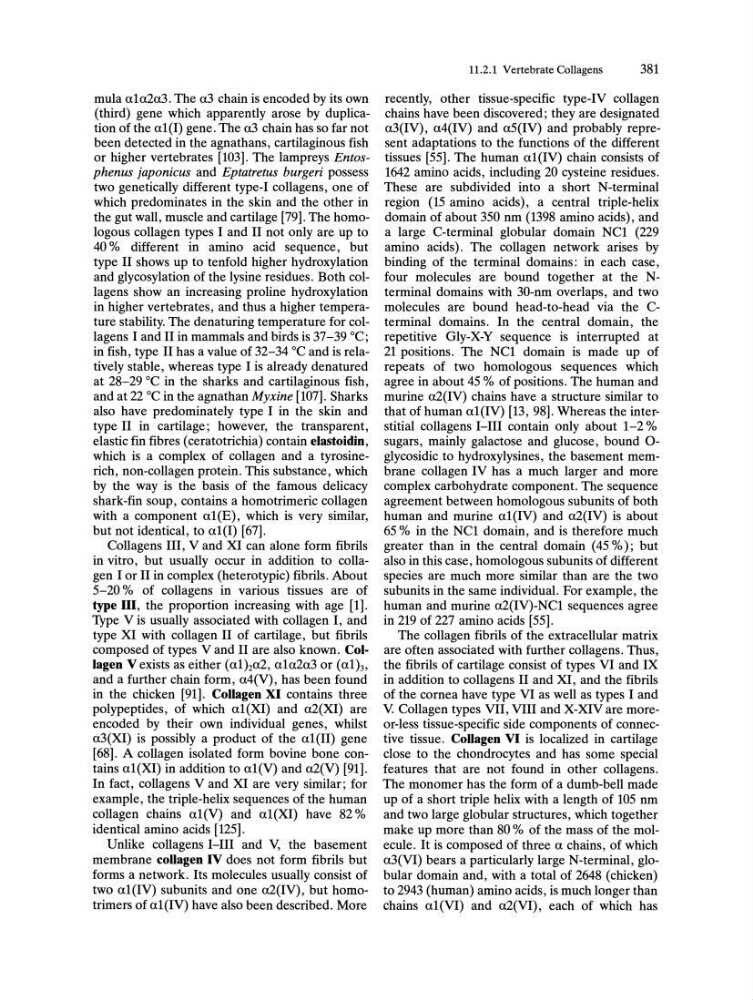
mula ala2a3. The a3 chain is encoded by its own
(third) gene which apparently arose by duplication of the al(I) gene. The a3 chain has so far not
been detected in the agnathans, cartilaginous fish
or higher vertebrates [103]. The lampreys Entosphenus japonicus and Eptatretus burgeri possess
two genetically different type-I collagens, one of
which predominates in the skin and the other in
the gut wall, muscle and cartilage [79]. The homologous collagen types I and II not only are up to
40 % different in amino acid sequence, but
type II shows up to tenfold higher hydroxylation
and glycosylation of the lysine residues. Both collagens show an increasing proline hydroxylation
in higher vertebrates, and thus a higher temperature stability. The denaturing temperature for collagens I and II in mammals and birds is 37-39 °C;
in fish, type II has a value of 32-34 °C and is relatively stable, whereas type I is already denatured
at 28-29 °C in the sharks and cartilaginous fish,
and at 22°C in the agnathan Myxine [107]. Sharks
also have predominately type I in the skin and
type II in cartilage; however, the transparent,
elastic fin fibres (ceratotrichia) contain elastoidin,
which is a complex of collagen and a tyrosinerich, non-collagen protein. This substance, which
by the way is the basis of the famous delicacy
shark-fin soup, contains a homotrimeric collagen
with a component al(E), which is very similar,
but not identical, to al(I) [67].
Collagens III, V and XI can alone form fibrils
in vitro, but usually occur in addition to collagen lor II in complex (heterotypic) fibrils. About
5-20 % of collagens in various tissues are of
type III, the proportion increasing with age [1].
Type V is usually associated with collagen I, and
type XI with collagen II of cartilage, but fibrils
composed of types V and II are also known. Collagen V exists as either (al)2a2, ala2a3 or (alh,
and a further chain form, a4(V), has been found
in the chicken [91]. Collagen XI contains three
polypeptides, of which al(XI) and a2(XI) are
encoded by their own individual genes, whilst
a3(XI) is possibly a product of the al(II) gene
[68]. A collagen isolated form bovine bone contains al(XI) in addition to al(V) and a2(V) [91].
In fact, collagens V and XI are very similar; for
example, the triple-helix sequences of the human
collagen chains al(V) and al(XI) have 82 %
identical amino acids [125].
Unlike collagens I-III and V, the basement
membrane collagen IV does not form fibrils but
forms a network. Its molecules usually consist of
two al(IV) subunits and one a2(IV), but homotrimers of al(IV) have also been described. More
11.2.1 Vertebrate Collagens
381
recently, other tissue-specific type-IV collagen
chains have been discovered; they are designated
a3(IV) , a4(IV) and a5(IV) and probably represent adaptations to the functions of the different
tissues [55]. The human al(IV) chain consists of
1642 amino acids, including 20 cysteine residues.
These are subdivided into a short N-terminal
region (15 amino acids), a central triple-helix
domain of about 350 nm (1398 amino acids), and
a large C-terminal globular domain NCl (229
amino acids). The collagen network arises by
binding of the terminal domains: in each case,
four molecules are bound together at the Nterminal domains with 30-nm overlaps, and two
molecules are bound head-to-head via the Cterminal domains. In the central domain, the
repetitive Gly-X-Y sequence is interrupted at
21 positions. The NCl domain is made up of
repeats of two homologous sequences which
agree in about 45 % of positions. The human and
murine a2(IV) chains have a structure similar to
that of human al(IV) [13, 98]. Whereas the interstitial collagens I-III contain only about 1-2 %
sugars, mainly galactose and glucose, bound 0glycosidic to hydroxylysines, the basement membrane collagen IV has a much larger and more
complex carbohydrate component. The sequence
agreement between homologous subunits of both
human and murine al(IV) and a2(IV) is about
65 % in the NCl domain, and is therefore much
greater than in the central domain (45 % ); but
also in this case, homologous subunits of different
species are much more similar than are the two
subunits in the same individual. For example, the
human and murine a2(IV)-NCl sequences agree
in 219 of 227 amino acids [55].
The collagen fibrils of the extracellular matrix
are often associated with further collagens. Thus,
the fibrils of cartilage consist of types VI and IX
in addition to collagens II and XI, and the fibrils
of the cornea have type VI as well as types I and
V. Collagen types VII, VIII and X-XIV are moreor-less tissue-specific side components of connective tissue. Collagen VI is localized in cartilage
close to the chondrocytes and has some special
features that are not found in other collagens.
The monomer has the form of a dumb-bell made
up of a short triple helix with a length of 105 nm
and two large globular structures, which together
make up more than 80 % of the mass of the molecule. It is composed of three a chains, of which
a3(VI) bears a particularly large N-terminal, globular domain and, with a total of 2648 (chicken)
to 2943 (human) amino acids, is much longer than
chains al(VI) and a2(VI), each of which has