

Photosynthesis as a Tool for Indicating Temperature Stress Events
271
cellular ice formation and freeze-induced dehydration of the protoplasm
("freezing tolerance"). Plants that are only protected by avoidance mechanisms are subject to immediate injury as soon as ice forms in their tissues.
Nevertheless, in freezing-sensitive plants of this kind ice nucleation can
be prevented for a considerable time by persistent supercooling (Larcher
1982). Supercooling as a survival mechanism is not only important for bud
primordia, xylem parenchyma and seeds, but also for leaves of certain plants
of regions subject to episodic frosts down to about -10°C (e.g., some
palms, bamboos, Olea, Polylepsis; Sakai and Larcher 1987). By means
of differential thermal analysis combined with chlorophyll fluorescence
measurements, it was shown on Trachycarpus !ortunei, a palm species growing in warm temperate regions, that the leaves can be persistently supercooled down to -14°C and that their frost resistance is based solely upon
freezing avoidance (Larcher et al. 1991 b). Leaves that survive frost temperatures by maintaining supercooling resume full photosynthetic activity upon
rewarming and exhibit no inhibitory after-effects.
2. Detection of different states of acclimation. A moderate improvement
in frost resistance can be achieved by freezing point depression and enhanced
supercooling. This is normally effected by cold acclimation during the course
of a few cooler days. However, lowering of the tissue freezing point and
stabilization of the cell membranes can also be observed in connection
with a general rise in resistance under the influence of stress factors (e.g.,
drought). Vigna unguiculata plants grown under salt stress (by addition of
100 to 200 mM NaCl to the substrate) were less susceptible to freezing than
control plants; in the salinized plants photosynthesis was less depressed
at the temperatures below + 5 °C and the tissue-freezing temperature was
lowered by 2 to 3 K as compared to nonsalinized plants (Larcher et al.
1990). The rise in temperature resistance under chronic saline stress points
to adjustments at the level of proteins and biomembranes, resulting in a
general stabilization of protoplasmic structures.
In regions with cold winters there is a regular progression to different
levels of hardiness. In woody plants, there is not only a rise in the degree of
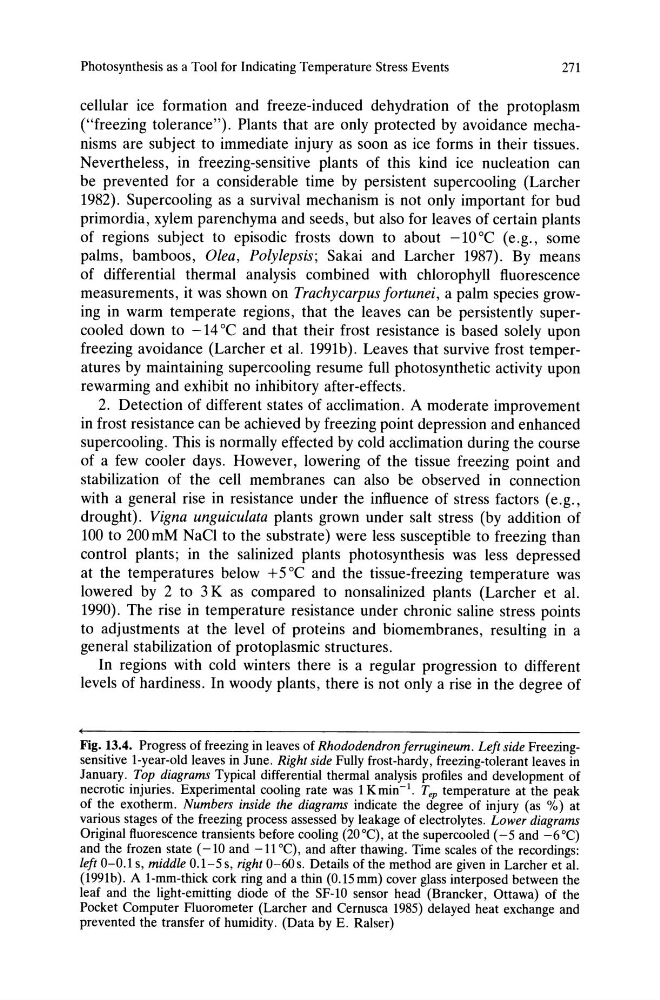
Fig. 13.4. Progress of freezing in leaves of Rhododendron ferrugineum. Left side Freezingsensitive l-year-old leaves in June. Right side Fully frost-hardy, freezing-tolerant leaves in
January. Top diagrams Typical differential thermal analysis profiles and development of
necrotic injuries. Experimental cooling rate was 1 Kmin-I. Tep temperature at the peak
of the exotherm. Numbers inside the diagrams indicate the degree of injury (as %) at
various stages of the freezing process assessed by leakage of electrolytes. Lower diagrams
Original fluorescence transients before cooling (20°C), at the supercooled (-5 and -6°C)
and the frozen state (-10 and -11 0C), and after thawing. Time scales of the recordings:
left 0-0.1 s, middle 0.1-5 s, right 0-60 s. Details of the method are given in Larcher et al.
(1991b). A I-mm-thick cork ring and a thin (0.15mm) cover glass interposed between the
leaf and the light-emitting diode of the SF-1O sensor head (Brancker, Ottawa) of the
Pocket Computer Fluorometer (Larcher and Cernusca 1985) delayed heat exchange and
prevented the transfer of humidity. (Data by E. Raiser)