

Internal Coordination of Plant Responses to Drought and Evaporational Demand
193
7.5
... 7.0
-a.
Co
~ 6.5
E
~
6.0
Helianthus annuus
•
5.5 -f-----r-----r---...,.-----'
0.05
0.10
0.15
0.20
Soil water content (g g.l)
1000
'?E
! 100
:s III
.12
i
10
Ba reulh 1988
•
... ~. ... .
• i'~
• •
•
I. '
•••
•
1~--~-~~-~--~
o
5
10
15
20
Xylem sap nitrate (mol m-3 )
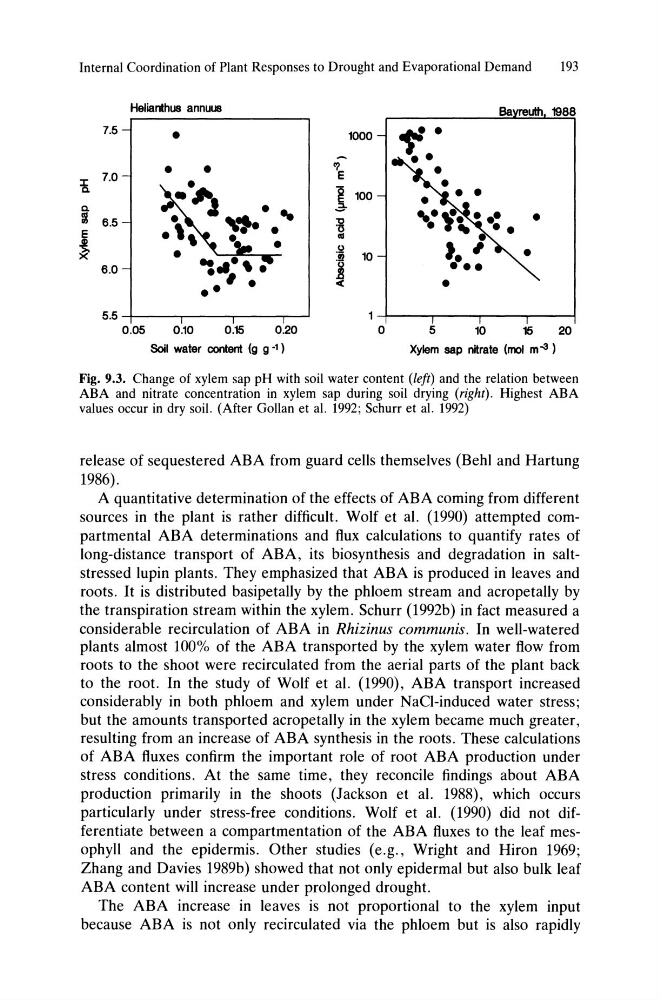
Fig. 9.3. Change of xylem sap pH with soil water content (left) and the relation between
ABA and nitrate concentration in xylem sap during soil drying (right). Highest ABA
values occur in dry soil. (After Gollan et al. 1992; Schurr et al. 1992)
release of sequestered ABA from guard cells themselves (Behl and Hartung
1986).
A quantitative determination of the effects of ABA coming from different
sources in the plant is rather difficult. Wolf et al. (1990) attempted compartmental ABA determinations and flux calculations to quantify rates of
long-distance transport of ABA, its biosynthesis and degradation in saltstressed lupin plants. They emphasized that ABA is produced in leaves and
roots. It is distributed basipetally by the phloem stream and acropetally by
the transpiration stream within the xylem. Schurr (1992b) in fact measured a
considerable recirculation of ABA in Rhizinus communis. In well-watered
plants almost 100% of the ABA transported by the xylem water flow from
roots to the shoot were recirculated from the aerial parts of the plant back
to the root. In the study of Wolf et al. (1990), ABA transport increased
considerably in both phloem and xylem under NaCl-induced water stress;
but the amounts transported acropetally in the xylem became much greater,
resulting from an increase of ABA synthesis in the roots. These calculations
of ABA fluxes confirm the important role of root ABA production under
stress conditions. At the same time, they reconcile findings about ABA
production primarily in the shoots (Jackson et al. 1988), which occurs
particularly under stress-free conditions. Wolf et al. (1990) did not differentiate between a compartmentation of the ABA fluxes to the leaf mesophyll and the epidermis. Other studies (e.g., Wright and Hiron 1969;
Zhang and Davies 1989b) showed that not only epidermal but also bulk leaf
ABA content will increase under prolonged drought.
The ABA increase in leaves is not proportional to the xylem input
because ABA is not only recirculated via the phloem but is also rapidly