

224
Davidson et al. 1991). This method promotes uniform distribution of the isotope throughout the soil
volume; however, if ambient nutrient concentrations are heterogeneous, then the isotopic enrichment will also be heterogeneous because micro sites
with low ambient concentrations will become more
highly enriched than micro sites with high concentrations. In tracer and isotope dilution studies where
soils have had low NHt or NO; concentrations,
researchers have sometimes combined NHt and
NO; pools for isotope analysis. This approach also
violates the assumption of uniform distribution of
isotope because the NHt and NO; pools are likely
to have different enrichments (Schimel1996). For
example, if the NHt pool is more highly enriched
in 15N, then consumption of NHt will result in
greater 15N uptake than the same rate of NO; consumption. Modeling studies have shown that errors
in rate estimates caused by non-uniform isotope
distributions depend on how isotope is distributed
relative to transformation rates (Davidson et al.
1991; Milchunas and Lauenroth 1992). If the nonuniformity in isotope distribution is random with
respect to rates, then little error results; however, if
the most active pools are more highly enriched in
isotope, then rates will be overestimated. The importance of non-uniform isotope enrichments as a
source of error in soil transformation rate measurements needs further evaluation.
Stimulation of rates by addition of isotope may
be another important source of error in tracer studies. Many nutrient transformation rates are substrate limited, and thus, increased substrate availability will increase transformation rates. For this
reason, the amount of isotope added should be just
high enough to ensure that detectable quantities
will appear in sink pools at the end of the incubation. To decide how much isotope to add, one must
have initial estimates (guesses) of source and sink
pool sizes and gross transformation rates. Preliminary experiments may be necessary to obtain this
information.
Flow of nutrients either into the labeled source
pool or out of the sink pool can cause large errors
in rate estimates based on tracer calculations. If nutrients flow into the source pool, the isotopic enrichment (IA in Equation 14.6) will decline during
the incubation, and thus, a greater total number of
nutrient atoms will be transferred to the sink pool
for each atom of isotope that is transferred. When
John M. Stark
dilution of the isotopic enrichment of the source
pool occurs, isotope dilution calculations must be
used to accurately estimate rates (see next section,
Equations 14.10 and 14.11).
If nutrients flow out of sink pools during the incubation period, then the amount of isotope that is
recovered in the sink pool will underestimate the
amount of isotope that really flowed into that pool.
For example, the tracer equation (Equation 14.6)
will underestimate the flow of nutrient from pool
A into pool C because some of the isotope moved
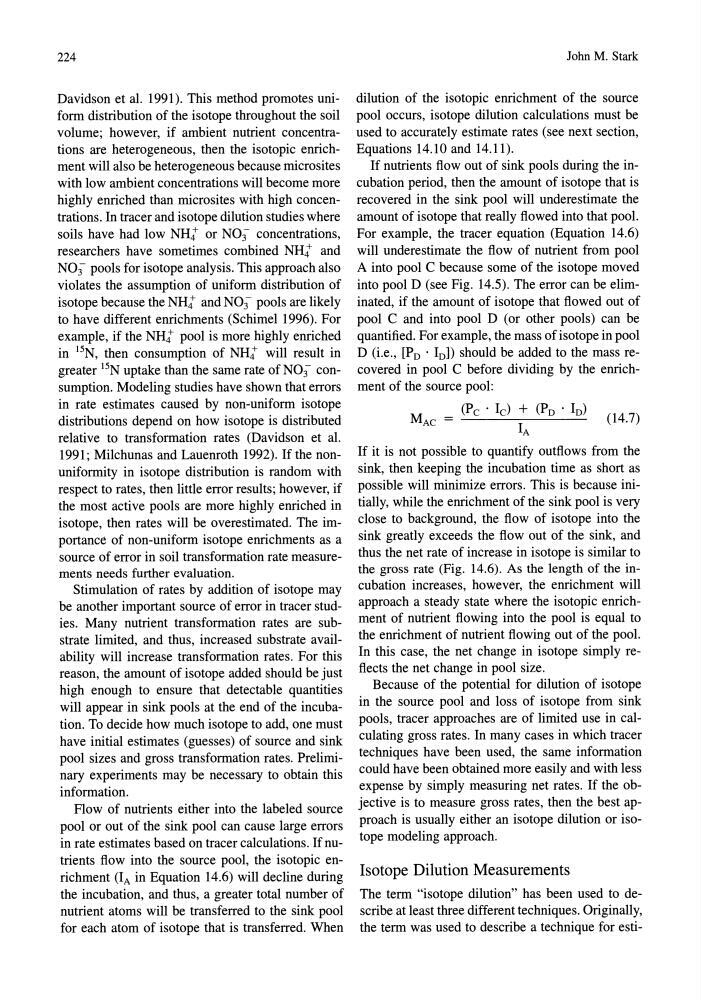
into pool D (see Fig. 14.5). The error can be eliminated, if the amount of isotope that flowed out of
pool C and into pool D (or other pools) can be
quantified. For example, the mass of isotope in pool
D (i.e., [PD . IDD should be added to the mass recovered in pool C before dividing by the enrichment of the source pool:
MAC = (Pc· Ie) + (PD • ID) (14.7)
IA
If it is not possible to quantify outflows from the
sink, then keeping the incubation time as short as
possible will minimize errors. This is because initially, while the enrichment of the sink pool is very
close to background, the flow of isotope into the
sink greatly exceeds the flow out of the sink, and
thus the net rate of increase in isotope is similar to
the gross rate (Fig. 14.6). As the length of the incubation increases, however, the enrichment will
approach a steady state where the isotopic enrichment of nutrient flowing into the pool is equal to
the enrichment of nutrient flowing out of the pool.
In this case, the net change in isotope simply reflects the net change in pool size.
Because of the potential for dilution of isotope
in the source pool and loss of isotope from sink
pools, tracer approaches are of limited use in calculating gross rates. In many cases in which tracer
techniques have been used, the same information
could have been obtained more easily and with less
expense by simply measuring net rates. If the objective is to measure gross rates, then the best approach is usually either an isotope dilution or isotope modeling approach.
Isotope Dilution Measurements
The term "isotope dilution" has been used to describe at least three different techniques. Originally,
the term was used to describe a technique for esti-