

8. Stable Isotope Tracers and Mathematical Models in Soil Organic Matter Studies
125
nate include very sandy soils, and particularly
Spodosols.
The third term on the right hand side of Equation
8.14 represents loss of SOC from the profile due to
heterotrophic respiration or leaching of DOC. It is
analogous to the decomposition term presented in
Equation 8.4. Here, we assume that k is constant
with depth. The notion that a single decomposition
rate, k, is inadequate to fully represent SOC dynamics has led to the development of models that consider multiple pools of SaM: either simply as we
present in the next section (Trumbore 1993) or by
introducing multiple simultaneous versions of
Equations 8.14 and 8.15, each for different SaM
pools (O'Brien and Stout 1978; Elzein and Balesdent, 1995).
The final term on the right side of Equation 8.14
(fd) represents inputs of SOC from plant roots. The
flux of aboveground litter at the soil surface must
also be considered in the upper boundary condition.
O'Brien and Stout (1978) successfully account for
the distribution of l3C and 14C in a forest soil, converted to pasture, while considering only inputs of
litter at the soil surface. Fitting a multi-pool version
of Equation 8.14 to SOC concentration and 14C
content, Elzein and Balesdent (1995) obtain relatively similar results with and without including
root inputs. Thus, it may be appropriate to ignore
the last term in Equation 8.14 in systems such as
forests, or shallowly rooted pastures, where most
root activity is near the mineral soil surface or in
the litter layers. Alternatively, a model that considers only surface inputs may suffer by not recognizing the large inputs of SaM directly from living
and recently deceased plant roots. In many environments, such as grassland and steppes, where
much of the photosynthetic productivity of the
plants is directed below ground (e.g., Lauenroth
and Whitman 1977), the distribution of SaM with
depth is well correlated with root densities (Gile et
al. 1979; Amundson et al. 1989). For these environments, root inputs clearly must be considered:
it is common for grasslands to have belowground/
aboveground inputs ratios of 2: 1 or more (Bray
1963; Volobuev 1964; Kononova 1966; Lauenroth
and Whitman, 1977), while in forests, the ratio can
commonly be <1 (Bray 1963; Volobuev 1964;
Vogt 1991).
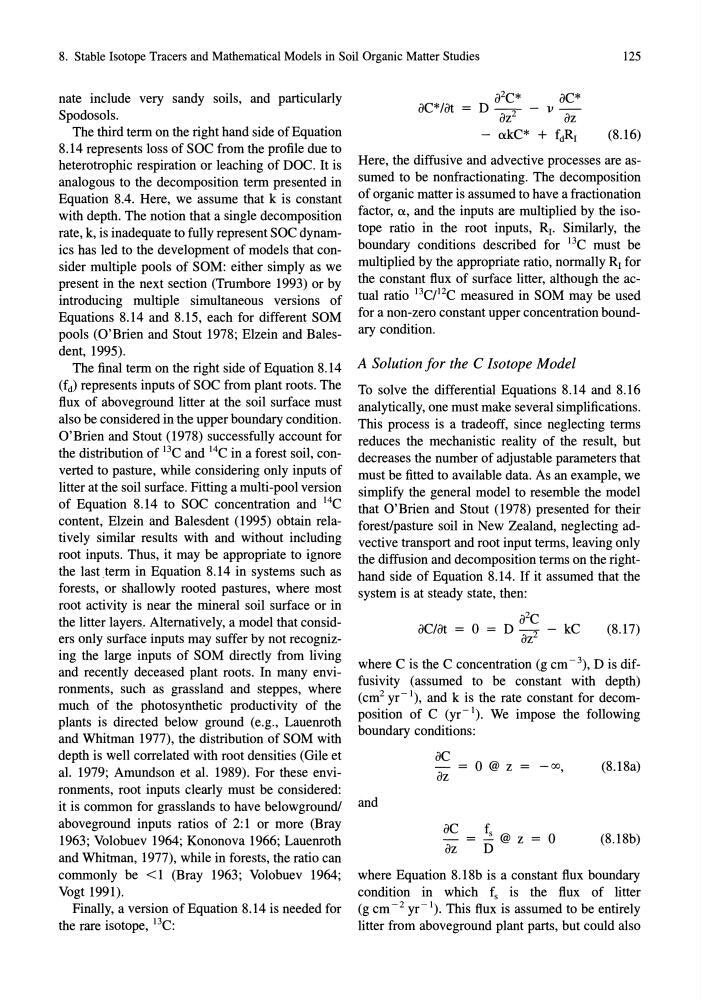
Finally, a version of Equation 8.14 is needed for
the rare isotope, l3C:
aC*lat
a 2 c*
ac*
D - -
v -
az 2
az
- akC* + fdRr
(8.16)
Here, the diffusive and advective processes are assumed to be nonfractionating. The decomposition
of organic matter is assumed to have a fractionation
factor, a, and the inputs are multiplied by the isotope ratio in the root inputs, R r . Similarly, the
boundary conditions described for l3C must be
multiplied by the appropriate ratio, normally Rr for
the constant flux of surface litter, although the actual ratio l3C/ 12 C measured in SaM may be used
for a non-zero constant upper concentration boundary condition.
A Solution for the C Isotope Model
To solve the differential Equations 8.14 and 8.16
analytically, one must make several simplifications.
This process is a tradeoff, since neglecting terms
reduces the mechanistic reality of the result, but
decreases the number of adjustable parameters that
must be fitted to available data. As an example, we
simplify the general model to resemble the model
that O'Brien and Stout (1978) presented for their
forest/pasture soil in New Zealand, neglecting advective transport and root input terms, leaving only
the diffusion and decomposition terms on the righthand side of Equation 8.14. If it assumed that the
system is at steady state, then:
a 2 c
aClat = 0 = D - 2 - kC
az
(8.17)
where C is the C concentration (g cm - 3), D is diffusivity (assumed to be constant with depth)
(cm 2 yr - I), and k is the rate constant for decomposition of C (yr- I ). We impose the following
boundary conditions:
and
ac
-
= 0 @ z
az
-00 ,
ac
az
fs
-@z=O
D
(8.18a)
(8.18b)
where Equation 8.18b is a constant flux boundary
condition in which fs is the flux of litter
(g cm -2 yr- I ). This flux is assumed to be entirely
litter from aboveground plant parts, but could also