

176
K. Fennel· T. Neumann
March. During the same time period in 1995, the winds were stronger, with
speed exceeding 10 mIs, and therefore a deeper mixed layer existed until 9 of
April which reduced the growth of the phytoplankton. Later, the winds decreased and an exponential growth of the phytoplankton started. During April,
May and June of 1994, the frequency of strong winds was higher than in the same
period in 1995. Nutrients are exhausted in the euphotic zone during this time
and strong winds are an effective mechanism for transporting nutrients from
deeper regions of the water column into the euphotic zone, e.g. 21.5.1994 at station 113 (Fig. 2).
3.2
The Influence of the Grid Resolution on Tracer Concentration
The values of chemical-biological variables in the model are averaged over grid
boxes of 1 nautical mile x 1 nautical mile x 2 m size. Processes on smaller scales
than grid size are not resolved explicitly, e.g. the chemical-biological nutrient
uptake or the physical turbulence. These sub-grid processes are described via
parametrizations by processes having spatial scales comparable to the grid resolution or larger.
There are also parts of the circulation pattern with spatial dimensions in the
range of grid size, e.g. mesoscale circulation. The choice of grid width determines which parts are resolved explicitly and which are sub grid processes and
treated by parametrizations. Because of the non-linear coupling of chemical-biological dynamics and circulation the question arises: how are the chemical-biological interactions influenced by changes of the model resolution?
Model experiments with the same parameters and forcing, but different horizontal resolution, were performed. We compare two simulations: a fine scale
model run with the horizontal grid width of 1 nautical mile and a coarse scale
model run with twice the horizontal grid width and twice the horizontal mixing
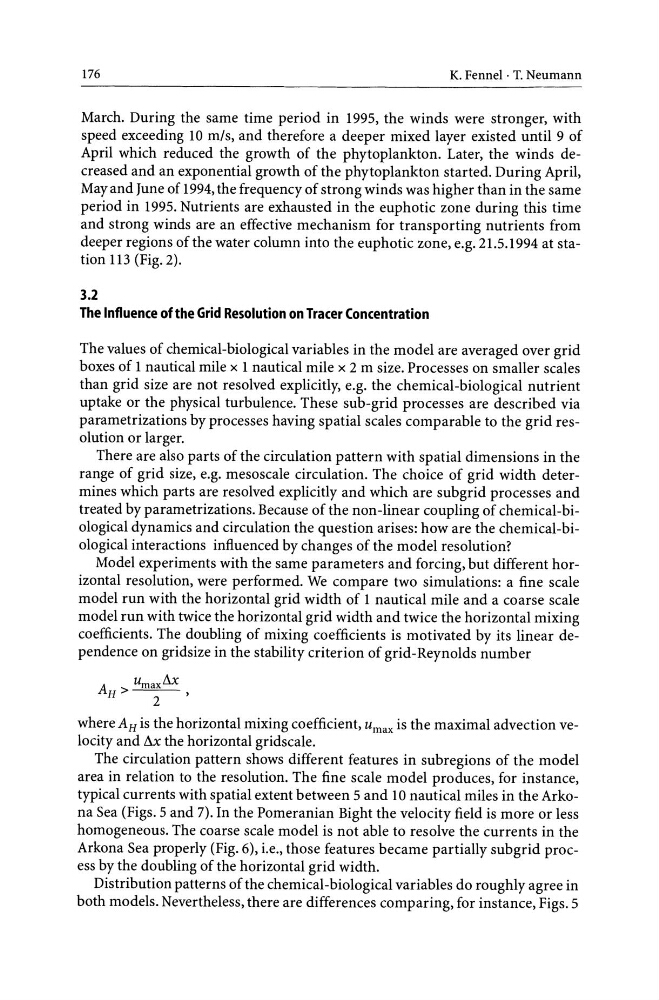
coefficients. The doubling of mixing coefficients is motivated by its linear dependence on gridsize in the stability criterion of grid-Reynolds number
A
umax.1x
H>
,
2
where AH is the horizontal mixing coefficient, u max is the maximal advection velocity and .1x the horizontal gridscale.
The circulation pattern shows different features in subregions of the model
area in relation to the resolution. The fine scale model produces, for instance,
typical currents with spatial extent between 5 and 10 nautical miles in the Arkona Sea (Figs. 5 and 7). In the Pomeranian Bight the velocity field is more or less
homogeneous. The coarse scale model is not able to resolve the currents in the
Arkona Sea properly (Fig. 6), i.e., those features became partially subgrid process by the doubling of the horizontal grid width.
Distribution patterns of the chemical-biological variables do roughly agree in
both models. Nevertheless, there are differences comparing, for instance, Figs. 5