

Biogenic Barium as a Proxy for Paleoproductivity
351
tor in regulating the flux of biogenic barium to the
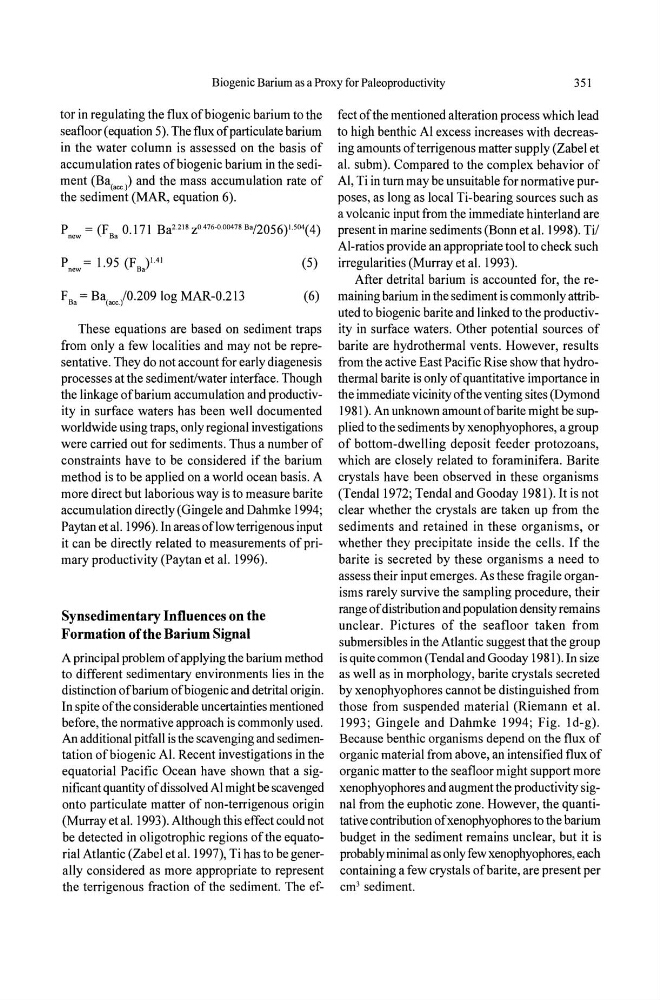
seafloor (equation 5). The flux of particulate barium
in the water column is assessed on the basis of
accumulation rates of biogenic barium in the sediment (Ba(acc») and the mass accumulation rate of
the sediment (MAR, equation 6).
Pn,w = (F Ba 0.171 Ba2.218 Z0,476-0.00478 BaI2056)LS04( 4)
F Ba = Ba(acc/O.20910g MAR-O.213
(6)
These equations are based on sediment traps
from only a few localities and may not be representative. They do not account for early diagenesis
processes at the sediment/water interface. Though
the linkage of barium accumulation and productivity in surface waters has been well documented
worldwide using traps, only regional investigations
were carried out for sediments. Thus a number of
constraints have to be considered if the barium
method is to be applied on a world ocean basis. A
more direct but laborious way is to measure barite
accumulation directly (Gingele and Dahmke 1994;
Paytan et al. 1996). In areas oflow terrigenous input
it can be directly related to measurements of primary productivity (Paytan et al. 1996).
Synsedimentary Influences on the
Formation ofthe Barium Signal
A principal problem of applying the barium method
to different sedimentary environments lies in the
distinction of barium of biogenic and detrital origin.
In spite of the considerable uncertainties mentioned
before, the normative approach is commonly used.
An additional pitfall is the scavenging and sedimentation of biogenic AI. Recent investigations in the
equatorial Pacific Ocean have shown that a significant quantity of dissolved Al might be scavenged
onto particulate matter of non-terrigenous origin
(Murray et al. 1993). Although this effect could not
be detected in oligotrophic regions of the equatorial Atlantic (Zabel et al. 1997), Ti has to be generally considered as more appropriate to represent
the terrigenous fraction of the sediment. The effect of the mentioned alteration process which lead
to high benthic Al excess increases with decreasing amounts of terrigenous matter supply (Zabel et
al. subm). Compared to the complex behavior of
AI, Ti in tum may be unsuitable for normative purposes, as long as local Ti-bearing sources such as
a volcanic input from the immediate hinterland are
present in marine sediments (Bonn et al. 1998). Til
AI-ratios provide an appropriate tool to check such
irregularities (Murray et al. 1993).
After detrital barium is accounted for, the remaining barium in the sediment is commonly attributed to biogenic barite and linked to the productivity in surface waters. Other potential sources of
barite are hydrothermal vents. However, results
from the active East Pacific Rise show that hydrothermal barite is only of quantitative importance in
the immediate vicinity of the venting sites (Dymond
1981 ). An unknown amount of barite might be supplied to the sediments by xenophyophores, a group
of bottom-dwelling deposit feeder protozoans,
which are closely related to foraminifera. Barite
crystals have been observed in these organisms
(TendaI1972; Tendal and Gooday 1981). It is not
clear whether the crystals are taken up from the
sediments and retained in these organisms, or
whether they precipitate inside the cells. If the
barite is secreted by these organisms a need to
assess their input emerges. As these fragile organisms rarely survive the sampling procedure, their
range of distribution and population density remains
unclear. Pictures of the seafloor taken from
submersibles in the Atlantic suggest that the group
is quite common (Tendal and Gooday 1981). In size
as well as in morphology, barite crystals secreted
by xenophyophores cannot be distinguished from
those from suspended material (Riemann et al.
1993; Gingele and Dahmke 1994; Fig. Id-g).
Because benthic organisms depend on the flux of
organic material from above, an intensified flux of
organic matter to the seafloor might support more
xenophyophores and augment the productivity signal from the euphotic zone. However, the quantitative contribution of xenophyophores to the barium
budget in the sediment remains unclear, but it is
probably minimal as only few xenophyophores, each
containing a few crystals of barite, are present per
cm 3 sediment.