

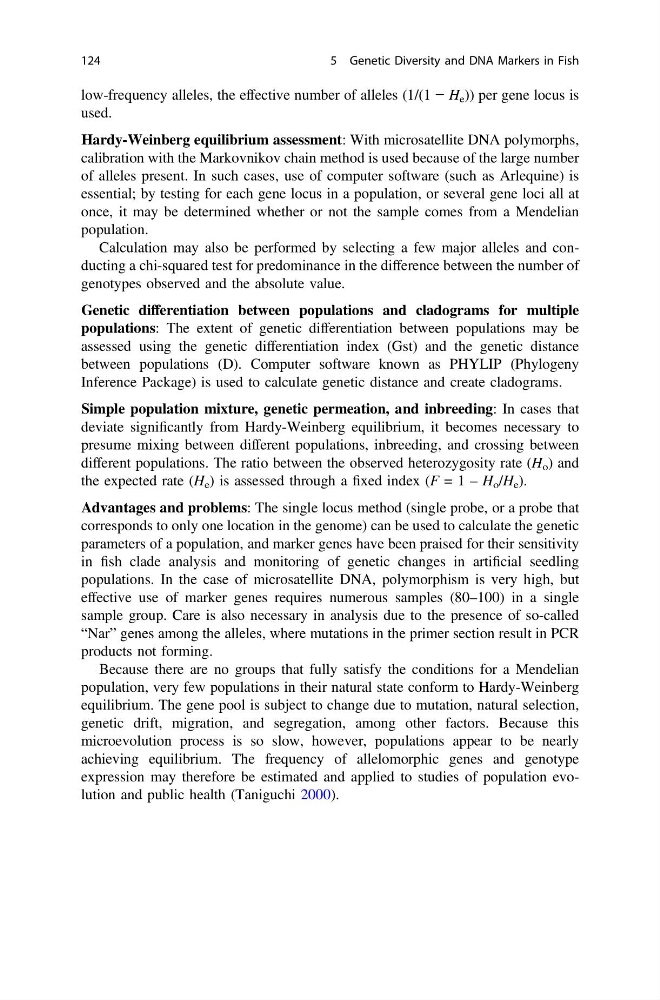
low-frequency alleles, the effective number of alleles (1/(1 − H e )) per gene locus is
used.
Hardy-Weinberg equilibrium assessment: With microsatellite DNA polymorphs,
calibration with the Markovnikov chain method is used because of the large number
of alleles present. In such cases, use of computer software (such as Arlequine) is
essential; by testing for each gene locus in a population, or several gene loci all at
once, it may be determined whether or not the sample comes from a Mendelian
population.
Calculation may also be performed by selecting a few major alleles and conducting a chi-squared test for predominance in the difference between the number of
genotypes observed and the absolute value.
Genetic differentiation between populations and cladograms for multiple
populations: The extent of genetic differentiation between populations may be
assessed using the genetic differentiation index (Gst) and the genetic distance
between populations (D). Computer software known as PHYLIP (Phylogeny
Inference Package) is used to calculate genetic distance and create cladograms.
Simple population mixture, genetic permeation, and inbreeding: In cases that
deviate significantly from Hardy-Weinberg equilibrium, it becomes necessary to
presume mixing between different populations, inbreeding, and crossing between
different populations. The ratio between the observed heterozygosity rate (H o ) and
the expected rate (H e ) is assessed through a fixed index (F = 1 – H o /H e ).
Advantages and problems: The single locus method (single probe, or a probe that
corresponds to only one location in the genome) can be used to calculate the genetic
parameters of a population, and marker genes have been praised for their sensitivity
in fish clade analysis and monitoring of genetic changes in artificial seedling
populations. In the case of microsatellite DNA, polymorphism is very high, but
effective use of marker genes requires numerous samples (80–100) in a single
sample group. Care is also necessary in analysis due to the presence of so-called
“Nar” genes among the alleles, where mutations in the primer section result in PCR
products not forming.
Because there are no groups that fully satisfy the conditions for a Mendelian
population, very few populations in their natural state conform to Hardy-Weinberg
equilibrium. The gene pool is subject to change due to mutation, natural selection,
genetic drift, migration, and segregation, among other factors. Because this
microevolution process is so slow, however, populations appear to be nearly
achieving equilibrium. The frequency of allelomorphic genes and genotype
expression may therefore be estimated and applied to studies of population evolution and public health (Taniguchi 2000).
124
5 Genetic Diversity and DNA Markers in Fish