

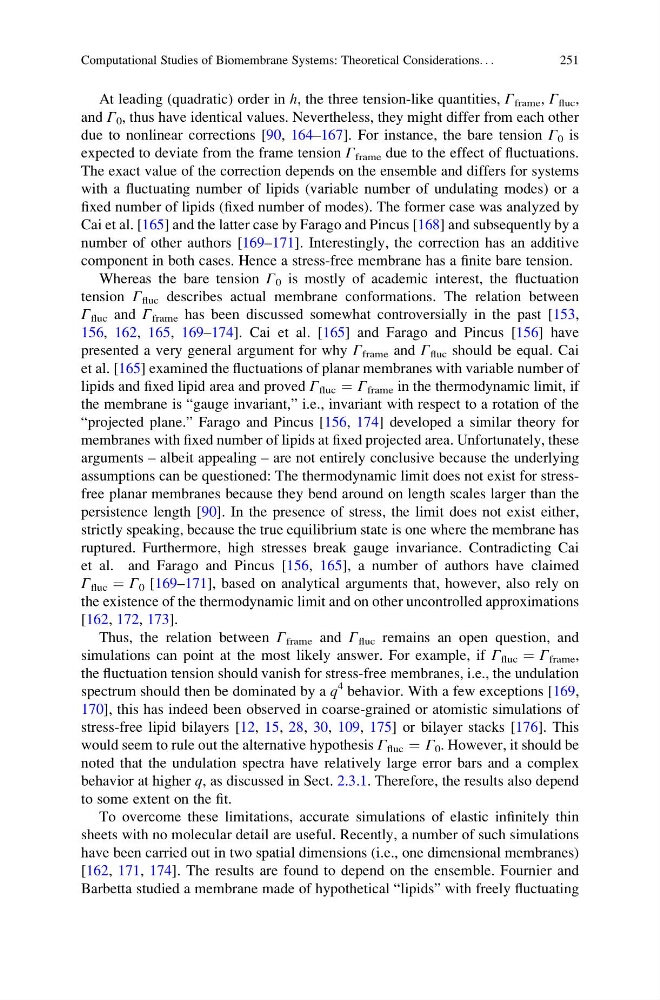
At leading (quadratic) order in h, the three tension-like quantities, Γ frame , Γ fluc ,
and Γ 0 , thus have identical values. Nevertheless, they might differ from each other
due to nonlinear corrections [90, 164–167]. For instance, the bare tension Γ 0 is
expected to deviate from the frame tension Γ frame due to the effect of fluctuations.
The exact value of the correction depends on the ensemble and differs for systems
with a fluctuating number of lipids (variable number of undulating modes) or a
fixed number of lipids (fixed number of modes). The former case was analyzed by
Cai et al. [165] and the latter case by Farago and Pincus [168] and subsequently by a
number of other authors [169–171]. Interestingly, the correction has an additive
component in both cases. Hence a stress-free membrane has a finite bare tension.
Whereas the bare tension Γ 0 is mostly of academic interest, the fluctuation
tension Γ fluc describes actual membrane conformations. The relation between
Γ fluc and Γ frame has been discussed somewhat controversially in the past [153,
156, 162, 165, 169–174]. Cai et al. [165] and Farago and Pincus [156] have
presented a very general argument for why Γ frame and Γ fluc should be equal. Cai
et al. [165] examined the fluctuations of planar membranes with variable number of
lipids and fixed lipid area and proved Γ fluc ¼ Γ frame in the thermodynamic limit, if
the membrane is “gauge invariant,” i.e., invariant with respect to a rotation of the
“projected plane.” Farago and Pincus [156, 174] developed a similar theory for
membranes with fixed number of lipids at fixed projected area. Unfortunately, these
arguments – albeit appealing – are not entirely conclusive because the underlying
assumptions can be questioned: The thermodynamic limit does not exist for stressfree planar membranes because they bend around on length scales larger than the
persistence length [90]. In the presence of stress, the limit does not exist either,
strictly speaking, because the true equilibrium state is one where the membrane has
ruptured. Furthermore, high stresses break gauge invariance. Contradicting Cai
et al. and Farago and Pincus [156, 165], a number of authors have claimed
Γ fluc ¼ Γ 0 [169–171], based on analytical arguments that, however, also rely on
the existence of the thermodynamic limit and on other uncontrolled approximations
[162, 172, 173].
Thus, the relation between Γ frame and Γ fluc remains an open question, and
simulations can point at the most likely answer. For example, if Γ fluc ¼ Γ frame ,
the fluctuation tension should vanish for stress-free membranes, i.e., the undulation
spectrum should then be dominated by a q
4 behavior. With a few exceptions [169,
170], this has indeed been observed in coarse-grained or atomistic simulations of
stress-free lipid bilayers [12, 15, 28, 30, 109, 175] or bilayer stacks [176]. This
would seem to rule out the alternative hypothesis Γ fluc ¼ Γ 0 . However, it should be
noted that the undulation spectra have relatively large error bars and a complex
behavior at higher q, as discussed in Sect. 2.3.1. Therefore, the results also depend
to some extent on the fit.
To overcome these limitations, accurate simulations of elastic infinitely thin
sheets with no molecular detail are useful. Recently, a number of such simulations
have been carried out in two spatial dimensions (i.e., one dimensional membranes)
[162, 171, 174]. The results are found to depend on the ensemble. Fournier and
Barbetta studied a membrane made of hypothetical “lipids” with freely fluctuating
Computational Studies of Biomembrane Systems: Theoretical Considerations. . .
251