

+ (or Mg
2+ ) ions [172]. From the functional standpoint, there are two types of
PQQ-containing DHs: those that are bound to the bacterial membrane (PQQ-As)
and those that are intracellular, and therefore water-soluble (PQQ-Bs). It has been
shown that they are distinct enzymes, with different molecular weights, substrate
specificity, optimal pH, and tolerance to heat. For example, the membrane-bound
glucose PQQGDH-A shows high selectivity for glucose; though, it requires suitable
detergents for solubilization [152, 153, 172]. In contrast, its water-soluble isoenzyme PQQGDH-B is not selective (catalyzes the oxidation of a variety of
monosaccharides and disaccharides) and is thermally unstable. On the other hand,
PQQGDH-B has a very high catalytic activity, which is over 25 times higher than
GOx’s activity [173]. Consequently, the interest in such active and O 2 -independent
enzymes for bioanalysis applications remained, and many studies based on protein
engineering techniques were done with success, resulting in the improvement of
water-soluble PQQGDH-B’s thermal stability [174–176] and narrowing its substrate specificity [177–179].
In recent years, a new type of fungi-derived thermostable FAD-dependent glucose dehydrogenases (FADGDHs) has been receiving particular attention, both in
the field of bioelectrochemistry and glucose biosensing. Tsujimura and Omura
found, for instance, a novel FAD-GDH from Aspergilus terreus, showing a high
thermostability, and specificity for glucose [180]. Since then, many other works
were published in the field, as recently reviewed by Okuda-Shimazakia et al. [181].
The main advantages of these FADGDHs are the high turnover rates and improved
substrate selectivity, good stability, and lower redox potentials [181].
Because flavin nucleotides and PQQ cofactors are embedded in the DHs
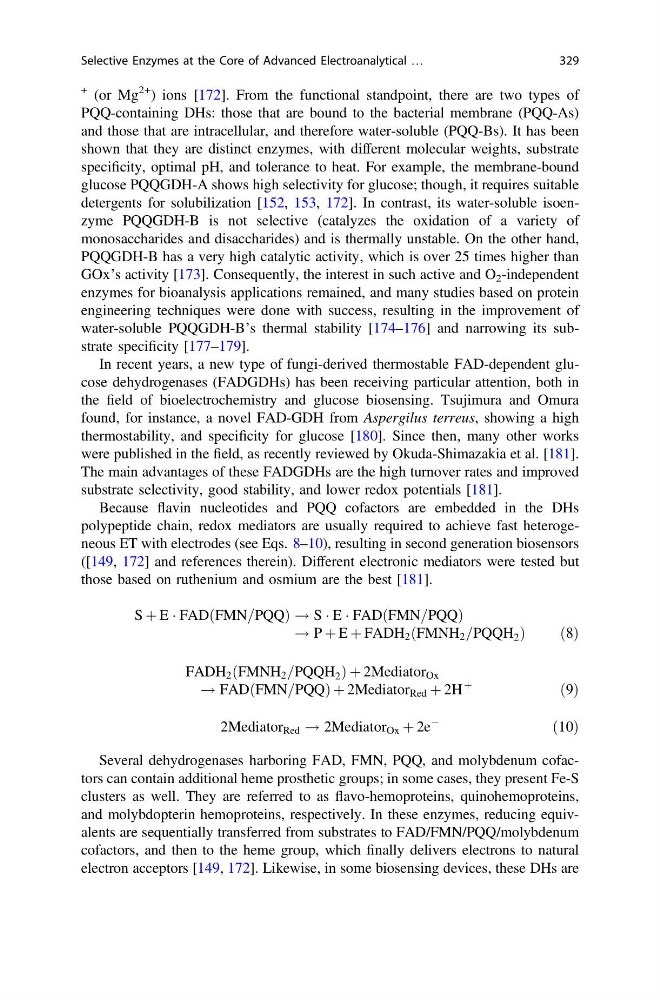
polypeptide chain, redox mediators are usually required to achieve fast heterogeneous ET with electrodes (see Eqs. 8–10), resulting in second generation biosensors
([149, 172] and references therein). Different electronic mediators were tested but
those based on ruthenium and osmium are the best [181].
S þ E Á FADðFMN=PQQÞ ! S Á E Á FADðFMN=PQQÞ
! P þ E þ FADH 2 ðFMNH 2 =PQQH 2 Þ
ð8Þ
FADH 2 ðFMNH 2 =PQQH 2 Þ þ 2Mediator Ox
! FADðFMN=PQQÞ þ 2Mediator Red þ 2H
þ
ð9Þ
2Mediator Red ! 2Mediator Ox þ 2e
À
ð10Þ
Several dehydrogenases harboring FAD, FMN, PQQ, and molybdenum cofactors can contain additional heme prosthetic groups; in some cases, they present Fe-S
clusters as well. They are referred to as flavo-hemoproteins, quinohemoproteins,
and molybdopterin hemoproteins, respectively. In these enzymes, reducing equivalents are sequentially transferred from substrates to FAD/FMN/PQQ/molybdenum
cofactors, and then to the heme group, which finally delivers electrons to natural
electron acceptors [149, 172]. Likewise, in some biosensing devices, these DHs are
Selective Enzymes at the Core of Advanced Electroanalytical …
329