

The archaeon Thermococcus onnurineus, also displays high activity in thermophilic conditions [91, 113–115]. Formate-driven H 2 production in this organism
occurs through a membrane-bound enzyme complex composed by an Fdh, a
hydrogenase and Na
+
/H
+ antiporter subunits that couples H 2 formation to formate
oxidation as well as energy conservation [115]. Under thermophilic conditions (80
ºC), Thermococcus onnurineus was able to reach the high hydrogen production of
404 mmol/g cells /h, which outcompete the ones obtained by dark fermentation [91].
Another microorganism with a great capacity for H 2 production from formate is
the strictly anaerobic acetogenic bacterium Acetobacterium woodii [96, 97, 116].
This bacterium possesses a new enzymatic system, the soluble hydrogen-dependent
CO 2 reductase complex (HDCR) that catalyzes the reversible oxidation of formate
to H 2 and CO 2 [116]. It was reported that whole-cells of A. woodii are capable of
producing 66 mmol/g cells /h of H 2 from formate [96].
3.2.2 Whole-Cell Biocatalysts for CO-Driven H 2 Production
Carbon monoxide-rich waste gases and syngas are considered as an interesting class
of substrates for biological H 2 production, allowing the simultaneous production of
fuel and the treatment of waste products. CO has a very low redox potential
(Eº = −520 mV) which makes it as great electron donor, although CO is toxic gas to
many microorganisms. Despite its toxicity, it has been reported that some microorganisms can use it as an energy and/or carbon source to produce H 2 [95, 102]. Efforts
have been made to isolate H 2 -producing microorganisms using CO as substrate, and
over the past decade the number of microorganisms known to be able to oxidize CO
duplicated [95, 102]. CO is biologically converted to H 2 according to the reaction:
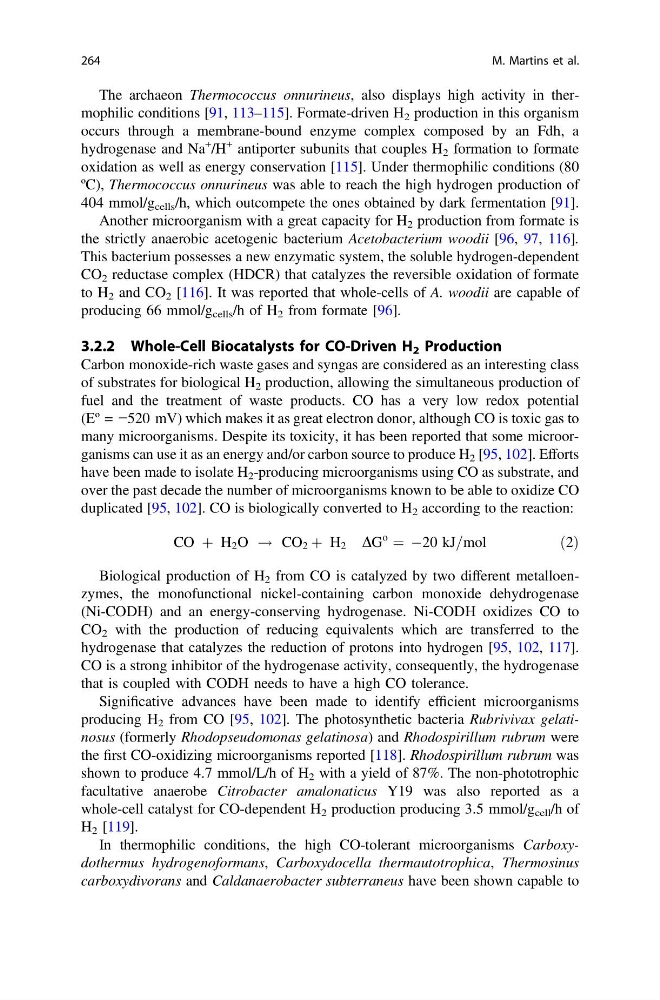
CO þ H 2 O ! CO 2 þ H 2 DG
o
¼ À20 kJ=mol
ð2Þ
Biological production of H 2 from CO is catalyzed by two different metalloenzymes, the monofunctional nickel-containing carbon monoxide dehydrogenase
(Ni-CODH) and an energy-conserving hydrogenase. Ni-CODH oxidizes CO to
CO 2 with the production of reducing equivalents which are transferred to the
hydrogenase that catalyzes the reduction of protons into hydrogen [95, 102, 117].
CO is a strong inhibitor of the hydrogenase activity, consequently, the hydrogenase
that is coupled with CODH needs to have a high CO tolerance.
Significative advances have been made to identify efficient microorganisms
producing H 2 from CO [95, 102]. The photosynthetic bacteria Rubrivivax gelatinosus (formerly Rhodopseudomonas gelatinosa) and Rhodospirillum rubrum were
the first CO-oxidizing microorganisms reported [118]. Rhodospirillum rubrum was
shown to produce 4.7 mmol/L/h of H 2 with a yield of 87%. The non-phototrophic
facultative anaerobe Citrobacter amalonaticus Y19 was also reported as a
whole-cell catalyst for CO-dependent H 2 production producing 3.5 mmol/g cell /h of
H 2 [119].
In thermophilic conditions, the high CO-tolerant microorganisms Carboxydothermus hydrogenoformans, Carboxydocella thermautotrophica, Thermosinus
carboxydivorans and Caldanaerobacter subterraneus have been shown capable to
264
M. Martins et al.