

400
9 Bioenergetics
gas has a pressure of p − − = 10 5 N/m 2 . For substances in solutions, the standard
state concentration, [C − − ], is one molar (one mole per liter).
In biochemical reactions, it is conventional to leave out certain concentrations in
the law of mass action that remain essentially constant, such as the concentration of
water in a cell, even when water takes part. We will expand on this topic later in this
Section.
If the concentrations of reactants and products do not represent equilibrium
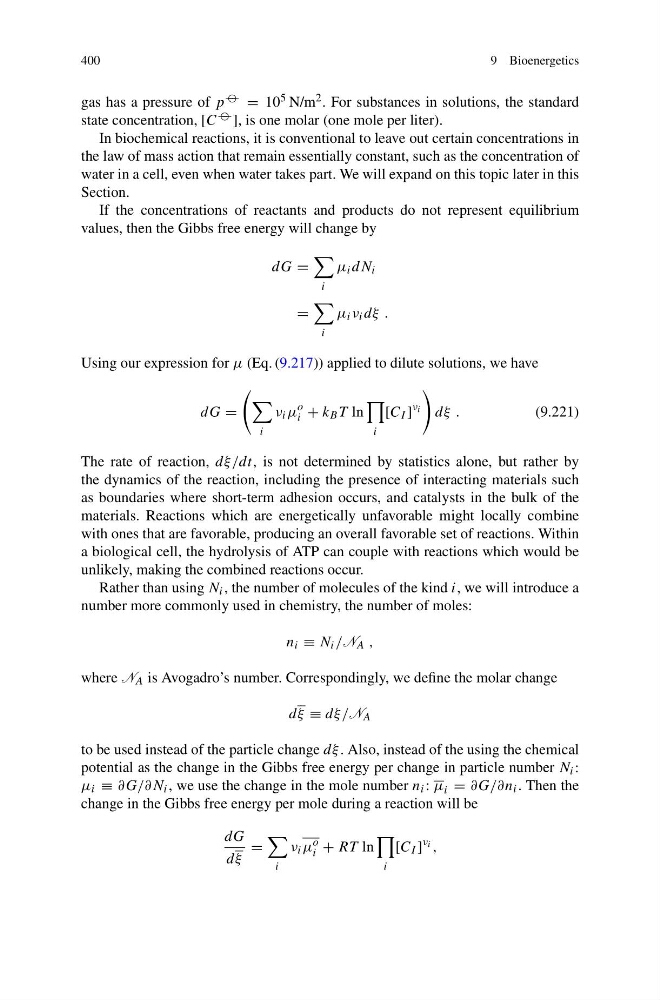
values, then the Gibbs free energy will change by
dG =
i
μ i dN i
=
i
μ i ν i dξ .
Using our expression for μ (Eq. (9.217)) applied to dilute solutions, we have
dG =
i
ν i μ
o
i + k B T ln
i
[C I ]
ν i
dξ .
(9.221)
The rate of reaction, dξ/dt, is not determined by statistics alone, but rather by
the dynamics of the reaction, including the presence of interacting materials such
as boundaries where short-term adhesion occurs, and catalysts in the bulk of the
materials. Reactions which are energetically unfavorable might locally combine
with ones that are favorable, producing an overall favorable set of reactions. Within
a biological cell, the hydrolysis of ATP can couple with reactions which would be
unlikely, making the combined reactions occur.
Rather than using N i , the number of molecules of the kind i, we will introduce a
number more commonly used in chemistry, the number of moles:
n i ≡ N i /N A ,
where N A is Avogadro’s number. Correspondingly, we define the molar change
dξ ≡ dξ/N A
to be used instead of the particle change dξ . Also, instead of the using the chemical
potential as the change in the Gibbs free energy per change in particle number N i :
μ i ≡ ∂G/∂N i , we use the change in the mole number n i : μ i = ∂G/∂n i . Then the
change in the Gibbs free energy per mole during a reaction will be
dG
dξ
=
i
ν i μ o
i + RT ln
i
[C I ]
ν i ,