

3
Can Allelopathic Interactions Assemble a Community?
In this section, the question if biological communities can emerge from allelopathy,
i.e., from competing interactions between their species mediated by toxins, is
addressed. Intuitively, this alternative faces a difficulty: multiple toxic environments
are the least expected to sustain species diversity.
3.1
An Eco-evolutionary Mathematical Model for Allelochemical
Networks
In order to discuss how community structures of populations enforced to
adapt and survive to the direct allelochemical suppression of each other are
affected by the evolutionary history of the interaction, Eqs. (1) or (3) can be
extended to include several species and to integrate ecological and evolutionary
processes. In such generalized models, the genetic diversity is generated by
mutations that induce changes in the allelochemical traits of the evolving
species, and selection is driven by ecological interactions, namely, intraand interspecific resource competition and allelopathic suppression. These
interactions determine how species evolve and enhance or diminish the
diversity of communities.
An example of this modeling strategy is the following model [35]. A set S of
l ℕ biological species with populations given by N
!
¼ N 1 , N 2 , :
ð
Þis considered. Every species in S synthesizes and releases toxic secondary
chemical compounds (microcins, fitotoxins, etc.) that enhance the mortality
of other species. The strengths of such interactions depend on the toxin concentration B
!
¼ B 1 , B 2 , . . .
ð
Þ and vary in time because B depends on the
abundance of species. Furthermore, the community assembly proceeds from
an initial subset S 0 S by randomly adding new species through mutationsfixed in a fraction of resident species offspring.
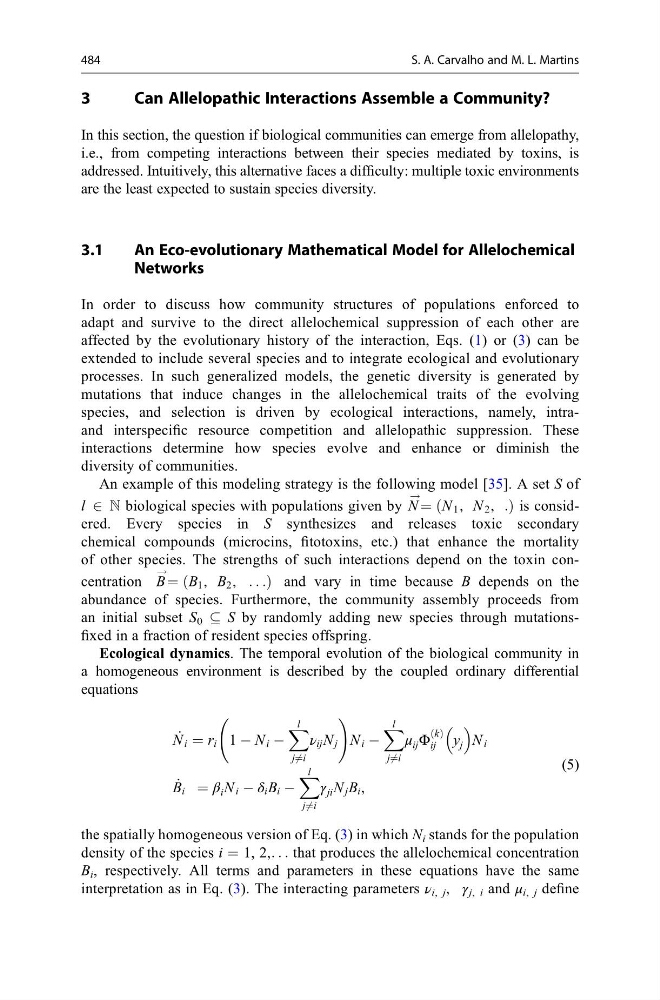
Ecological dynamics. The temporal evolution of the biological community in
a homogeneous environment is described by the coupled ordinary differential
equations
_
N i ¼ r i 1 À N i À
X l
j6 ¼i
ν ij N j
!
N i À
X l
j6 ¼i
μ ij Φ
k
ð Þ
ij
y j
N i
_
B i ¼ β i N i À δ i B i À
X l
j6 ¼i
γ ji N j B i ,
(5)
the spatially homogeneous version of Eq. (3) in which N i stands for the population
density of the species i = 1, 2,. . . that produces the allelochemical concentration
B i , respectively. All terms and parameters in these equations have the same
interpretation as in Eq. (3). The interacting parameters ν i, j , γ j, i and μ i, j define
484
S. A. Carvalho and M. L. Martins