

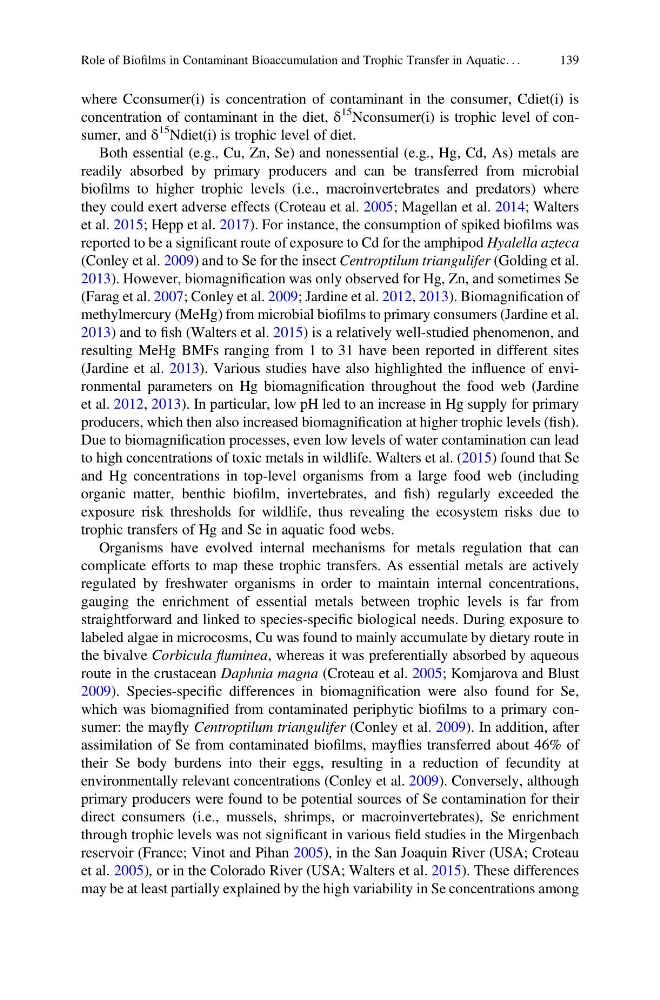
where Cconsumer(i) is concentration of contaminant in the consumer, Cdiet(i) is
concentration of contaminant in the diet, δ
15 Nconsumer(i) is trophic level of consumer, and δ
15 Ndiet(i) is trophic level of diet.
Both essential (e.g., Cu, Zn, Se) and nonessential (e.g., Hg, Cd, As) metals are
readily absorbed by primary producers and can be transferred from microbial
biofilms to higher trophic levels (i.e., macroinvertebrates and predators) where
they could exert adverse effects (Croteau et al. 2005; Magellan et al. 2014; Walters
et al. 2015; Hepp et al. 2017). For instance, the consumption of spiked biofilms was
reported to be a significant route of exposure to Cd for the amphipod Hyalella azteca
(Conley et al. 2009) and to Se for the insect Centroptilum triangulifer (Golding et al.
2013). However, biomagnification was only observed for Hg, Zn, and sometimes Se
(Farag et al. 2007; Conley et al. 2009; Jardine et al. 2012, 2013). Biomagnification of
methylmercury (MeHg) from microbial biofilms to primary consumers (Jardine et al.
2013) and to fish (Walters et al. 2015) is a relatively well-studied phenomenon, and
resulting MeHg BMFs ranging from 1 to 31 have been reported in different sites
(Jardine et al. 2013). Various studies have also highlighted the influence of environmental parameters on Hg biomagnification throughout the food web (Jardine
et al. 2012, 2013). In particular, low pH led to an increase in Hg supply for primary
producers, which then also increased biomagnification at higher trophic levels (fish).
Due to biomagnification processes, even low levels of water contamination can lead
to high concentrations of toxic metals in wildlife. Walters et al. (2015) found that Se
and Hg concentrations in top-level organisms from a large food web (including
organic matter, benthic biofilm, invertebrates, and fish) regularly exceeded the
exposure risk thresholds for wildlife, thus revealing the ecosystem risks due to
trophic transfers of Hg and Se in aquatic food webs.
Organisms have evolved internal mechanisms for metals regulation that can
complicate efforts to map these trophic transfers. As essential metals are actively
regulated by freshwater organisms in order to maintain internal concentrations,
gauging the enrichment of essential metals between trophic levels is far from
straightforward and linked to species-specific biological needs. During exposure to
labeled algae in microcosms, Cu was found to mainly accumulate by dietary route in
the bivalve Corbicula fluminea, whereas it was preferentially absorbed by aqueous
route in the crustacean Daphnia magna (Croteau et al. 2005; Komjarova and Blust
2009). Species-specific differences in biomagnification were also found for Se,
which was biomagnified from contaminated periphytic biofilms to a primary consumer: the mayfly Centroptilum triangulifer (Conley et al. 2009). In addition, after
assimilation of Se from contaminated biofilms, mayflies transferred about 46% of
their Se body burdens into their eggs, resulting in a reduction of fecundity at
environmentally relevant concentrations (Conley et al. 2009). Conversely, although
primary producers were found to be potential sources of Se contamination for their
direct consumers (i.e., mussels, shrimps, or macroinvertebrates), Se enrichment
through trophic levels was not significant in various field studies in the Mirgenbach
reservoir (France; Vinot and Pihan 2005), in the San Joaquin River (USA; Croteau
et al. 2005), or in the Colorado River (USA; Walters et al. 2015). These differences
may be at least partially explained by the high variability in Se concentrations among
Role of Biofilms in Contaminant Bioaccumulation and Trophic Transfer in Aquatic. . .
139