

Under this framework, stem taper is intimately related to both foliage shedding
and changes in the foliage distribution. Several factors that influence foliage distributions have been identified. Both stand (i.e. site fertility and stand density) and tree
level (i.e. tree size, age, and crown length) have been used to explain variations in
foliage distribution (Mäkelä and Vanninen 2001; Weiskittel et al. 2009; Schneider
et al. 2011b; Power et al. 2013; Williams et al. 2017). As illustrated in Schneider
et al. (2011a), a top-heavy foliage distribution will lead to a high sapwood area at
crown base whereas a bottom-heavy foliage distribution will have less sapwood
area, if the total crown foliage biomass is the same. This change in sapwood area
taper will lead to differences in stem taper. Nevertheless, this approach does not
integrate sapwood to heartwood turnover rates, as sapwood will not immediately
change into heartwood when the leaf is shed. The mechanisms underlying the
turnover are not well known, and most approaches rely on results obtained from
model simulations (e.g. Sievänen et al. 1997).
There has however been much debate on the validity of the pipe model theory
(Kershaw and Maguire 2000; Kershaw 2001; Valentine 2001; Sattler and Comeau
2015), if one considers sapwood area equivalent to the used pipe area. There is a lot
of evidence on the changes in sapwood conductivity in the radial direction (Domec
et al. 2006; Fiora and Cescatti 2008; Chang et al. 2014; Landsberg et al. 2017), and
might lead to ways of linking the theoretical pipes of the pipe model theory to
sapwood area.
4.2 Biomechanical Approaches
Tree stems are also used to support the crown in order to have access to the light
needed for photosynthesis. Biomechanics has thus also been used to explain tree
form. Metzger’s “d3” law was the first attempt to explain tree taper based on the
representation of a tree as a cantilever with constant stress along the stem (Metzger
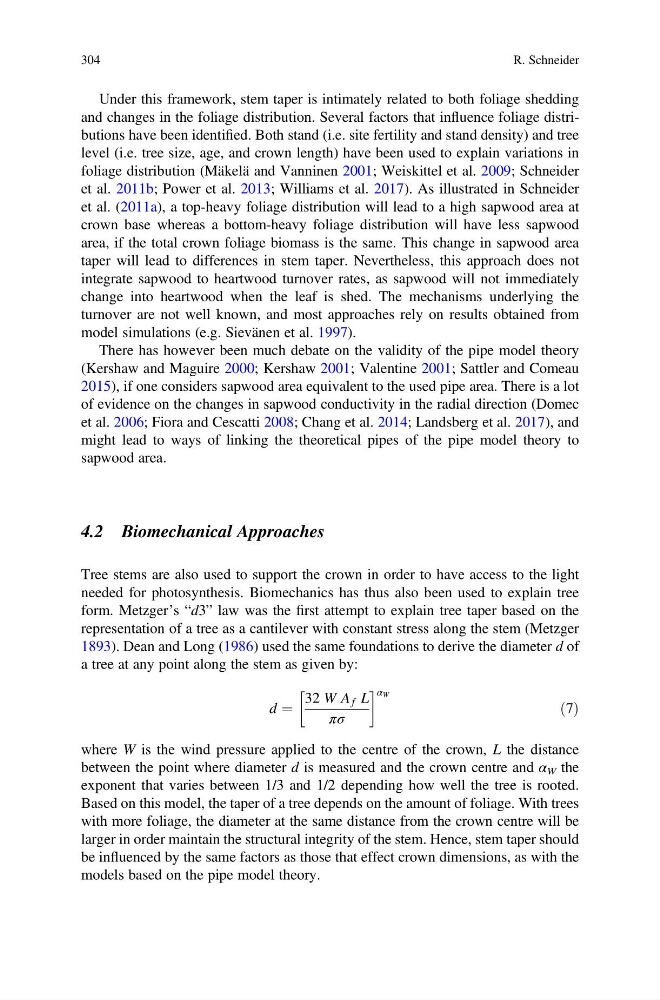
1893). Dean and Long (1986) used the same foundations to derive the diameter d of
a tree at any point along the stem as given by:
d ¼
32 W A f L
πσ
! α W
ð7Þ
where W is the wind pressure applied to the centre of the crown, L the distance
between the point where diameter d is measured and the crown centre and α W the
exponent that varies between 1/3 and 1/2 depending how well the tree is rooted.
Based on this model, the taper of a tree depends on the amount of foliage. With trees
with more foliage, the diameter at the same distance from the crown centre will be
larger in order maintain the structural integrity of the stem. Hence, stem taper should
be influenced by the same factors as those that effect crown dimensions, as with the
models based on the pipe model theory.
304
R. Schneider