

reducers of the Desulfosarcina/Desulfococcus group (Deltaproteobacteria)
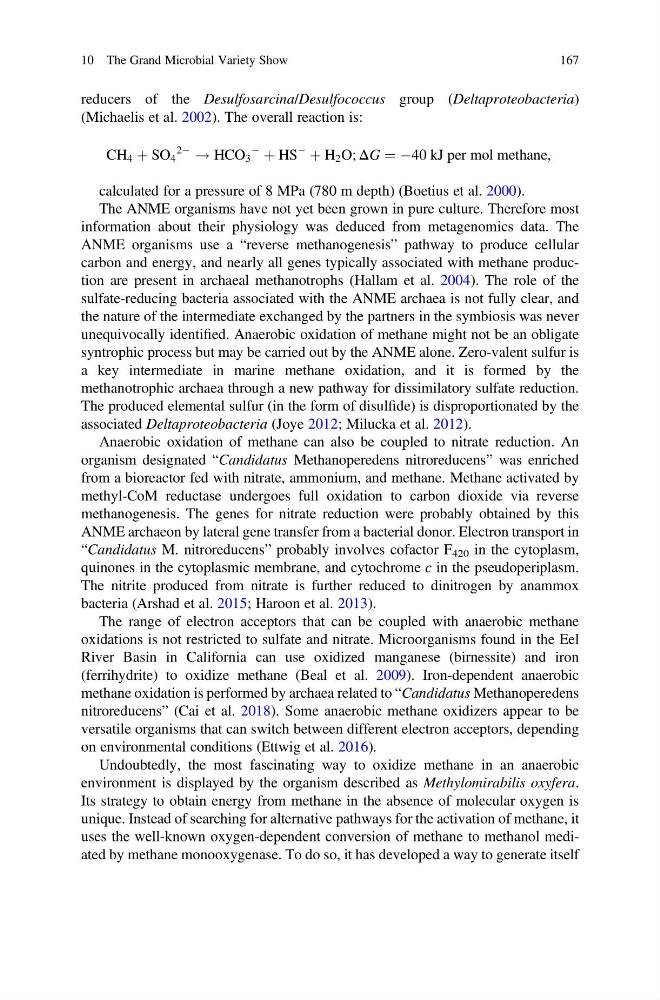
(Michaelis et al. 2002). The overall reaction is:
CH 4 þ SO 4
2À
! HCO 3
À
þ HS
À
þ H 2 O; ΔG ¼ À40 kJ per mol methane,
calculated for a pressure of 8 MPa (780 m depth) (Boetius et al. 2000).
The ANME organisms have not yet been grown in pure culture. Therefore most
information about their physiology was deduced from metagenomics data. The
ANME organisms use a “reverse methanogenesis” pathway to produce cellular
carbon and energy, and nearly all genes typically associated with methane production are present in archaeal methanotrophs (Hallam et al. 2004). The role of the
sulfate-reducing bacteria associated with the ANME archaea is not fully clear, and
the nature of the intermediate exchanged by the partners in the symbiosis was never
unequivocally identified. Anaerobic oxidation of methane might not be an obligate
syntrophic process but may be carried out by the ANME alone. Zero-valent sulfur is
a key intermediate in marine methane oxidation, and it is formed by the
methanotrophic archaea through a new pathway for dissimilatory sulfate reduction.
The produced elemental sulfur (in the form of disulfide) is disproportionated by the
associated Deltaproteobacteria (Joye 2012; Milucka et al. 2012).
Anaerobic oxidation of methane can also be coupled to nitrate reduction. An
organism designated “Candidatus Methanoperedens nitroreducens” was enriched
from a bioreactor fed with nitrate, ammonium, and methane. Methane activated by
methyl-CoM reductase undergoes full oxidation to carbon dioxide via reverse
methanogenesis. The genes for nitrate reduction were probably obtained by this
ANME archaeon by lateral gene transfer from a bacterial donor. Electron transport in
“Candidatus M. nitroreducens” probably involves cofactor F 420 in the cytoplasm,
quinones in the cytoplasmic membrane, and cytochrome c in the pseudoperiplasm.
The nitrite produced from nitrate is further reduced to dinitrogen by anammox
bacteria (Arshad et al. 2015; Haroon et al. 2013).
The range of electron acceptors that can be coupled with anaerobic methane
oxidations is not restricted to sulfate and nitrate. Microorganisms found in the Eel
River Basin in California can use oxidized manganese (birnessite) and iron
(ferrihydrite) to oxidize methane (Beal et al. 2009). Iron-dependent anaerobic
methane oxidation is performed by archaea related to “Candidatus Methanoperedens
nitroreducens” (Cai et al. 2018). Some anaerobic methane oxidizers appear to be
versatile organisms that can switch between different electron acceptors, depending
on environmental conditions (Ettwig et al. 2016).
Undoubtedly, the most fascinating way to oxidize methane in an anaerobic
environment is displayed by the organism described as Methylomirabilis oxyfera.
Its strategy to obtain energy from methane in the absence of molecular oxygen is
unique. Instead of searching for alternative pathways for the activation of methane, it
uses the well-known oxygen-dependent conversion of methane to methanol mediated by methane monooxygenase. To do so, it has developed a way to generate itself
10 The Grand Microbial Variety Show
167