

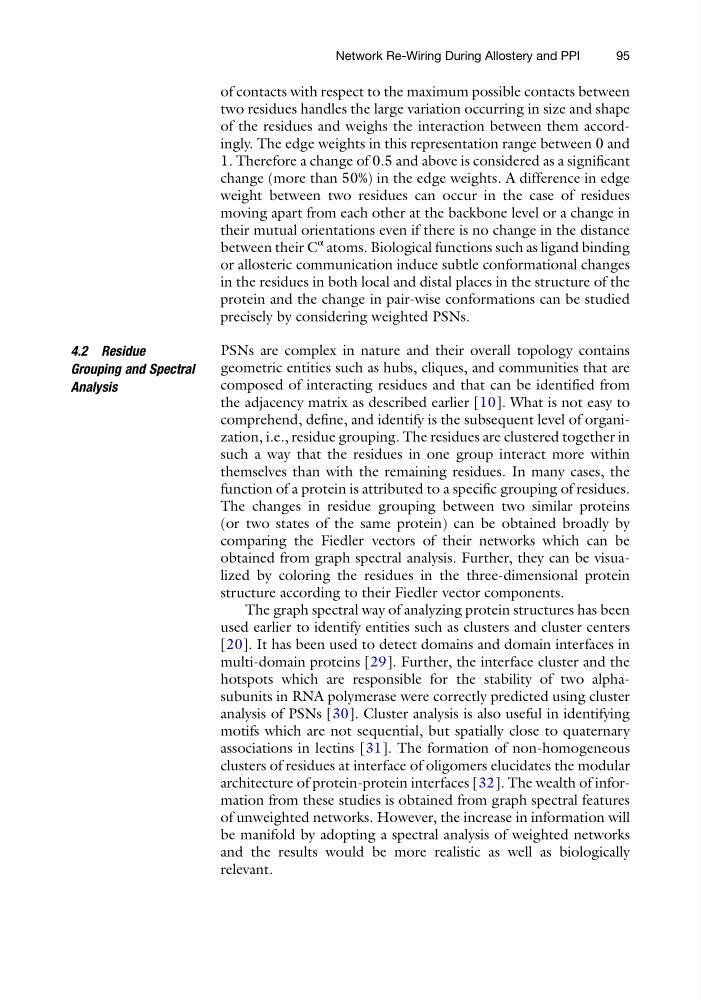
of contacts with respect to the maximum possible contacts between
two residues handles the large variation occurring in size and shape
of the residues and weighs the interaction between them accordingly. The edge weights in this representation range between 0 and
1. Therefore a change of 0.5 and above is considered as a significant
change (more than 50%) in the edge weights. A difference in edge
weight between two residues can occur in the case of residues
moving apart from each other at the backbone level or a change in
their mutual orientations even if there is no change in the distance
between their C
α atoms. Biological functions such as ligand binding
or allosteric communication induce subtle conformational changes
in the residues in both local and distal places in the structure of the
protein and the change in pair-wise conformations can be studied
precisely by considering weighted PSNs.
4.2 Residue
Grouping and Spectral
Analysis
PSNs are complex in nature and their overall topology contains
geometric entities such as hubs, cliques, and communities that are
composed of interacting residues and that can be identified from
the adjacency matrix as described earlier [10]. What is not easy to
comprehend, define, and identify is the subsequent level of organization, i.e., residue grouping. The residues are clustered together in
such a way that the residues in one group interact more within
themselves than with the remaining residues. In many cases, the
function of a protein is attributed to a specific grouping of residues.
The changes in residue grouping between two similar proteins
(or two states of the same protein) can be obtained broadly by
comparing the Fiedler vectors of their networks which can be
obtained from graph spectral analysis. Further, they can be visualized by coloring the residues in the three-dimensional protein
structure according to their Fiedler vector components.
The graph spectral way of analyzing protein structures has been
used earlier to identify entities such as clusters and cluster centers
[20]. It has been used to detect domains and domain interfaces in
multi-domain proteins [29]. Further, the interface cluster and the
hotspots which are responsible for the stability of two alphasubunits in RNA polymerase were correctly predicted using cluster
analysis of PSNs [30]. Cluster analysis is also useful in identifying
motifs which are not sequential, but spatially close to quaternary
associations in lectins [31]. The formation of non-homogeneous
clusters of residues at interface of oligomers elucidates the modular
architecture of protein-protein interfaces [32]. The wealth of information from these studies is obtained from graph spectral features
of unweighted networks. However, the increase in information will
be manifold by adopting a spectral analysis of weighted networks
and the results would be more realistic as well as biologically
relevant.
Network Re-Wiring During Allostery and PPI
95