

60
P. Sjödin et al.
from the same subpopulation to find a common ancestor. The intuition for this
definition is that it measures the relatively longer time it takes for two genes situated
in individuals from different subpopulations to find a common ancestor compared
to when they are situated in individuals from the same subpopulation. From this
definition, it is clear that if the expected coalescent time for two genes does not
depend on which population the genes are drawn from (t s = t w ), then F ST = 0. In
contrast, if genes from different populations take much longer to find a common
ancestor than genes from the same population, F ST tends toward 1.
In order to estimate F ST , we need genetic variation from individuals drawn from
predefined populations. Depending on the type of genetic data, different assumptions of the mutational process can be used. For sequence data, the mutational
process is well approximated by the infinite sites model, for which at most one
mutation is allowed for each site. The mutation rate per site is typically very low
and the influence of branch-specific, novel mutations when estimating F ST will
be assumed to be negligible compared to demographic factors that affect sites
polymorphic in the ancestral population to the predefined populations. Alternatively,
an outgroup can be utilized to delimit the data to SNPs that were polymorphic
prior to the time period of interest. In order to account for the sample variance
(due to limited sample sizes), Weir and Cockerham (1984) developed a robust (and
commonly used) estimator for F ST (see also Weir 1996; Bhatia et al. 2013).
Model-specific demographic parameters such as migration rate and/or divergence
time can often be directly related to F ST , although caution is warranted for directly
equating an F ST estimate with a specific demographic parameter as there are many
different factors that influence estimates of F ST . For instance, in a two-population
divergence model, the relationship between F ST and the divergence time t is (Slatkin
1995):
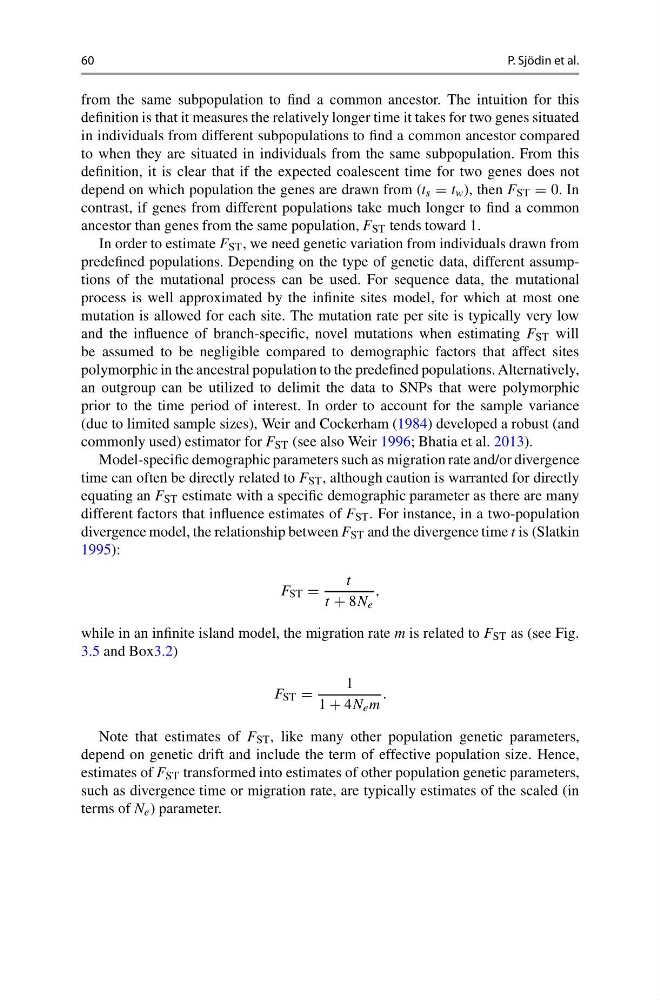
F ST =
t
t + 8N e
,
while in an infinite island model, the migration rate m is related to F ST as (see Fig.
3.5 and Box3.2)
F ST =
1
1 + 4N e m
.
Note that estimates of F ST , like many other population genetic parameters,
depend on genetic drift and include the term of effective population size. Hence,
estimates of F ST transformed into estimates of other population genetic parameters,
such as divergence time or migration rate, are typically estimates of the scaled (in
terms of N e ) parameter.