

6
J. Wakeley
model for a single locus without recombination are presented and explained. The
presentation begins with the idea that gene genealogies are embedded within
organismal pedigrees. Although this is not a controversial idea, it is not, in fact,
how gene genealogies are modeled in standard coalescent derivations.
1.2.1 Organismal Pedigrees and Gene Genealogies
Within any sexually reproducing species, such as humans, there exists a pattern of
ancestry and descent which we may call the population pedigree. If it were known,
the population pedigree would be a record of all reproduction events, connecting
parents with their offspring and extending from the distant past to the present day.
It would reflect the movement of individuals across the globe, changes in local
population sizes over time, and events such as the selective sweeps of advantageous
alleles through the population. Like the gene genealogy, the population pedigree
is an unknown but important outcome of the population-level processes which
affect genetic variation. Further, the gene genealogy at a locus without intra-locus
recombination is simply the result of Mendelian segregation within the parts of the
population pedigree relating to the sampled individuals.
The derivations of coalescent theory average over the unknown population
pedigree within each generation, with details depending on the reproduction form
assumed. For example, consider the probability that two gene copies or alleles
at an autosomal locus, obtained by randomly sampling two individuals from the
population without replacement, are descended from a common ancestor (i.e., they
“coalesce”) in the immediately previous generation. This quantity, which we may
call c N following Möhle (1998a) is fundamental in coalescent theory because it sets
the timescale of the coalescent process. Under the diploid, dioecious Wright–Fisher
model (Fisher 1930; Wright 1931) with random mating between the two sexes, we
have
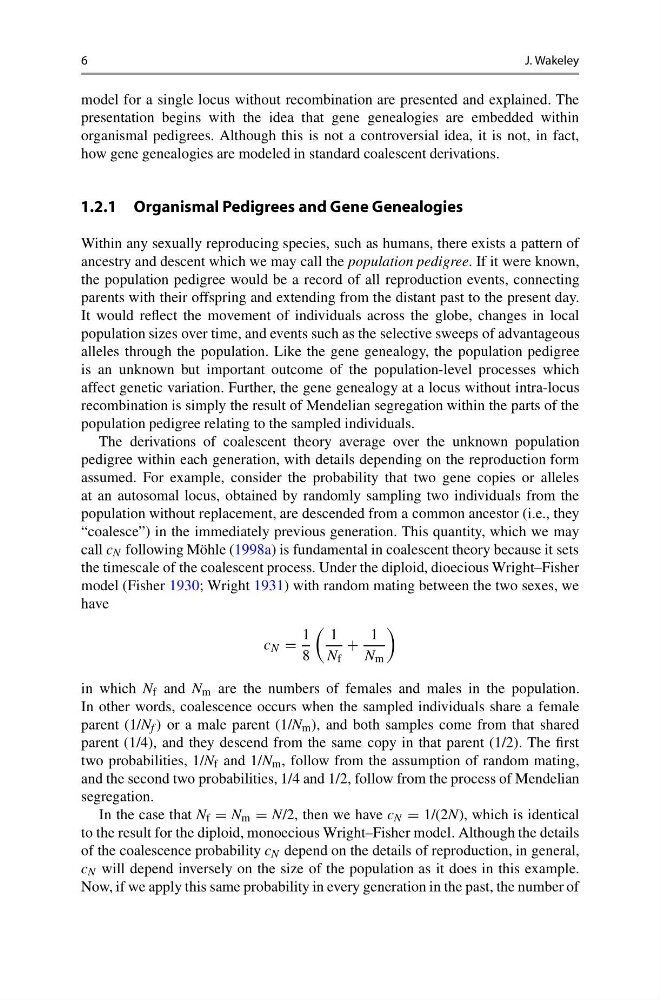
c N =
1
8
1
N f
+
1
N m
in which N f and N m are the numbers of females and males in the population.
In other words, coalescence occurs when the sampled individuals share a female
parent (1/N f ) or a male parent (1/N m ), and both samples come from that shared
parent (1/4), and they descend from the same copy in that parent (1/2). The first
two probabilities, 1/N f and 1/N m , follow from the assumption of random mating,
and the second two probabilities, 1/4 and 1/2, follow from the process of Mendelian
segregation.
In the case that N f = N m = N/2, then we have c N = 1/(2N), which is identical
to the result for the diploid, monoecious Wright–Fisher model. Although the details
of the coalescence probability c N depend on the details of reproduction, in general,
c N will depend inversely on the size of the population as it does in this example.
Now, if we apply this same probability in every generation in the past, the number of