

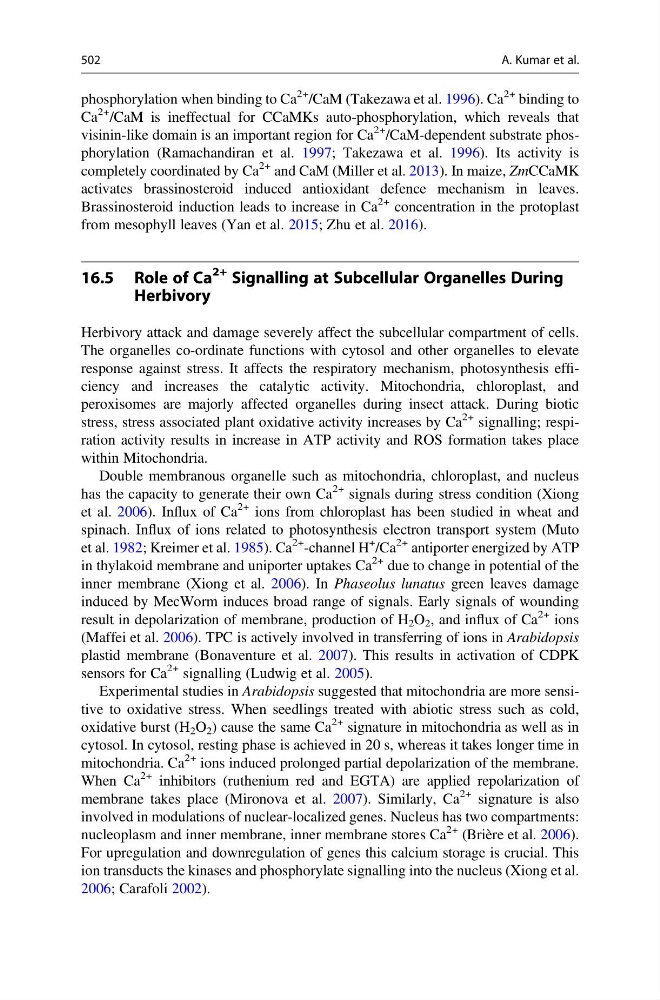
phosphorylation when binding to Ca
2+ /CaM (Takezawa et al. 1996). Ca
2+ binding to
Ca
2+ /CaM is ineffectual for CCaMKs auto-phosphorylation, which reveals that
visinin-like domain is an important region for Ca
2+ /CaM-dependent substrate phosphorylation (Ramachandiran et al. 1997; Takezawa et al. 1996). Its activity is
completely coordinated by Ca
2+ and CaM (Miller et al. 2013). In maize, ZmCCaMK
activates brassinosteroid induced antioxidant defence mechanism in leaves.
Brassinosteroid induction leads to increase in Ca
2+ concentration in the protoplast
from mesophyll leaves (Yan et al. 2015; Zhu et al. 2016).
16.5 Role of Ca
2+ Signalling at Subcellular Organelles During
Herbivory
Herbivory attack and damage severely affect the subcellular compartment of cells.
The organelles co-ordinate functions with cytosol and other organelles to elevate
response against stress. It affects the respiratory mechanism, photosynthesis efficiency and increases the catalytic activity. Mitochondria, chloroplast, and
peroxisomes are majorly affected organelles during insect attack. During biotic
stress, stress associated plant oxidative activity increases by Ca
2+ signalling; respiration activity results in increase in ATP activity and ROS formation takes place
within Mitochondria.
Double membranous organelle such as mitochondria, chloroplast, and nucleus
has the capacity to generate their own Ca
2+ signals during stress condition (Xiong
et al. 2006). Influx of Ca
2+ ions from chloroplast has been studied in wheat and
spinach. Influx of ions related to photosynthesis electron transport system (Muto
et al. 1982; Kreimer et al. 1985). Ca
2+ -channel H
+
/Ca
2+ antiporter energized by ATP
in thylakoid membrane and uniporter uptakes Ca
2+ due to change in potential of the
inner membrane (Xiong et al. 2006). In Phaseolus lunatus green leaves damage
induced by MecWorm induces broad range of signals. Early signals of wounding
result in depolarization of membrane, production of H 2 O 2 , and influx of Ca
2+ ions
(Maffei et al. 2006). TPC is actively involved in transferring of ions in Arabidopsis
plastid membrane (Bonaventure et al. 2007). This results in activation of CDPK
sensors for Ca
2+ signalling (Ludwig et al. 2005).
Experimental studies in Arabidopsis suggested that mitochondria are more sensitive to oxidative stress. When seedlings treated with abiotic stress such as cold,
oxidative burst (H 2 O 2 ) cause the same Ca
2+ signature in mitochondria as well as in
cytosol. In cytosol, resting phase is achieved in 20 s, whereas it takes longer time in
mitochondria. Ca
2+ ions induced prolonged partial depolarization of the membrane.
When Ca
2+ inhibitors (ruthenium red and EGTA) are applied repolarization of
membrane takes place (Mironova et al. 2007). Similarly, Ca
2+ signature is also
involved in modulations of nuclear-localized genes. Nucleus has two compartments:
nucleoplasm and inner membrane, inner membrane stores Ca
2+ (Brière et al. 2006).
For upregulation and downregulation of genes this calcium storage is crucial. This
ion transducts the kinases and phosphorylate signalling into the nucleus (Xiong et al.
2006; Carafoli 2002).
502
A. Kumar et al.