

190
C. ALBERS
hemoglobin content and the C 0 2 combining power. The reason for this
as well as for the effects of oxygenation and deoxygenation will be discussed below.
It seems necessary to stress the narrow range of CO, tensions encountered under physiological conditions. Generally the arterial pco, is
about 1-2 torr only and the venous pco, rarely exceeds 10 torr. In vitro
investigations of the CO, transport should concentrate largely on this
range. Equilibrium of fish blood with CO, tensions as high as 70 torr
as done in the early papers in this field does not seem to provide useful
information.
1. PHYSICALLY DISSOLVED COz
If the partial pressure of CO, is known, the amount of physically dissolved CO, can be calculated with the aid of the solubility coefficient S
[see Eq. (S)]. Whereas values of S are well established for mammalian
blood, there are almost no data reported on fish blood. In the case of
marine fish some authors simply use the solubility of C 0 2 in the surrounding seawater. Since the ionic composition and the ionic strength
of fish plasma displays a fairly large variability, it is highly dcsirable
to obtain reliable data for S especially if the Henderson-Hasselbalch
equation is to be used. If approximations of S are applied, the results
of such calculations are jeopardized by substantial errors.
Reaction (9a)
CO, + Hz0 HzCOS
as a molecular reaction proceeds very slowly. The time needed for full
equilibrium is about 200 times longer than the time spent by the blood
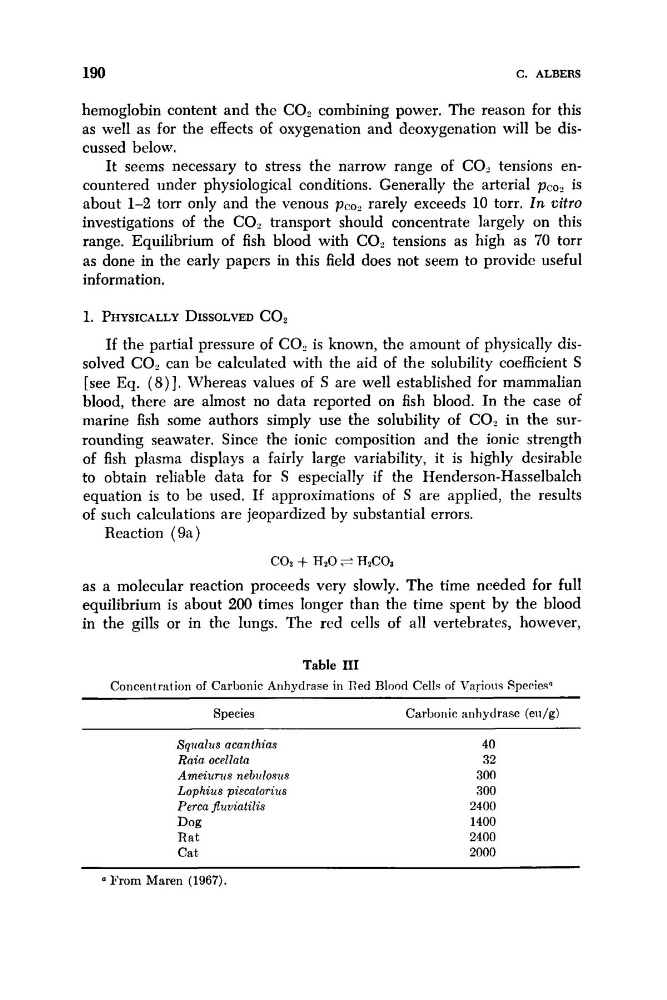
in the gills or in the lungs. The red cells of all vertebrates, however,
Table I11
Concentration of Carbonic Anhydrase in Xed Blood Cells of Various Speries'
Species
Carbonic arihydrase (en/g)
Sqiialus acanthias
Raia owllala
Ameizinis nebirloszis
Lophius piecatorius
Perca jluvialilis
Dog
R a t
Cat
40
32
300
300
2400
1400
2400
2000
From Maren (1967).