

3 90
a. B. COWEY AND J. R. SAFLQENT
that they were totally depleted. Thus Morgulis (1918), cited by
Gerking, found no stabilization of nitrogen excretion in brook trout
following a four week fast. With this reservation Gerking showed that
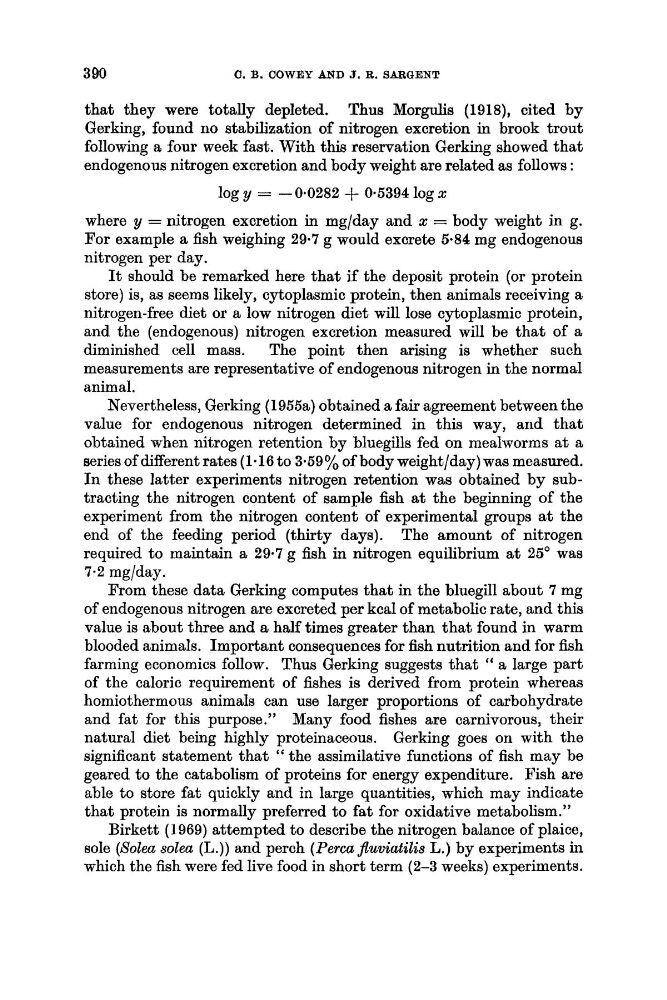
endogenous nitrogen excretion and body weight are related as follows :
log y = -0.0282 + 0.5394 log x
where y = nitrogen excretion in mg/day and x = body weight in g.
For example a fish weighing 29.7 g would excrete 5.84 mg endogenous
nitrogen per day.
It should be remarked here that if the deposit protein (or protein
store) is, as seems likely, cytoplasmic protein, then animals receiving a
nitrogen-free diet or a low nitrogen diet will lose cytoplasmic protein,
and the (endogenous) nitrogen excretion measured will be that of a
diminished cell mass. The point then arising is whether such
measurements are representative of endogenous nitrogen in the normal
animal.
Nevertheless, Gerking (1955a) obtained a fair agreement between the
value for endogenous nitrogen determined in this way, and that
obtained when nitrogen retention by bluegills fed on rnealworms at a
series of different rates (1.16 to 3.59% of body weight/day) was measured.
In these latter experiments nitrogen retention was obtained by subtracting the nitrogen content of sample fish at the beginning of the
experiment from the nitrogen content of experimental groups at the
end of the feeding period (thirty days). The amount of nitrogen
required to maintain a 29.7 g fish in nitrogen equilibrium at 25’ was
7.2 mglday.
From these data Gerking computes that in the bluegill about 7 mg
of endogenous nitrogen are excreted per kcal of metabolic rate, and this
value is about three and a, half times greater than that found in warm
blooded animals. Important consequences for fish nutrition and for fish
farming economics follow. Thus Gerking suggests that “ a large part
of the caloric requirement of fishes is derived from protein whereas
homiothermous animals can use larger proportions of carbohydrate
and fat for this purpose.” Many food fishes are carnivorous, their
natural diet being highly proteinaceous. Gerking goes on with the
significant statement that “ the assimilative functions of fish may be
geared to the catabolism of proteins for energy expenditure. Fish are
able to store fat quickly and in large quantities, which may indicate
that protein is normally preferred to fat for oxidative metabolism.”
Birkett (1969) attempted to describe the nitrogen balance of plaice,
sole (Solea solea (L.)) and perch (Perm Jluviatilis L.) by experiments in
which the fish were fed live food in short term (2-3 weeks) experiments.