

162
J . E. a. RAYMONT
Antarctic areas the grazing activity was so intense that the standing
crop was only 0.5% of the calculated productions. A number of workers
(Riley, 1946; Gauld, 1950; Cushing, 1950a and b; Mare, 1940) have
noticed the relatively small standing crop of plant plankton when zooplankton density is high. But the time relations between phytoplankton
and zooplankton growth must be remembered; a zooplankton population can graze down plant cells in a matter of a few days, although the
animals grow and reproduce more slowly. On the other hand, a relatively
small algal population can reproduce exceedingly quickly, and thus
with good growth conditions and in absence of grazers, can become a
very dense population in a few days. The importance of this time factor
in phytoplankton/zooplankton relationships has been well emphasized
by both Steemann Nielsen (1937, 1963) and Clarke (1939).
The importance of grazing as a factor in phytoplankton production
has led to a number of mathematical treatments. Fleming (1939) expressed the difference between an initial population of phytoplankton
and the population at some time interval as the “increment”. Clearly
total production can be equivalent to increment only if no death of
cells or removal by grazing occurs. Most workers agree that relatively
little natural mortality of algal phytoplankton normally occurs, but an
animal population may remove a considerable proportion of the phytoplankton by grazing. Fleming proposed the term “yield” for the difference between the total production and the increment, assuming that the
difference was due to the removal of algae by zooplankton alone.
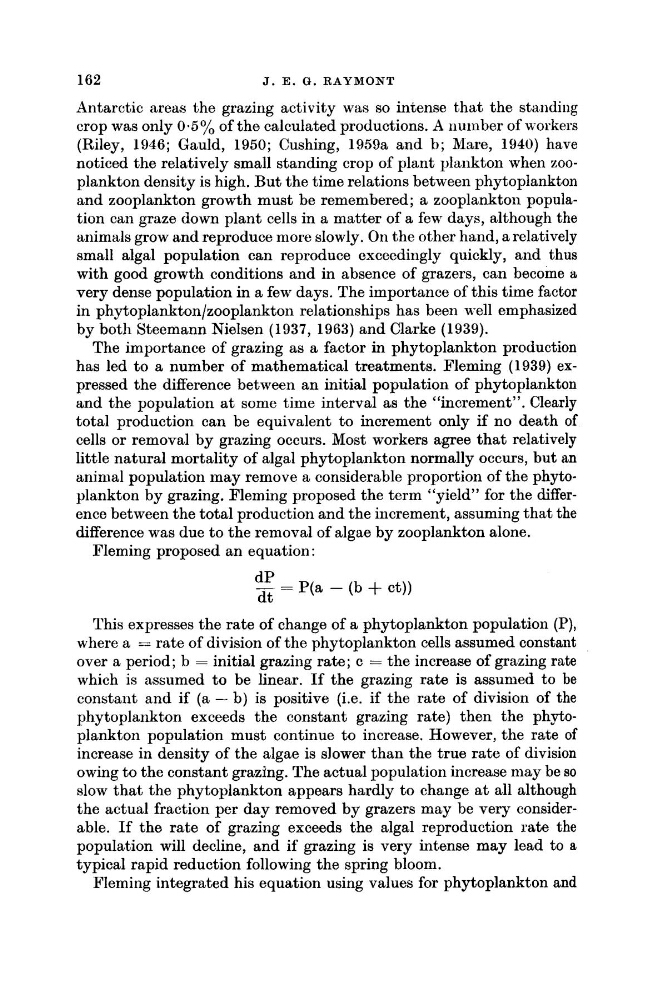
Fleming proposed an equation :
- _ - P(a - (b + ct))
d P
dt
This expresses the rate of change of a phytoplankton population (P),
where a = rate of division of the phytoplankton cells assumed constant
over a period; b = initial grazing rate; c = the increase of grazing rate
which is assumed to be linear. If the grazing rate is assumed t o be
constant and if (a - b) is positive (i.e. if the rate of division of the
phytoplankton exceeds the constant grazing rate) then the phytoplankton population must continue to increase. However, the rate of
increase in density of the algae is slower than the true rate of division
owing to the constant grazing. The actual population increase may be so
slow that the phytoplankton appears hardly to change a t all although
the actual fraction per day removed by grazers may be very considerable. If the rate of grazing exceeds the algal reproduction rate the
population will decline, and if grazing is very intense may lead to a
typical rapid reduction following the spring bloom.
Fleming integrated his equation using values for phytoplankton and