

9. SACCHARIDES: ALTERNATE ROUTES OF METABOLISM
455
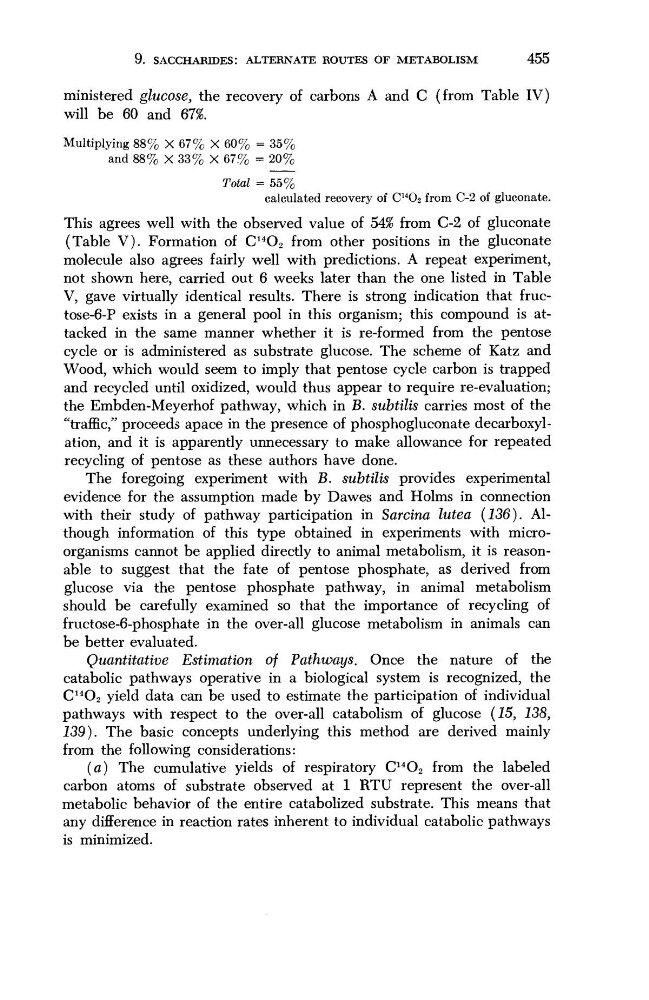
ministered glucose, the recovery of carbons A and C (from Table IV)
will be 60 and 671
Multiplying 88% X 67% X 60% = 35%
and 88% X 33% X 67.% = 20%
Total = 55%
calculated recovery of C
14 0 2 from C-2 of gluconate.
This agrees well with the observed value of 54% from C-2 of gluconate
(Table V). Formation of C
14 0 2 from other positions in the gluconate
molecule also agrees fairly well with predictions. A repeat experiment,
not shown here, carried out 6 weeks later than the one listed in Table
V, gave virtually identical results. There is strong indication that fructose-6-P exists in a general pool in this organism; this compound is attacked in the same manner whether it is re-formed from the pentose
cycle or is administered as substrate glucose. The scheme of Katz and
Wood, which would seem to imply that pentose cycle carbon is trapped
and recycled until oxidized, would thus appear to require re-evaluation;
the Embden-Meyerhof pathway, which in B. subtilis carries most of the
"traffic," proceeds apace in the presence of phosphogluconate decarboxylation, and it is apparently unnecessary to make allowance for repeated
recycling of pentose as these authors have done.
The foregoing experiment with B. subtilis provides experimental
evidence for the assumption made by Dawes and Holms in connection
with their study of pathway participation in Sarcina lutea (136). Although information of this type obtained in experiments with microorganisms cannot be applied directly to animal metabolism, it is reasonable to suggest that the fate of pentose phosphate, as derived from
glucose via the pentose phosphate pathway, in animal metabolism
should be carefully examined so that the importance of recycling of
fructose-6-phosphate in the over-all glucose metabolism in animals can
be better evaluated.
Quantitative Estimation of Pathways. Once the nature of the
catabolic pathways operative in a biological system is recognized, the
C
14 0 2 yield data can be used to estimate the participation of individual
pathways with respect to the over-all catabolism of glucose (15, 138,
139). The basic concepts underlying this method are derived mainly
from the following considerations:
(a) The cumulative yields of respiratory C
14 0 2 from the labeled
carbon atoms of substrate observed at 1 RTU represent the over-all
metabolic behavior of the entire catabolized substrate. This means that
any difference in reaction rates inherent to individual catabolic pathways
is minimized.