

8.1.2 The Underwater Light Field
The wavelength dependence of biological responses to light is well established.
The relationship varies from the induction of photosynthetic activity by PAR (400 –
700 nm) to the induction of repair enzymes (or production of UVR-screening pigments)
during exposure to component bands of ultraviolet–A radiation (UV-A, 315 – 400 nm)
(Corredor, et al. 2000) or to direct photochemical damage to DNA by ultraviolet–B
radiation (UV-B, 280 – 315 nm) (Lyons, et al. 1998). Due to the complexity of coral
responses to light, a number of studies aimed at investigating the relationship between
different spectral regions and coral bleaching have been undertaken (Gleason and
Wellington 1993, Fitt and Warner 1995). In these studies, both the density of
zooxanthellae cells and the concentration of chlorophyll in zooxanthellae showed
significant reductions with increasing UVR and visible light intensity.
UV and blue light penetration in shallow oligotrophic environments, with
chlorophyll a concentrations of less than 0.5 mg/m
3 , is largely controlled by CDOM
(Markager and Vincent 2000, Nelson and Siegel 2002). This macromolecular mixture
of organic molecules contains a complex array of unidentified chromophores with
overlapping absorbance spectra (Stabenau and Zika 2004). The mixture is often
characterized by its exponential increase in absorbance with decreasing wavelength
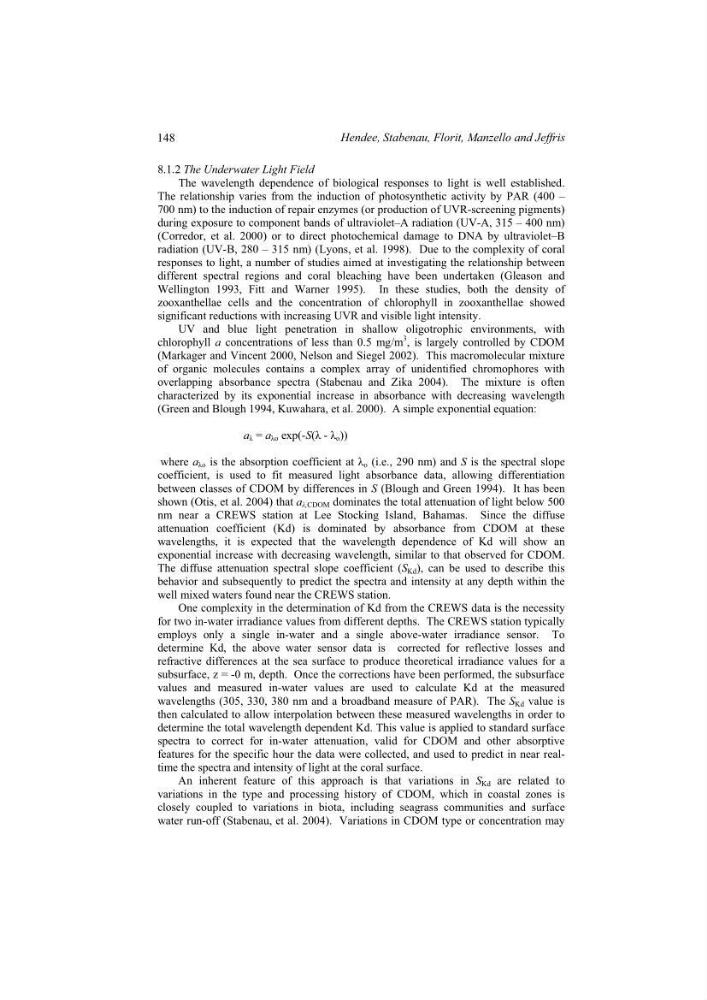
(Green and Blough 1994, Kuwahara, et al. 2000). A simple exponential equation:
a Ȝ = a Ȝo exp(-S(Ȝ - Ȝ o ))
where a Ȝo is the absorption coefficient at Ȝ o (i.e., 290 nm) and S is the spectral slope
coefficient, is used to fit measured light absorbance data, allowing differentiation
between classes of CDOM by differences in S (Blough and Green 1994). It has been
shown (Otis, et al. 2004) that a Ȝ,CDOM dominates the total attenuation of light below 500
nm near a CREWS station at Lee Stocking Island, Bahamas. Since the diffuse
attenuation coefficient (Kd) is dominated by absorbance from CDOM at these
wavelengths, it is expected that the wavelength dependence of Kd will show an
exponential increase with decreasing wavelength, similar to that observed for CDOM.
The diffuse attenuation spectral slope coefficient (S Kd ), can be used to describe this
behavior and subsequently to predict the spectra and intensity at any depth within the
well mixed waters found near the CREWS station.
One complexity in the determination of Kd from the CREWS data is the necessity
for two in-water irradiance values from different depths. The CREWS station typically
employs only a single in-water and a single above-water irradiance sensor. To
determine Kd, the above water sensor data is corrected for reflective losses and
refractive differences at the sea surface to produce theoretical irradiance values for a
subsurface, z = -0 m, depth. Once the corrections have been performed, the subsurface
values and measured in-water values are used to calculate Kd at the measured
wavelengths (305, 330, 380 nm and a broadband measure of PAR). The S Kd value is
then calculated to allow interpolation between these measured wavelengths in order to
determine the total wavelength dependent Kd. This value is applied to standard surface
spectra to correct for in-water attenuation, valid for CDOM and other absorptive
features for the specific hour the data were collected, and used to predict in near realtime the spectra and intensity of light at the coral surface.
An inherent feature of this approach is that variations in S Kd are related to
variations in the type and processing history of CDOM, which in coastal zones is
closely coupled to variations in biota, including seagrass communities and surface
water run-off (Stabenau, et al. 2004). Variations in CDOM type or concentration may
148
Hendee, Stabenau, Florit, Manzello and Jeffris