

f APAR is derived through VI relationships and LUE is scaled down with
meteorological information available, normally, at much coarser resolution. In the
BIOME-BGC (BioGeochemical Cycles) model, biome specific LUE max values are
scaled down using meteorological data (Running et al. 2004). Net Primary Productivity (NPP) has been modeled with AVHRR-NDVI inputs to the NASACASA (Carnegie Ames Stanford Approach) model, and more recently, Potter et al.
(2007) found monthly EVI inputs to the CASA model significantly improved both
predicted high- and low-seasonal carbon fluxes, associated with peak growing
season uptake rates of CO 2 in irrigated croplands and moist temperate forests.
There is also much interest in estimating GPP solely with remote sensing
methods in order to avoid the large uncertainties in LUE estimates based on land
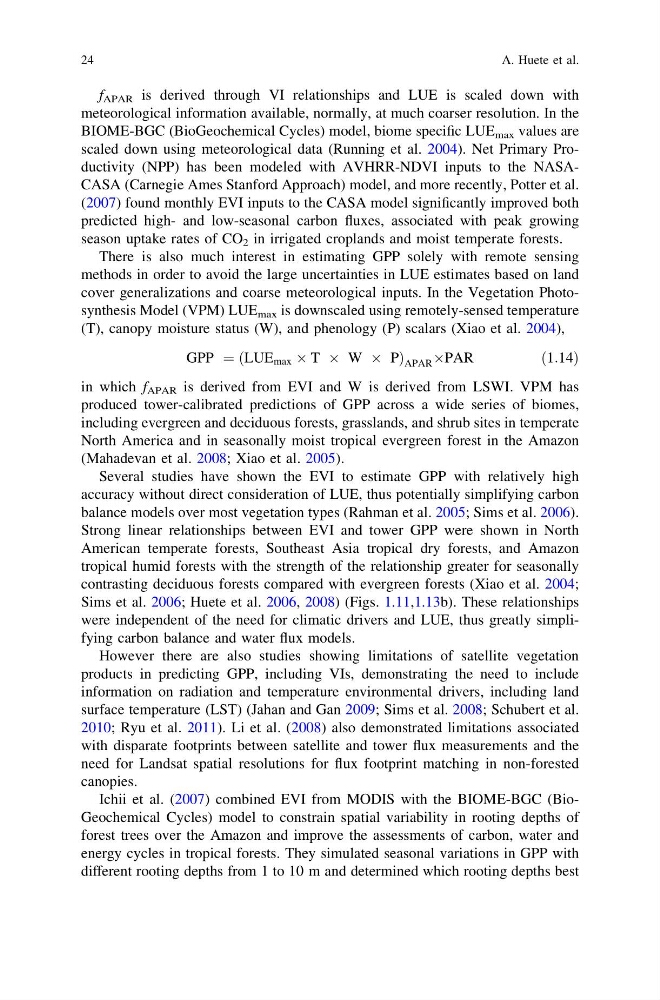
cover generalizations and coarse meteorological inputs. In the Vegetation Photosynthesis Model (VPM) LUE max is downscaled using remotely-sensed temperature
(T), canopy moisture status (W), and phenology (P) scalars (Xiao et al. 2004),
GPP ¼ LUE max  T  W  P
ð
Þ APAR ÂPAR
ð1:14Þ
in which f APAR is derived from EVI and W is derived from LSWI. VPM has
produced tower-calibrated predictions of GPP across a wide series of biomes,
including evergreen and deciduous forests, grasslands, and shrub sites in temperate
North America and in seasonally moist tropical evergreen forest in the Amazon
(Mahadevan et al. 2008; Xiao et al. 2005).
Several studies have shown the EVI to estimate GPP with relatively high
accuracy without direct consideration of LUE, thus potentially simplifying carbon
balance models over most vegetation types (Rahman et al. 2005; Sims et al. 2006).
Strong linear relationships between EVI and tower GPP were shown in North
American temperate forests, Southeast Asia tropical dry forests, and Amazon
tropical humid forests with the strength of the relationship greater for seasonally
contrasting deciduous forests compared with evergreen forests (Xiao et al. 2004;
Sims et al. 2006; Huete et al. 2006, 2008) (Figs. 1.11,1.13b). These relationships
were independent of the need for climatic drivers and LUE, thus greatly simplifying carbon balance and water flux models.
However there are also studies showing limitations of satellite vegetation
products in predicting GPP, including VIs, demonstrating the need to include
information on radiation and temperature environmental drivers, including land
surface temperature (LST) (Jahan and Gan 2009; Sims et al. 2008; Schubert et al.
2010; Ryu et al. 2011). Li et al. (2008) also demonstrated limitations associated
with disparate footprints between satellite and tower flux measurements and the
need for Landsat spatial resolutions for flux footprint matching in non-forested
canopies.
Ichii et al. (2007) combined EVI from MODIS with the BIOME-BGC (BioGeochemical Cycles) model to constrain spatial variability in rooting depths of
forest trees over the Amazon and improve the assessments of carbon, water and
energy cycles in tropical forests. They simulated seasonal variations in GPP with
different rooting depths from 1 to 10 m and determined which rooting depths best
24
A. Huete et al.