

13.2. The Model
271
allocated to somatic (Gs) and gametic (Gg) growth, plus those lost as heat
in both resting/standard metabolism (Rs) and activity (Ra) . Based on the
laws of conservation of energy and mass this formula must always balance,
though determining its absolute values may prove difficult.
We used Fish Bioenergetics 3.0 (Hewett and johnson 1992) to determine
the energy partition pattern for the two growth scenarios of Nile perch (see
Hewett and johnson (992) for a discussion of the technique and Kitchell et
al. (997) for the specific assumptions and data used for Nile perch). From
these functions we calculated the weight specific metabolic rates for both
scenarios in the form of a simple allometric function
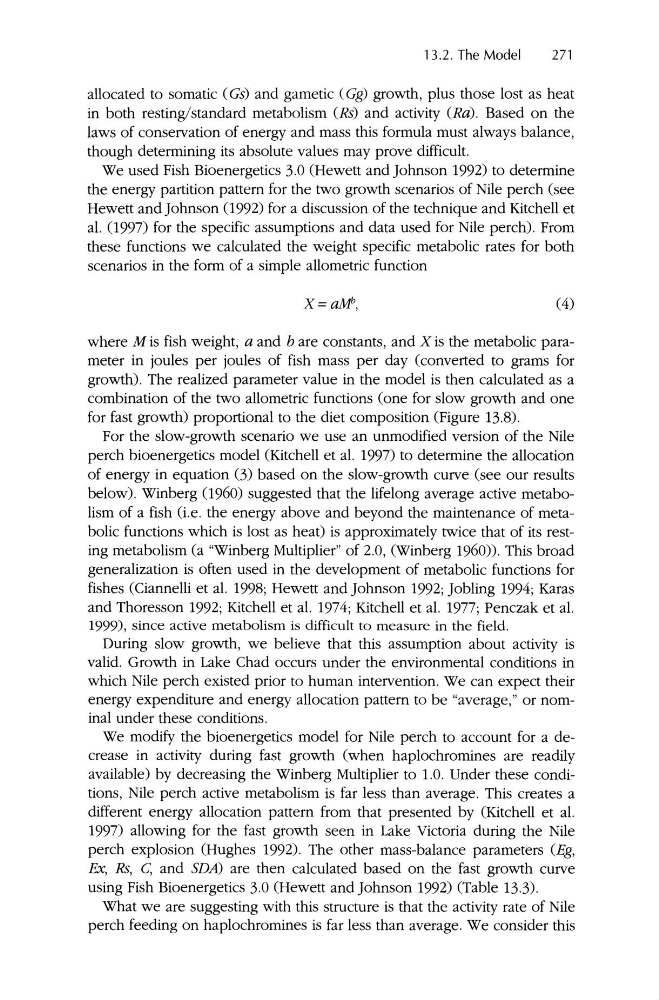
X=aM,
(4)
where M is fish weight, a and b are constants, and X is the metabolic parameter in joules per joules of fish mass per day (converted to grams for
growth). The realized parameter value in the model is then calculated as a
combination of the two allometric functions (one for slow growth and one
for fast growth) proportional to the diet composition (Figure 13.8).
For the slow-growth scenario we use an unmodified version of the Nile
perch bioenergetics model (Kitchell et al. 1997) to determine the allocation
of energy in equation (3) based on the slow-growth curve (see our results
below). Winberg (960) suggested that the lifelong average active metabolism of a fish (i.e . the energy above and beyond the maintenance of metabolic functions which is lost as heat) is approximately twice that of its resting metabolism (a "Winberg Multiplier" of 2.0, (Winberg 1960)). This broad
generalization is often used in the development of metabolic functions for
fishes (Ciannelli et al. 1998; Hewett and johnson 1992; jobling 1994; Karas
and Thoresson 1992; Kitchell et al. 1974; Kitchell et al. 1977; Penczak et al.
1999), since active metabolism is difficult to measure in the field .
During slow growth, we believe that this assumption about activity is
valid. Growth in Lake Chad occurs under the environmental conditions in
which Nile perch existed prior to human intervention. We can expect their
energy expenditure and energy allocation pattern to be "average ," or nominal under these conditions.
We modify the bioenergetics model for Nile perch to account for a decrease in activity during fast growth (when haplochromines are readily
available) by decreasing the Winberg Multiplier to 1.0. Under these conditions, Nile perch active metabolism is far less than average. This creates a
different energy allocation pattern from that presented by (Kitchell et al.
1997) allowing for the fast growth seen in Lake Victoria during the Nile
perch explosion (Hughes 1992). The other mass-balance parameters (Eg,
Ex, Rs, C, and SDA) are then calculated based on the fast growth curve
using Fish Bioenergetics 3.0 (Hewett and johnson 1992) (Table 13.3).
What we are suggesting with this structure is that the activity rate of Nile
perch feeding on haplochromines is far less than average. We consider this