

373
sure have also been discussed in this context (for a comprehensive overview of the
potential interpretation, see the discussions in Deng et al. 2011 , 2013 ).
In several additional groups of euteleostomorph fi shes, ancillary auditory structures evolved. Anabantiformes (labyrinth fi shes) possess suprabranchial airbreathing organs that are located close to the saccules. The macula sacculi shows
the opposing pattern of ciliary bundle orientation, while the maculae utriculi and
lagenae have “standard” patterns (Fig. 4b ). These fi shes have improved auditory
abilities, detecting frequencies up to 4 kHz (Schneider 1942 ; Ladich and Yan 1998 ).
In this group, it is assumed that the ancillary auditory structures primarily evolved
for air-breathing, enabling the fi sh to inhabit freshwaters with low oxygen concentrations, and that improved hearing was a by-product of this development (Ladich
and Popper 2001 ).
Members of the Etroplinae (Cichliformes, Cichlidae) and some members of the
Sciaenidae ( Micropogonias undulates , Cynoscion nebulosus , Bairdiella chrysoura ;
order incertae sedis) and Chaetodontidae (genus Chaetodon ; Chaetodontiformes)
display anterior swim bladder extensions approaching or contacting the ears
(Ramcharitar et al. 2001 ; Webb et al. 2001 ; Ramcharitar et al. 2004 ; Webb et al.
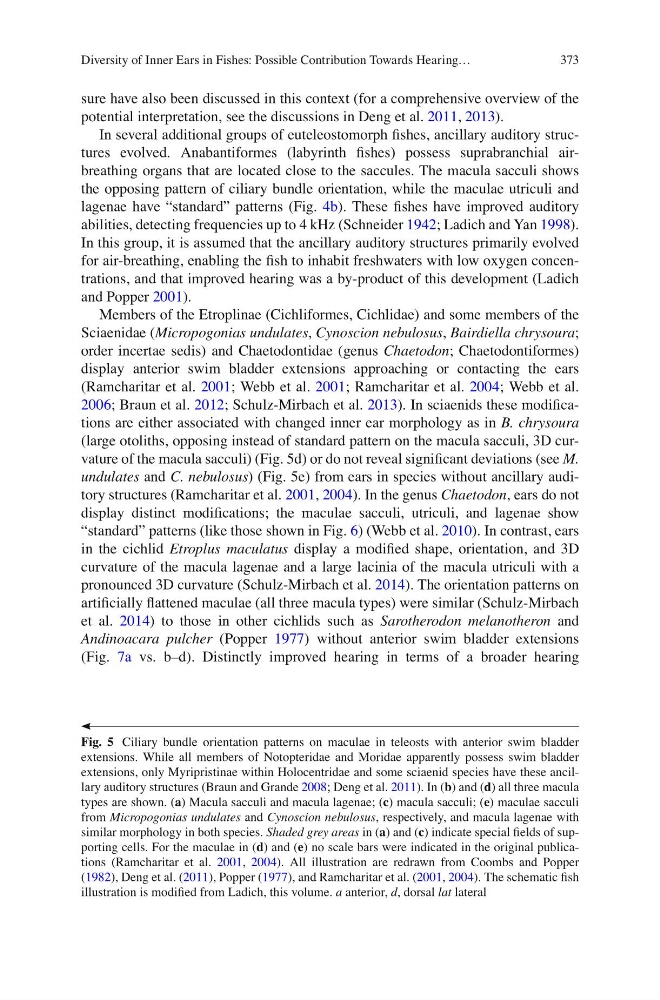
2006 ; Braun et al. 2012 ; Schulz-Mirbach et al. 2013 ). In sciaenids these modifi cations are either associated with changed inner ear morphology as in B. chrysoura
(large otoliths, opposing instead of standard pattern on the macula sacculi, 3D curvature of the macula sacculi) (Fig. 5d ) or do not reveal signifi cant deviations (see M.
undulates and C. nebulosus ) (Fig. 5e ) from ears in species without ancillary auditory structures (Ramcharitar et al. 2001 , 2004 ). In the genus Chaetodon , ears do not
display distinct modifi cations; the maculae sacculi, utriculi, and lagenae show
“standard” patterns (like those shown in Fig. 6 ) (Webb et al. 2010 ). In contrast, ears
in the cichlid Etroplus maculatus display a modifi ed shape, orientation, and 3D
curvature of the macula lagenae and a large lacinia of the macula utriculi with a
pronounced 3D curvature (Schulz-Mirbach et al. 2014 ). The orientation patterns on
artifi cially fl attened maculae (all three macula types) were similar (Schulz-Mirbach
et al. 2014 ) to those in other cichlids such as Sarotherodon melanotheron and
Andinoacara pulcher (Popper 1977 ) without anterior swim bladder extensions
(Fig. 7a vs. b–d). Distinctly improved hearing in terms of a broader hearing
Fig. 5 Ciliary bundle orientation patterns on maculae in teleosts with anterior swim bladder
extensions. While all members of Notopteridae and Moridae apparently possess swim bladder
extensions, only Myripristinae within Holocentridae and some sciaenid species have these ancillary auditory structures (Braun and Grande 2008 ; Deng et al. 2011 ). In ( b ) and ( d ) all three macula
types are shown. ( a ) Macula sacculi and macula lagenae; ( c ) macula sacculi; ( e ) maculae sacculi
from Micropogonias undulates and Cynoscion nebulosus , respectively, and macula lagenae with
similar morphology in both species. Shaded grey areas in ( a ) and ( c ) indicate special fi elds of supporting cells. For the maculae in ( d ) and ( e ) no scale bars were indicated in the original publications (Ramcharitar et al. 2001 , 2004 ). All illustration are redrawn from Coombs and Popper
( 1982 ), Deng et al. ( 2011 ), Popper ( 1977 ), and Ramcharitar et al. ( 2001 , 2004 ). The schematic fi sh
illustration is modifi ed from Ladich, this volume. a anterior, d , dorsal lat lateral
Diversity of Inner Ears in Fishes: Possible Contribution Towards Hearing…