

109
ken surface are relatively quiet with a constant spectral peak at very low frequencies
(~30 Hz), regardless of fl ow velocity, water depth, or substrate composition (Lugli
and Fine 2003 ; Speares et al. 2011 ). However, when the water surface becomes
turbulent and air bubbles are trapped below the water surface, broadband spectral
energy emerges between 100 and 2000 Hz (Lugli and Fine 2003 ; Wysocki et al.
2007 ; Tonolla et al. 2009 , 2010 ). The frequency range of the second spectral peak is
variable, but does not typically overlap with the low frequency peak of the unbroken
surface waters, leaving a quiet window in a variety of freshwater and coastal habitats (Lugli and Fine 2003 ; Amoser and Ladich 2005 ; Wysocki et al. 2007 ; Tonolla
et al. 2010 ). Shallow coastal habitats can generate similar low frequency quiet windows (Lugli 2010 ; but see Coers et al. 2008 ). Sources of ambient noise in freshwater
and shallow marine habitats are reviewed in more detail by others (Shellert and
Popper 1992; Myrberg and Lugli 2006 ; Lugli 2010 ). Given the local variability in
ambient noise in freshwater habitats, further quantifi cation of relationships between
ambient noise spectra, sound spectra, and auditory sensitivity will advance our
understanding of the general question, “what are fi sh listening to” in their respective
environments, and to what extent masking has signifi cant effects on behaviour (Fay
and Popper 2012 ).
In addition to ambient noise, there is considerable transmission loss of low frequency sounds in shallow freshwater and coastal habitats, since sound energies are
well below the cutoff frequencies of most stream habitats (0.8 kHz for water depth
of 50 cm over a rigid bottom, Offi cer 1958 ; Rogers and Cox 1988 ). Field measurements of courtship sound transmission in Padogobius bonelli indicate an attenuation of 15–20 dB over 20 cm at depths of about 50 cm (Lugli and Fine 2003 , 2007 ),
which is more rapid decay than spherical or cylindrical spreading. The result is
small active spaces for acoustic communication, with sound production often occurring when individuals are within decimeters of each other.
Absolute sound levels measured close to the fi sh (i.e. within 10 cm) are 110–125
dB dB re 1 μPa for Cottus species (Ladich 1989 ; Colleye et al. 2013 ), 100–138 for
gobies (Lugli et al. 1995 , 1997 ; Lindström and Lugli 2000 ; Stadler 2002 ), and
80–90 dB for darters (Speares et al. 2011 ). Signal-to-noise ratios within the quiet
window were 40 dB greater than average environmental noise levels in the stony
stream habitats of P. nigricans and P. bonelli and 50 dB greater for Knipowitschia
punctatissma residing in spring habitats (Lugli 2010). In darters, Speares et al.
( 2011 ) found a 20–30 dB difference between the ambient noise and dominant
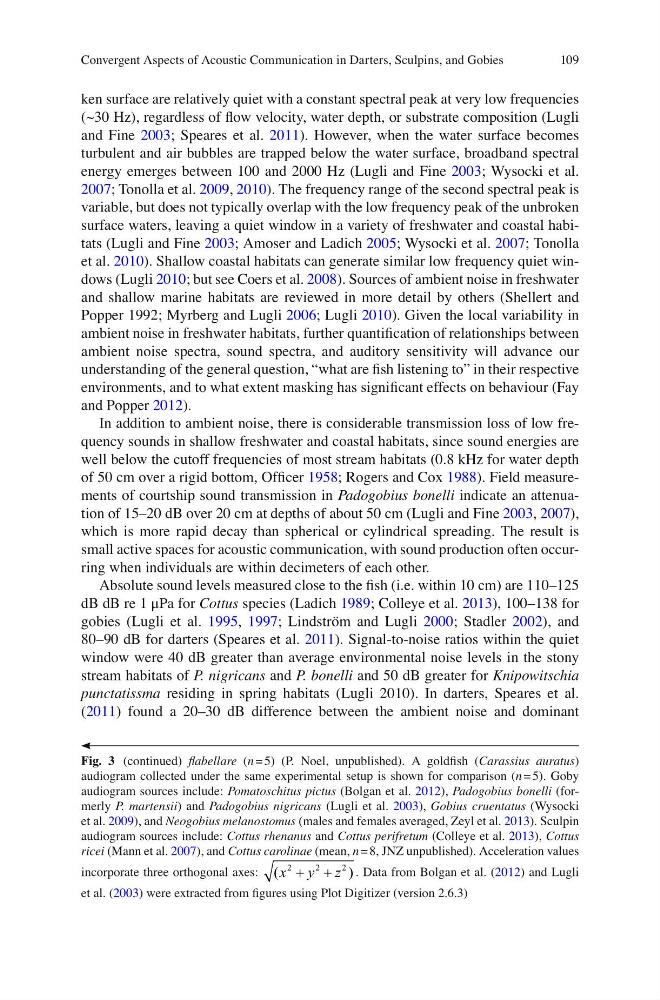
Fig. 3 (continued) fl abellare ( n = 5) (P. Noel, unpublished). A goldfi sh ( Carassius auratus )
audiogram collected under the same experimental setup is shown for comparison ( n = 5). Goby
audiogram sources include: Pomatoschitus pictus (Bolgan et al. 2012 ), Padogobius bonelli (formerly P. martensii ) and Padogobius nigricans (Lugli et al. 2003 ), Gobius cruentatus (Wysocki
et al. 2009 ), and Neogobius melanostomus (males and females averaged, Zeyl et al. 2013 ). Sculpin
audiogram sources include: Cottus rhenanus and Cottus perifretum (Colleye et al. 2013 ), Cottus
ricei (Mann et al. 2007 ), and Cottus carolinae (mean, n = 8, JNZ unpublished). Acceleration values
incorporate three orthogonal axes: (
)
x y z
2
2
2
+ +
. Data from Bolgan et al. ( 2012 ) and Lugli
et al. ( 2003 ) were extracted from fi gures using Plot Digitizer (version 2.6.3)
Convergent Aspects of Acoustic Communication in Darters, Sculpins, and Gobies