

42
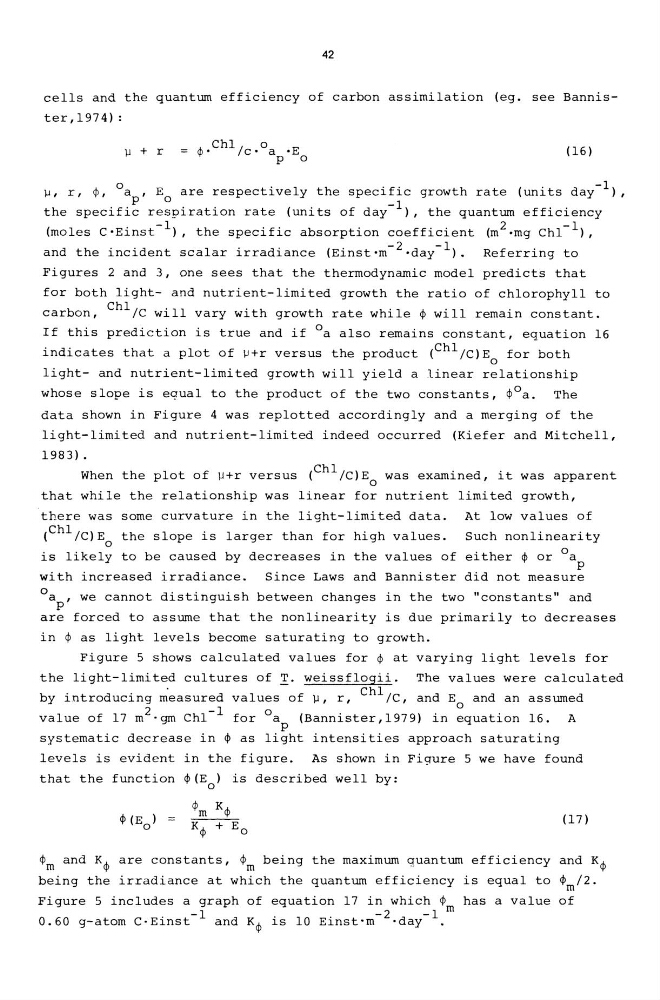
cells and the quantum efficiency of carbon assimilation (eg. see Bannister, 1974) :
)l + r
ChI
0
ep.
/c· a ·E
p 0
(16)
)1, r, ep, °a ,E are respectively the specific growth rate (units day-I),
p O l
the specific respiration rate (units of day- ), the quantum efficiency
(moles C.Einst- l ), the specific absorption coefficient (m 2 .mg Chl- l ),
and the incident scalar irradiance (Einst.m- 2 .day-l).
Referring to
Figures 2 and 3, one sees that the thermodynamic model predicts that
for both light- and nutrient-limited growth the ratio of chlorophyll to
carbon, Chl/c will vary with growth rate while ep will remain constant.
If this prediction is true and if °a also remains constant, equation 16
indicates that a plot of )l+r versus the product (Chl/C)E for both
o
light- and nutrient-limited growth will yield a linear relationship
whose slope is equal to the product of the two constants, epoa.
The
data shown in Figure 4 was replotted accordingly and a merging of the
light-limited and nutrient-limited indeed occurred (Kiefer and Mitchell,
1983) .
When the plot of )l+r versus (Chl/C)E o was examined, it was apparent
that while the relationship was linear for nutrient limited growth,
there was some curvature in the light-limited data.
(Chl/C)E the slope is larger than for high values.
o
is likely to be caused by decreases in the values of
with increased irradiance.
Since Laws and Bannister
At low values of
Such nonlinearity
either ep or °a
p
did not measure
°a p ' we cannot distinguish between changes in the two "constants" and
are forced to assume that the nonlinearity is due primarily to decreases
in ep as light levels become saturating to growth.
Figure 5 shows calculated values for ep at varying light levels for
the light-limited cultures of !. weissflogii. The values were calculated
by introducing ~easured values of )1, r, Chl/C , and E and an assumed
o
value of 17 m 2 .gm Chl- l for oa p (Bannister,1979) in equation 16. A
systematic decrease in ep as light intensities approach saturating
levels is evident in the figure.
As shown in Figure 5 we have found
that the function ep(E o ) is described well by:
ep(E o ) =
epm Kep
(17)
Kep + Eo
¢m and Kep are constants, ¢m being the maximum quantum efficiency and Kep
being the irradiance at which the quantum efficiency is equal to epm/2.
Figure 5 includes a graph of equation 17 in which epm has a value of
-1
-2
-1
0.60 g-atom C·Einst
and K¢ is 10 Einst·m ·day