

214
cD..O.
c:: 0
C~E
Q) Q)
(ij;;:o
.~"O E
::J>.
O":!:: E
W32r.o
E •
::J ~
..c::
-
cD 'e/)
c:: ON
Q) c:: •
-coE CO_
> 0 _
.- ::J 0
::J "0 E
O"c::
Wo~
0 ......
C)
cD..-. CO e/)
....
c::~
o E
. .
co- .... 0
'0.. E
~ E
~W
I40
30
20
10
0.6
0.4
0.2
10
5
LR. Cowan
cP~OOOO OOOOOCIDQJXP
r#
0
Cl)I)
CbOCboooooo 0 0 0 0 0 0 0 0 0
~
_ 0
•• • •••••
••
0
••
o
00
~,
00
00000
~o
#>
I~
herlox
1
8 0
air
0
00
CllQ
-
0
00000
• •
••••••
00
V rP
•••
..".",-.
100
200
300
400
Time, min
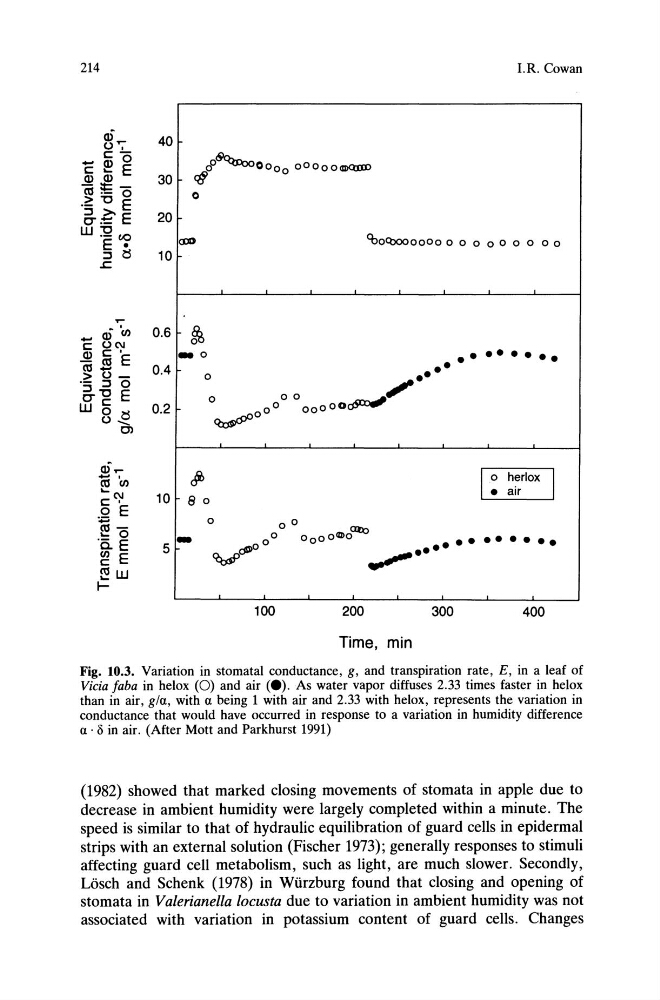
Fig. 10.3. Variation in stomatal conductance, g, and transpiration rate, E, in a leaf of
Vicia faba in helox (0) and air (e). As water vapor diffuses 2.33 times faster in helox
than in air, gla, with a being 1 with air and 2.33 with helox, represents the variation in
conductance that would have occurred in response to a variation in humidity difference
a . 0 in air. (After Mott and Parkhurst 1991)
(1982) showed that marked closing movements of stomata in apple due to
decrease in ambient humidity were largely completed within a minute. The
speed is similar to that of hydraulic equilibration of guard cells in epidermal
strips with an external solution (Fischer 1973); generally responses to stimuli
affecting guard cell metabolism, such as light, are much slower. Secondly,
Losch and Schenk (1978) in Wiirzburg found that closing and opening of
stomata in Valerianella locusta due to variation in ambient humidity was not
associated with variation in potassium content of guard cells. Changes
cD..O.
c:: 0
C~E
Q) Q)
(ij;;:o
.~"O E
::J>.
O":!:: E
W32r.o
E •
::J ~
..c::
-
cD 'e/)
c:: ON
Q) c:: •
-coE CO_
> 0 _
.- ::J 0
::J "0 E
O"c::
Wo~
0 ......
C)
cD..-. CO e/)
....
c::~
o E
. .
co- .... 0
'0.. E
~ E
~W
I40
30
20
10
0.6
0.4
0.2
10
5
LR. Cowan
cP~OOOO OOOOOCIDQJXP
r#
0
Cl)I)
CbOCboooooo 0 0 0 0 0 0 0 0 0
~
_ 0
•• • •••••
••
0
••
o
00
~,
00
00000
~o
#>
I~
herlox
1
8 0
air
0
00
CllQ
-
0
0000
• •
••••••
00
V rP
•••
..".",-.
100
200
300
400
Time, min
Fig. 10.3. Variation in stomatal conductance, g, and transpiration rate, E, in a leaf of
Vicia faba in helox (0) and air (e). As water vapor diffuses 2.33 times faster in helox
than in air, gla, with a being 1 with air and 2.33 with helox, represents the variation in
conductance that would have occurred in response to a variation in humidity difference
a . 0 in air. (After Mott and Parkhurst 1991)
(1982) showed that marked closing movements of stomata in apple due to
decrease in ambient humidity were largely completed within a minute. The
speed is similar to that of hydraulic equilibration of guard cells in epidermal
strips with an external solution (Fischer 1973); generally responses to stimuli
affecting guard cell metabolism, such as light, are much slower. Secondly,
Losch and Schenk (1978) in Wiirzburg found that closing and opening of
stomata in Valerianella locusta due to variation in ambient humidity was not
associated with variation in potassium content of guard cells. Changes