

“dissolution residue.” The association of biogenic Ba,
opal, and biogenic sedimentation has been described by
many authors (see reviews in Schmitz, 1987; Gingele
et al., 1999). These observations have opened the potential
to use biogenic barium downcore distributions as an
important proxy for paleoproductivity, given that both
organic carbon and opal may suffer from remineralization
and dissolution. An important step in quantifying past productivity is to establish the relationship between biogenic
barium and organic carbon in sediment traps (Dymond
et al., 1992; Francois et al., 1995). Using algorithms developed from empirical observations, downcore variations in
biogenic barium flux have been converted to paleoprimary production. This approach has a number of
assumptions and potential drawbacks. In particular, it is
necessary to calculate the biogenic component of the total
barium content in the sediment. This is usually achieved
by normalization to lithogenic metals such as aluminum
or titanium. There may be additional sources of barium
to the sediment from hydrothermal systems or benthic
organisms such as xenophyophores. Finally, although barite is very refractory under oxic conditions, during sulfate
reduction in anaerobic sediments, barite dissolution may
occur.
Bibliography
Bishop, J. K. B., 1988. The barite-opal-organic-carbon association
in oceanic particulate matter. Nature, 332, 341–343.
Calvert, S. E., and Price, N. B., 1983. Geochemistry of Namibian
shelf sediments. In Suess, E., and Thiede, J. (eds.), Coastal
Upwelling, Part A. New York: Plenum, pp. 337–375.
Dehairs, F., Chesselet, R., and Jedwab, J., 1980. Discrete suspended
particles of barite and the barium cycle in the open ocean. Earth
and Planetary Science Letters, 49, 528–550.
Dymond, J., 1981. Geochemistry of Nazca plate surface sediments:
an evaluation of hydrothermal, biogenic, detrital, and hydrogenous sources. Memoirs of the Geological Society of America,
154, 133–173.
Dymond, J., Suess, E., and Lyle, M., 1992. Barium in deep-sea sediment: a geochemical proxy for paleoproductivity. Paleoceanography, 7(2), 163–181.
Francois, R., Honjo, S., Manganini, S. J., and Ravizza, G. E., 1995.
Biogenic barium fluxes to the deep-sea: implications for
paleoproductivity reconstruction. Global Biogeochemical
Cycles, 9, 289–303.
Gingele, F. X., Zabel, M., Kasten, S., Bonn, W. J., and Nurnberg,
C. C., 1999. Biogenic barium as a proxy for paleoproductivity:
methods and limitations of application. In Fischer, G., and
Wefer, G. (eds.), Use of Proxies in Paleoceanography. Berlin:
Springer, pp. 345–364.
Revelle, R., Bramelette, M., Arrenhius, G., and Goldberg, E. D.,
1955. Pelagic sediments of the Pacific. Geological Society of
America, Special Paper, 62, 221–235.
Schmitz, B., 1987. Barium, high productivity, and northward wandering of the Indian continent. Paleoceanography, 2, 63–77.
Shimmield, G. B., 1992. Can sediment geochemistry record
changes in coastal upwelling paleoproductivity? Evidence from
northwest Africa and the Arabian Sea. In Summerhayes, C.,
Prell, W., and Emeis, K. (eds.), Upwelling Systems Since the
Early Miocene. London: Geological Society. Geology Society
Special Publication, Vol. 63, pp. 29–46.
BIOTURBATION
Gerhard Graf
Institute for Biological Sciences, University of Rostock,
Rostock, Germany
Definition
Bioturbation is the mixing and displacement of particles
in marine and freshwater sediments caused by benthic
fauna mainly during foraging and the construction of
burrows. As a result particulate proxies and microfossils
such as tests of foraminifera deposited at the seafloor
may not be found in the time slice corresponding to
its deposition, and the interpretation of the geological
record can be hampered. Other effects of animal activity,
such as biodeposition and bioresuspension, but also
fluid transport will not be considered in this section
although they are essential for biogeochemical cycles
and are used as subprocesses of bioturbation in recent biological literature (cf. Kristensen et al. 2012).
Measurement and modeling
In geological sciences, mainly natural radioactive tracers
like
210
Pb,
234
Th, or
7
Be but also chlorophyll a or stained
sand grains have been used for a quantitative description.
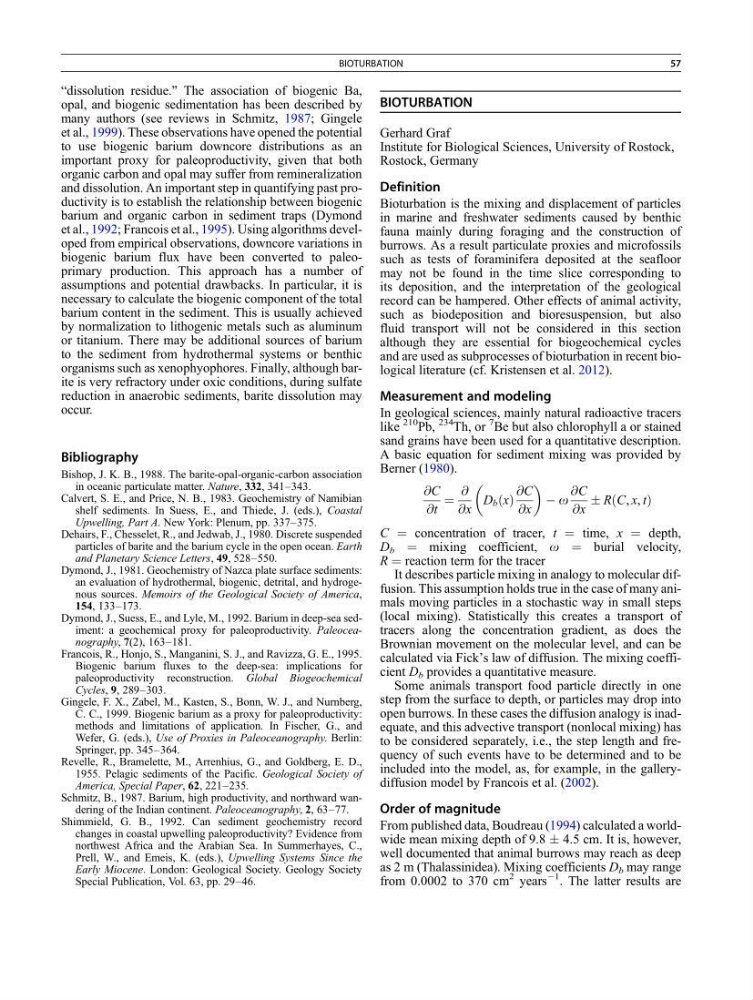
A basic equation for sediment mixing was provided by
Berner (1980).
@C
@t
¼
@
@x
D b x
ð Þ
@C
@x
À o
@C
@x
Æ R C, x, t
ð
Þ
C ¼ concentration of tracer, t ¼ time, x ¼ depth,
D b ¼ mixing coefficient, o ¼ burial velocity,
R ¼ reaction term for the tracer
It describes particle mixing in analogy to molecular diffusion. This assumption holds true in the case of many animals moving particles in a stochastic way in small steps
(local mixing). Statistically this creates a transport of
tracers along the concentration gradient, as does the
Brownian movement on the molecular level, and can be
calculated via Fick’s law of diffusion. The mixing coefficient D b provides a quantitative measure.
Some animals transport food particle directly in one
step from the surface to depth, or particles may drop into
open burrows. In these cases the diffusion analogy is inadequate, and this advective transport (nonlocal mixing) has
to be considered separately, i.e., the step length and frequency of such events have to be determined and to be
included into the model, as, for example, in the gallerydiffusion model by Francois et al. (2002).
Order of magnitude
From published data, Boudreau (1994) calculated a worldwide mean mixing depth of 9.8 Æ 4.5 cm. It is, however,
well documented that animal burrows may reach as deep
as 2 m (Thalassinidea). Mixing coefficients D b may range
from 0.0002 to 370 cm
2 years
À1 . The latter results are
BIOTURBATION
57