

173
Chapter eight: Fasting
and while providing critical insulation, its extent is generally far greater than required
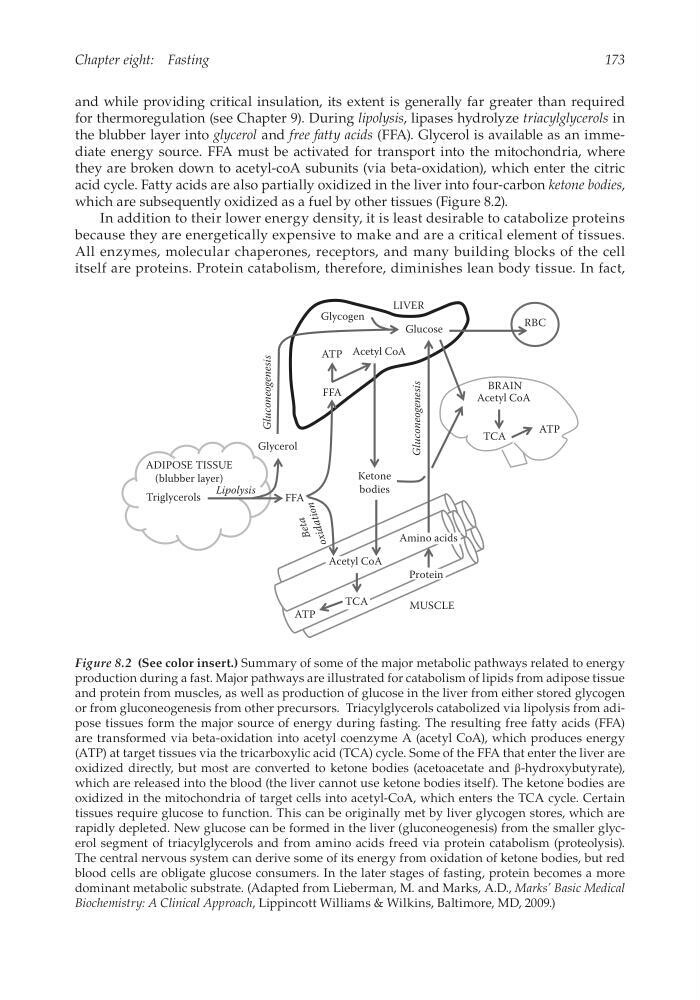
for thermoregulation (see Chapter 9). During lipolysis, lipases hydrolyze triacylglycerols in
the blubber layer into glycerol and free fatty acids (FFA). Glycerol is available as an immediate energy source. FFA must be activated for transport into the mitochondria, where
they are broken down to acetyl-coA subunits (via beta-oxidation), which enter the citric
acid cycle. Fatty acids are also partially oxidized in the liver into four-carbon ketone bodies,
which are subsequently oxidized as a fuel by other tissues (Figure 8.2).
In addition to their lower energy density, it is least desirable to catabolize proteins
because they are energetically expensive to make and are a critical element of tissues.
All enzymes, molecular chaperones, receptors, and many building blocks of the cell
itself are proteins. Protein catabolism, therefore, diminishes lean body tissue. In fact,
ATP
ATP
ATP
TCA
TCA
Glucose
Glycogen
Ketone
bodies
Glycerol
Lipolysis
B
e
ta
o
x
id
a
ti
o
n
Gluconeogenesis
Gluconeogenesis
Triglycerols
FFA
FFA
Acetyl CoA
Acetyl CoA
Acetyl CoA
MUSCLE
ADIPOSE TISSUE
(blubber layer)
BRAIN
LIVER
RBC
Amino acids
Protein
Figure 8.2 (See color insert.) Summary of some of the major metabolic pathways related to energy
production during a fast. Major pathways are illustrated for catabolism of lipids from adipose tissue
and protein from muscles, as well as production of glucose in the liver from either stored glycogen
or from gluconeogenesis from other precursors. Triacylglycerols catabolized via lipolysis from adipose tissues form the major source of energy during fasting. The resulting free fatty acids (FFA)
are transformed via beta-oxidation into acetyl coenzyme A (acetyl CoA), which produces energy
(ATP) at target tissues via the tricarboxylic acid (TCA) cycle. Some of the FFA that enter the liver are
oxidized directly, but most are converted to ketone bodies (acetoacetate and β-hydroxybutyrate),
which are released into the blood (the liver cannot use ketone bodies itself). The ketone bodies are
oxidized in the mitochondria of target cells into acetyl-CoA, which enters the TCA cycle. Certain
tissues require glucose to function. This can be originally met by liver glycogen stores, which are
rapidly depleted. New glucose can be formed in the liver (gluconeogenesis) from the smaller glycerol segment of triacylglycerols and from amino acids freed via protein catabolism (proteolysis).
The central nervous system can derive some of its energy from oxidation of ketone bodies, but red
blood cells are obligate glucose consumers. In the later stages of fasting, protein becomes a more
dominant metabolic substrate. (Adapted from Lieberman, M. and Marks, A.D., Marks’ Basic Medical
Biochemistry: A Clinical Approach, Lippincott Williams & Wilkins, Baltimore, MD, 2009.)