

Modeling Predator–Prey Dynamics
259
relevant parameters to be periodic functions of time. For example, we can
rewrite equation (8.1) with time-varying r or K:
dV /dt = rV [1 – V /K(t)] – P × F(V )
(8.3)
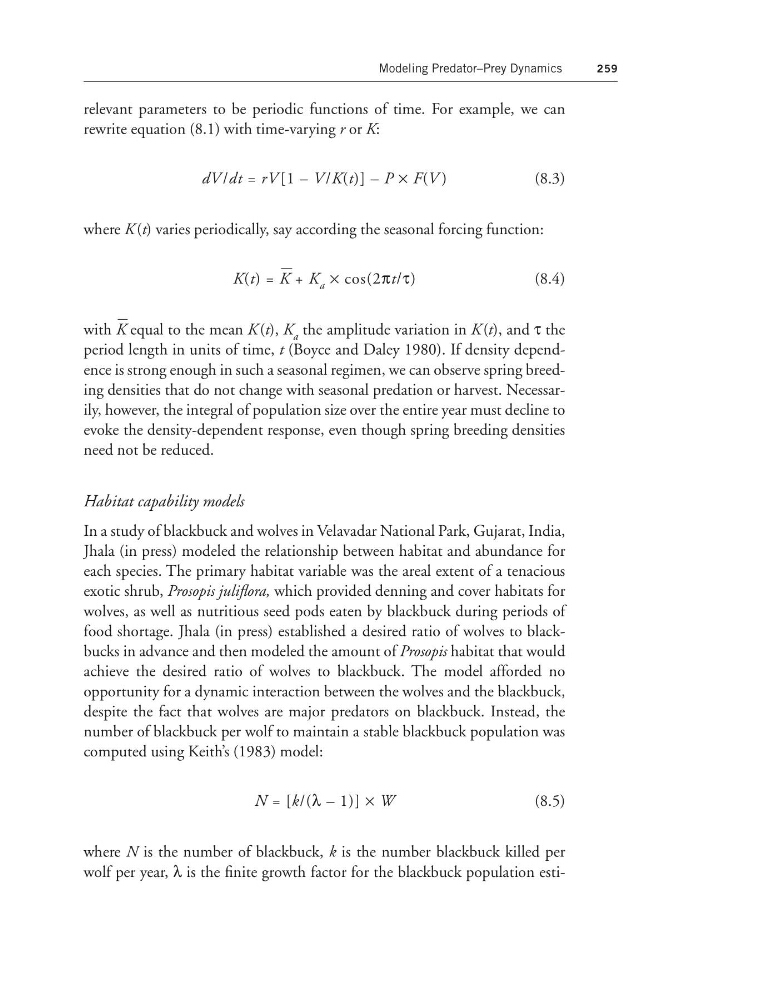
where K (t) varies periodically, say according the seasonal forcing function:
K(t) = K ෆ + K a × cos(2πt/τ)
(8.4)
with K ෆ equal to the mean K (t), K a the amplitude variation in K (t), and τ the
period length in units of time, t (Boyce and Daley 1980). If density dependence is strong enough in such a seasonal regimen, we can observe spring breeding densities that do not change with seasonal predation or harvest. Necessarily, however, the integral of population size over the entire year must decline to
evoke the density-dependent response, even though spring breeding densities
need not be reduced.
Habitat capability models
In a study of blackbuck and wolves in Velavadar National Park, Gujarat, India,
Jhala (in press) modeled the relationship between habitat and abundance for
each species. The primary habitat variable was the areal extent of a tenacious
exotic shrub, Prosopis juliflora, which provided denning and cover habitats for
wolves, as well as nutritious seed pods eaten by blackbuck during periods of
food shortage. Jhala (in press) established a desired ratio of wolves to blackbucks in advance and then modeled the amount of Prosopis habitat that would
achieve the desired ratio of wolves to blackbuck. The model afforded no
opportunity for a dynamic interaction between the wolves and the blackbuck,
despite the fact that wolves are major predators on blackbuck. Instead, the
number of blackbuck per wolf to maintain a stable blackbuck population was
computed using Keith’s (1983) model:
N = [k/(λ – 1)] × W
(8.5)
where N is the number of blackbuck, k is the number blackbuck killed per
wolf per year, λ is the finite growth factor for the blackbuck population esti-