

136
S. Yuvan and M. Bier
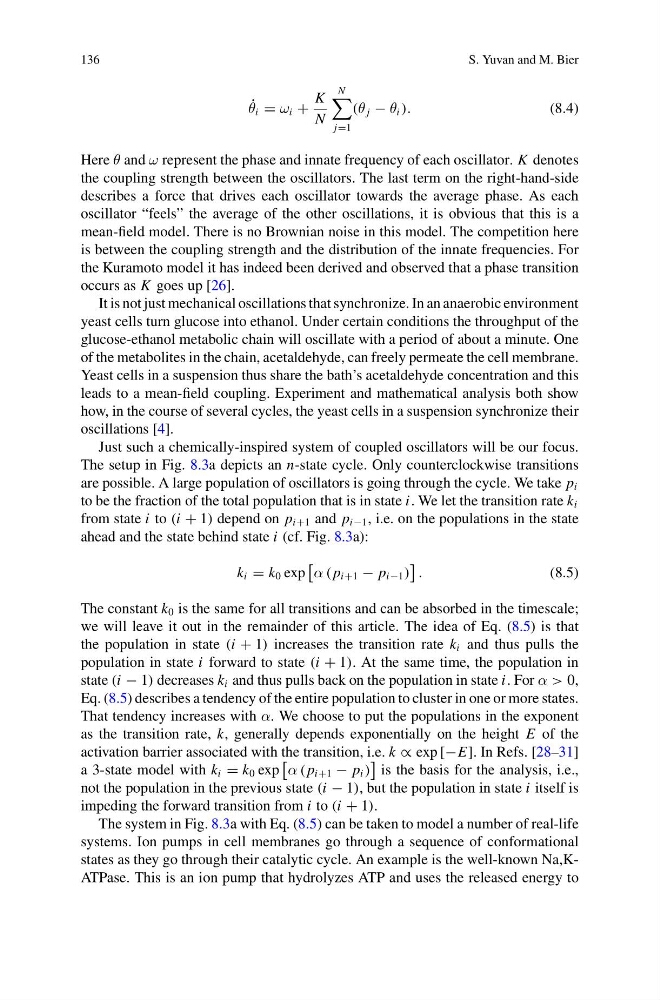
˙
θ i = ω i +
K
N
N
j=1
(θ j − θ i ).
(8.4)
Here θ and ω represent the phase and innate frequency of each oscillator. K denotes
the coupling strength between the oscillators. The last term on the right-hand-side
describes a force that drives each oscillator towards the average phase. As each
oscillator “feels” the average of the other oscillations, it is obvious that this is a
mean-field model. There is no Brownian noise in this model. The competition here
is between the coupling strength and the distribution of the innate frequencies. For
the Kuramoto model it has indeed been derived and observed that a phase transition
occurs as K goes up [26].
It is not just mechanical oscillations that synchronize. In an anaerobic environment
yeast cells turn glucose into ethanol. Under certain conditions the throughput of the
glucose-ethanol metabolic chain will oscillate with a period of about a minute. One
of the metabolites in the chain, acetaldehyde, can freely permeate the cell membrane.
Yeast cells in a suspension thus share the bath’s acetaldehyde concentration and this
leads to a mean-field coupling. Experiment and mathematical analysis both show
how, in the course of several cycles, the yeast cells in a suspension synchronize their
oscillations [4].
Just such a chemically-inspired system of coupled oscillators will be our focus.
The setup in Fig. 8.3a depicts an n-state cycle. Only counterclockwise transitions
are possible. A large population of oscillators is going through the cycle. We take p i
to be the fraction of the total population that is in state i. We let the transition rate k i
from state i to (i + 1) depend on p i+1 and p i−1 , i.e. on the populations in the state
ahead and the state behind state i (cf. Fig. 8.3a):
k i = k 0 exp
α ( p i+1 − p i−1 )
.
(8.5)
The constant k 0 is the same for all transitions and can be absorbed in the timescale;
we will leave it out in the remainder of this article. The idea of Eq. (8.5) is that
the population in state (i + 1) increases the transition rate k i and thus pulls the
population in state i forward to state (i + 1). At the same time, the population in
state (i − 1) decreases k i and thus pulls back on the population in state i. For α > 0,
Eq. (8.5) describes a tendency of the entire population to cluster in one or more states.
That tendency increases with α. We choose to put the populations in the exponent
as the transition rate, k, generally depends exponentially on the height E of the
activation barrier associated with the transition, i.e. k ∝ exp [−E]. In Refs. [28–31]
a 3-state model with k i = k 0 exp
α ( p i+1 − p i )
is the basis for the analysis, i.e.,
not the population in the previous state (i − 1), but the population in state i itself is
impeding the forward transition from i to (i + 1).
The system in Fig. 8.3a with Eq. (8.5) can be taken to model a number of real-life
systems. Ion pumps in cell membranes go through a sequence of conformational
states as they go through their catalytic cycle. An example is the well-known Na,KATPase. This is an ion pump that hydrolyzes ATP and uses the released energy to