

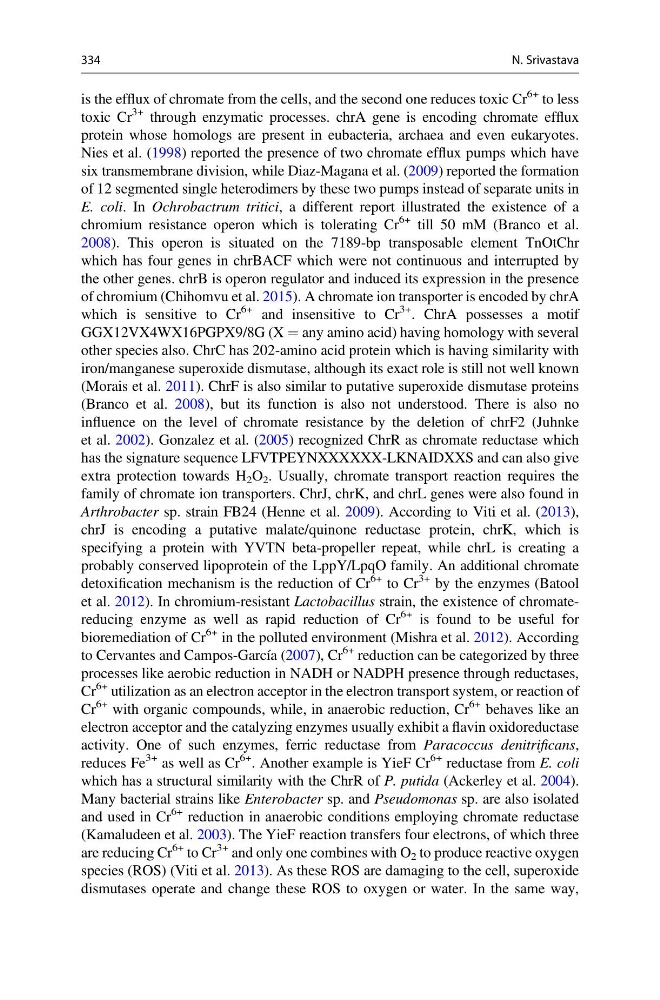
is the efflux of chromate from the cells, and the second one reduces toxic Cr
6+ to less
toxic Cr
3+ through enzymatic processes. chrA gene is encoding chromate efflux
protein whose homologs are present in eubacteria, archaea and even eukaryotes.
Nies et al. (1998) reported the presence of two chromate efflux pumps which have
six transmembrane division, while Diaz-Magana et al. (2009) reported the formation
of 12 segmented single heterodimers by these two pumps instead of separate units in
E. coli. In Ochrobactrum tritici, a different report illustrated the existence of a
chromium resistance operon which is tolerating Cr
6+ till 50 mM (Branco et al.
2008). This operon is situated on the 7189-bp transposable element TnOtChr
which has four genes in chrBACF which were not continuous and interrupted by
the other genes. chrB is operon regulator and induced its expression in the presence
of chromium (Chihomvu et al. 2015). A chromate ion transporter is encoded by chrA
which is sensitive to Cr
6+ and insensitive to Cr
3+ . ChrA possesses a motif
GGX12VX4WX16PGPX9/8G (X ¼ any amino acid) having homology with several
other species also. ChrC has 202-amino acid protein which is having similarity with
iron/manganese superoxide dismutase, although its exact role is still not well known
(Morais et al. 2011). ChrF is also similar to putative superoxide dismutase proteins
(Branco et al. 2008), but its function is also not understood. There is also no
influence on the level of chromate resistance by the deletion of chrF2 (Juhnke
et al. 2002). Gonzalez et al. (2005) recognized ChrR as chromate reductase which
has the signature sequence LFVTPEYNXXXXXX-LKNAIDXXS and can also give
extra protection towards H 2 O 2 . Usually, chromate transport reaction requires the
family of chromate ion transporters. ChrJ, chrK, and chrL genes were also found in
Arthrobacter sp. strain FB24 (Henne et al. 2009). According to Viti et al. (2013),
chrJ is encoding a putative malate/quinone reductase protein, chrK, which is
specifying a protein with YVTN beta-propeller repeat, while chrL is creating a
probably conserved lipoprotein of the LppY/LpqO family. An additional chromate
detoxification mechanism is the reduction of Cr
6+ to Cr
3+ by the enzymes (Batool
et al. 2012). In chromium-resistant Lactobacillus strain, the existence of chromatereducing enzyme as well as rapid reduction of Cr
6+ is found to be useful for
bioremediation of Cr
6+ in the polluted environment (Mishra et al. 2012). According
to Cervantes and Campos-García (2007), Cr
6+ reduction can be categorized by three
processes like aerobic reduction in NADH or NADPH presence through reductases,
Cr
6+ utilization as an electron acceptor in the electron transport system, or reaction of
Cr
6+ with organic compounds, while, in anaerobic reduction, Cr
6+ behaves like an
electron acceptor and the catalyzing enzymes usually exhibit a flavin oxidoreductase
activity. One of such enzymes, ferric reductase from Paracoccus denitrificans,
reduces Fe
3+ as well as Cr
6+ . Another example is YieF Cr
6+ reductase from E. coli
which has a structural similarity with the ChrR of P. putida (Ackerley et al. 2004).
Many bacterial strains like Enterobacter sp. and Pseudomonas sp. are also isolated
and used in Cr
6+ reduction in anaerobic conditions employing chromate reductase
(Kamaludeen et al. 2003). The YieF reaction transfers four electrons, of which three
are reducing Cr
6+ to Cr
3+ and only one combines with O 2 to produce reactive oxygen
species (ROS) (Viti et al. 2013). As these ROS are damaging to the cell, superoxide
dismutases operate and change these ROS to oxygen or water. In the same way,
334
N. Srivastava