

temperature does not affect this mode of resistance (Martinez et al. 2014; Doremus
et al. 2018). With warming, there may be selection for aphid clones, especially those
with endogenous anti-parasitoid protection, that carry thermally protective strains.
Another common protective symbiont in insects is Spiroplasma, which protects
Drosophila flies against parasitic nematodes and parasitoid wasps via the production
of variable RIP (ribosome-inactivating protein) toxins (Xie et al. 2010; Jaenike et al.
2010; Hamilton et al. 2016; Ballinger and Perlman 2017). A recent study found that
Spiroplasma protection against parasitoids performs better at cooler temperatures
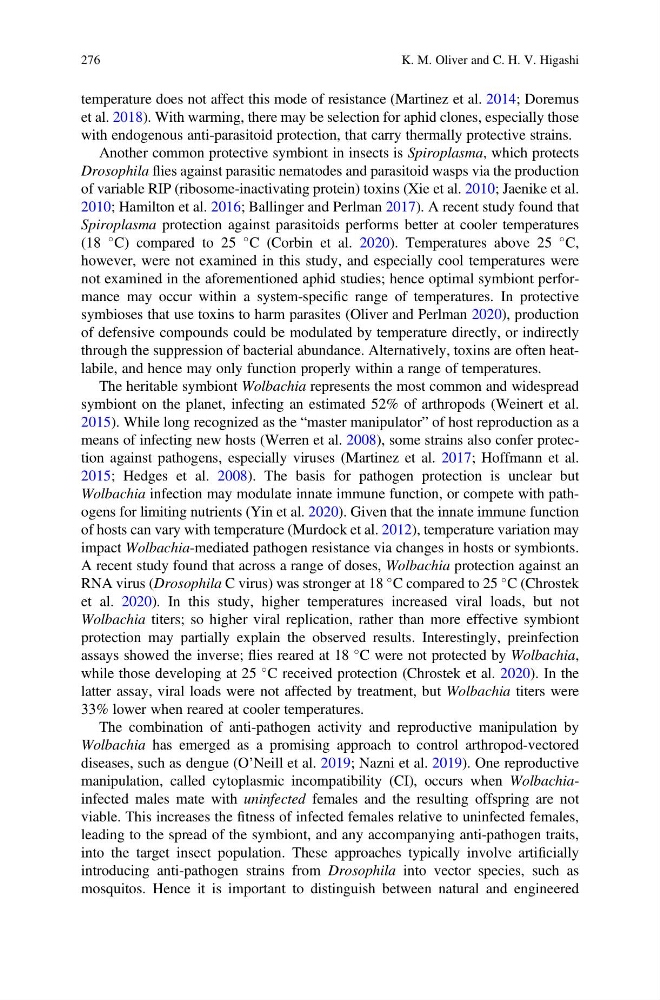
(18
C) compared to 25
C (Corbin et al. 2020). Temperatures above 25
C,
however, were not examined in this study, and especially cool temperatures were
not examined in the aforementioned aphid studies; hence optimal symbiont performance may occur within a system-specific range of temperatures. In protective
symbioses that use toxins to harm parasites (Oliver and Perlman 2020), production
of defensive compounds could be modulated by temperature directly, or indirectly
through the suppression of bacterial abundance. Alternatively, toxins are often heatlabile, and hence may only function properly within a range of temperatures.
The heritable symbiont Wolbachia represents the most common and widespread
symbiont on the planet, infecting an estimated 52% of arthropods (Weinert et al.
2015). While long recognized as the “master manipulator” of host reproduction as a
means of infecting new hosts (Werren et al. 2008), some strains also confer protection against pathogens, especially viruses (Martinez et al. 2017; Hoffmann et al.
2015; Hedges et al. 2008). The basis for pathogen protection is unclear but
Wolbachia infection may modulate innate immune function, or compete with pathogens for limiting nutrients (Yin et al. 2020). Given that the innate immune function
of hosts can vary with temperature (Murdock et al. 2012), temperature variation may
impact Wolbachia-mediated pathogen resistance via changes in hosts or symbionts.
A recent study found that across a range of doses, Wolbachia protection against an
RNA virus (Drosophila C virus) was stronger at 18
C compared to 25
C (Chrostek
et al. 2020). In this study, higher temperatures increased viral loads, but not
Wolbachia titers; so higher viral replication, rather than more effective symbiont
protection may partially explain the observed results. Interestingly, preinfection
assays showed the inverse; flies reared at 18
C were not protected by Wolbachia,
while those developing at 25
C received protection (Chrostek et al. 2020). In the
latter assay, viral loads were not affected by treatment, but Wolbachia titers were
33% lower when reared at cooler temperatures.
The combination of anti-pathogen activity and reproductive manipulation by
Wolbachia has emerged as a promising approach to control arthropod-vectored
diseases, such as dengue (O’Neill et al. 2019; Nazni et al. 2019). One reproductive
manipulation, called cytoplasmic incompatibility (CI), occurs when Wolbachiainfected males mate with uninfected females and the resulting offspring are not
viable. This increases the fitness of infected females relative to uninfected females,
leading to the spread of the symbiont, and any accompanying anti-pathogen traits,
into the target insect population. These approaches typically involve artificially
introducing anti-pathogen strains from Drosophila into vector species, such as
mosquitos. Hence it is important to distinguish between natural and engineered
276
K. M. Oliver and C. H. V. Higashi