

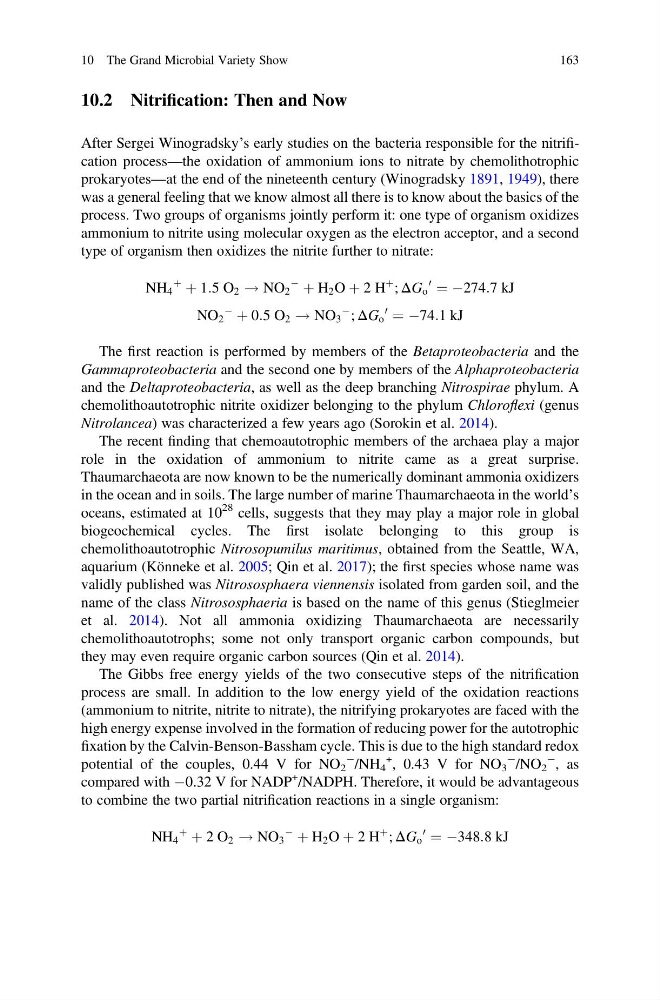
10.2 Nitrification: Then and Now
After Sergei Winogradsky’s early studies on the bacteria responsible for the nitrification process—the oxidation of ammonium ions to nitrate by chemolithotrophic
prokaryotes—at the end of the nineteenth century (Winogradsky 1891, 1949), there
was a general feeling that we know almost all there is to know about the basics of the
process. Two groups of organisms jointly perform it: one type of organism oxidizes
ammonium to nitrite using molecular oxygen as the electron acceptor, and a second
type of organism then oxidizes the nitrite further to nitrate:
NH 4
þ
þ 1:5 O 2 ! NO 2
À
þ H 2 O þ 2 H
þ ; ΔG o
0
¼ À274:7 kJ
NO 2
À
þ 0:5 O 2 ! NO 3
À ; ΔG o
0
¼ À74:1 kJ
The first reaction is performed by members of the Betaproteobacteria and the
Gammaproteobacteria and the second one by members of the Alphaproteobacteria
and the Deltaproteobacteria, as well as the deep branching Nitrospirae phylum. A
chemolithoautotrophic nitrite oxidizer belonging to the phylum Chloroflexi (genus
Nitrolancea) was characterized a few years ago (Sorokin et al. 2014).
The recent finding that chemoautotrophic members of the archaea play a major
role in the oxidation of ammonium to nitrite came as a great surprise.
Thaumarchaeota are now known to be the numerically dominant ammonia oxidizers
in the ocean and in soils. The large number of marine Thaumarchaeota in the world’s
oceans, estimated at 10
28 cells, suggests that they may play a major role in global
biogeochemical cycles. The first isolate belonging to this group is
chemolithoautotrophic Nitrosopumilus maritimus, obtained from the Seattle, WA,
aquarium (Könneke et al. 2005; Qin et al. 2017); the first species whose name was
validly published was Nitrososphaera viennensis isolated from garden soil, and the
name of the class Nitrososphaeria is based on the name of this genus (Stieglmeier
et al. 2014). Not all ammonia oxidizing Thaumarchaeota are necessarily
chemolithoautotrophs; some not only transport organic carbon compounds, but
they may even require organic carbon sources (Qin et al. 2014).
The Gibbs free energy yields of the two consecutive steps of the nitrification
process are small. In addition to the low energy yield of the oxidation reactions
(ammonium to nitrite, nitrite to nitrate), the nitrifying prokaryotes are faced with the
high energy expense involved in the formation of reducing power for the autotrophic
fixation by the Calvin-Benson-Bassham cycle. This is due to the high standard redox
potential of the couples, 0.44 V for NO 2
À
/NH 4
+
, 0.43 V for NO 3
À /NO 2
À
, as
compared with À0.32 V for NADP
+ /NADPH. Therefore, it would be advantageous
to combine the two partial nitrification reactions in a single organism:
NH 4
þ
þ 2 O 2 ! NO 3
À
þ H 2 O þ 2 H
þ ; ΔG o
0
¼ À348:8 kJ
10 The Grand Microbial Variety Show
163