

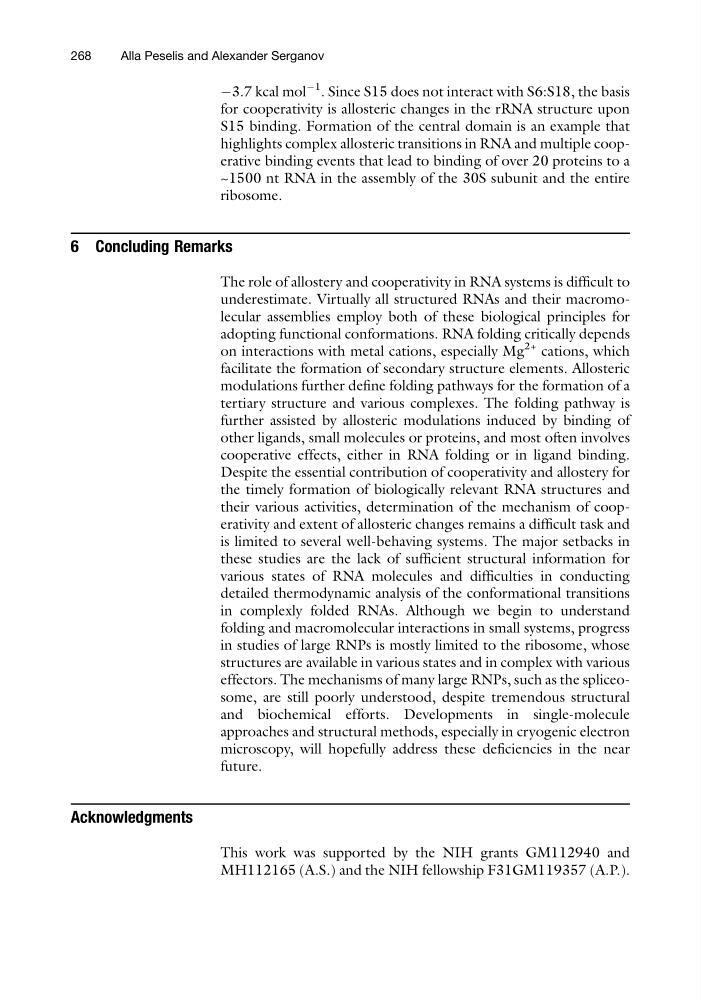
À3.7 kcal mol
À1 . Since S15 does not interact with S6:S18, the basis
for cooperativity is allosteric changes in the rRNA structure upon
S15 binding. Formation of the central domain is an example that
highlights complex allosteric transitions in RNA and multiple cooperative binding events that lead to binding of over 20 proteins to a
~1500 nt RNA in the assembly of the 30S subunit and the entire
ribosome.
6 Concluding Remarks
The role of allostery and cooperativity in RNA systems is difficult to
underestimate. Virtually all structured RNAs and their macromolecular assemblies employ both of these biological principles for
adopting functional conformations. RNA folding critically depends
on interactions with metal cations, especially Mg
2+ cations, which
facilitate the formation of secondary structure elements. Allosteric
modulations further define folding pathways for the formation of a
tertiary structure and various complexes. The folding pathway is
further assisted by allosteric modulations induced by binding of
other ligands, small molecules or proteins, and most often involves
cooperative effects, either in RNA folding or in ligand binding.
Despite the essential contribution of cooperativity and allostery for
the timely formation of biologically relevant RNA structures and
their various activities, determination of the mechanism of cooperativity and extent of allosteric changes remains a difficult task and
is limited to several well-behaving systems. The major setbacks in
these studies are the lack of sufficient structural information for
various states of RNA molecules and difficulties in conducting
detailed thermodynamic analysis of the conformational transitions
in complexly folded RNAs. Although we begin to understand
folding and macromolecular interactions in small systems, progress
in studies of large RNPs is mostly limited to the ribosome, whose
structures are available in various states and in complex with various
effectors. The mechanisms of many large RNPs, such as the spliceosome, are still poorly understood, despite tremendous structural
and biochemical efforts. Developments in single-molecule
approaches and structural methods, especially in cryogenic electron
microscopy, will hopefully address these deficiencies in the near
future.
Acknowledgments
This work was supported by the NIH grants GM112940 and
MH112165 (A.S.) and the NIH fellowship F31GM119357 (A.P.).
268
Alla Peselis and Alexander Serganov